Week 2 HW: DNA Design
This week focused on DNA Design — understanding how DNA can be organised into functional parts and combined to control how a biological system behaves.
Coming from design rather than biology, what interested me most was the shift in perspective: DNA is not only something to observe and understand, but something that can also be designed.
A simple genetic construct can be built from four main elements:
Promoter → RBS → CDS → Terminator
- Promoter — controls where transcription begins.
- RBS (Ribosome Binding Site) — influences how efficiently a protein is produced.
- CDS (Coding Sequence) — contains the DNA instructions for producing a protein.
- Terminator — signals the end of transcription.

Figure 1. Common components of a genetic circuit.
I found it useful to translate this into a language closer to design and manufacturing:
CONTROL → PRODUCTION INTENSITY → INSTRUCTION → STOP
Changing one part can change the behaviour of the whole system.
Genetic Circuits
When genetic parts are intentionally connected to control an output, they form a genetic circuit.
At its simplest:
INPUT → GENETIC CONTROL → GENE EXPRESSION → OUTPUT
The output might be a fluorescent protein, an enzyme or, eventually, part of a more complex biological production system.
This immediately made me think about my final project, Fashion Feeds on Pollution, where I am exploring whether methane-consuming microorganisms could eventually contribute to the production of a new biomaterial.
A very simplified version of the long-term system could look like:
Methane → Methanotroph → Biological Production → Extracellular Polymer → Material
This introduced a new question:
What if material production could eventually be switched on and controlled?
Before attempting that, however, I first needed to understand how a simple genetic circuit works.
Kernel
For DNA design we were introduced to Kernel, a platform for creating, assembling and simulating genetic constructs.
Kernel uses a parts-based approach to genetic design and can predict outputs such as RNA polymerase flux, ribosome flux and protein concentration.
For this exercise, the workflow became:
SEARCH → ASSEMBLE → SIMULATE → OBSERVE → REDESIGN
Part 1 — Learning the Basics
Creating My First Construct
I started by creating a new blank construct.
I initially called it:
Fashion Feeds on Pollution: Methane-Responsive Material Production Circuit
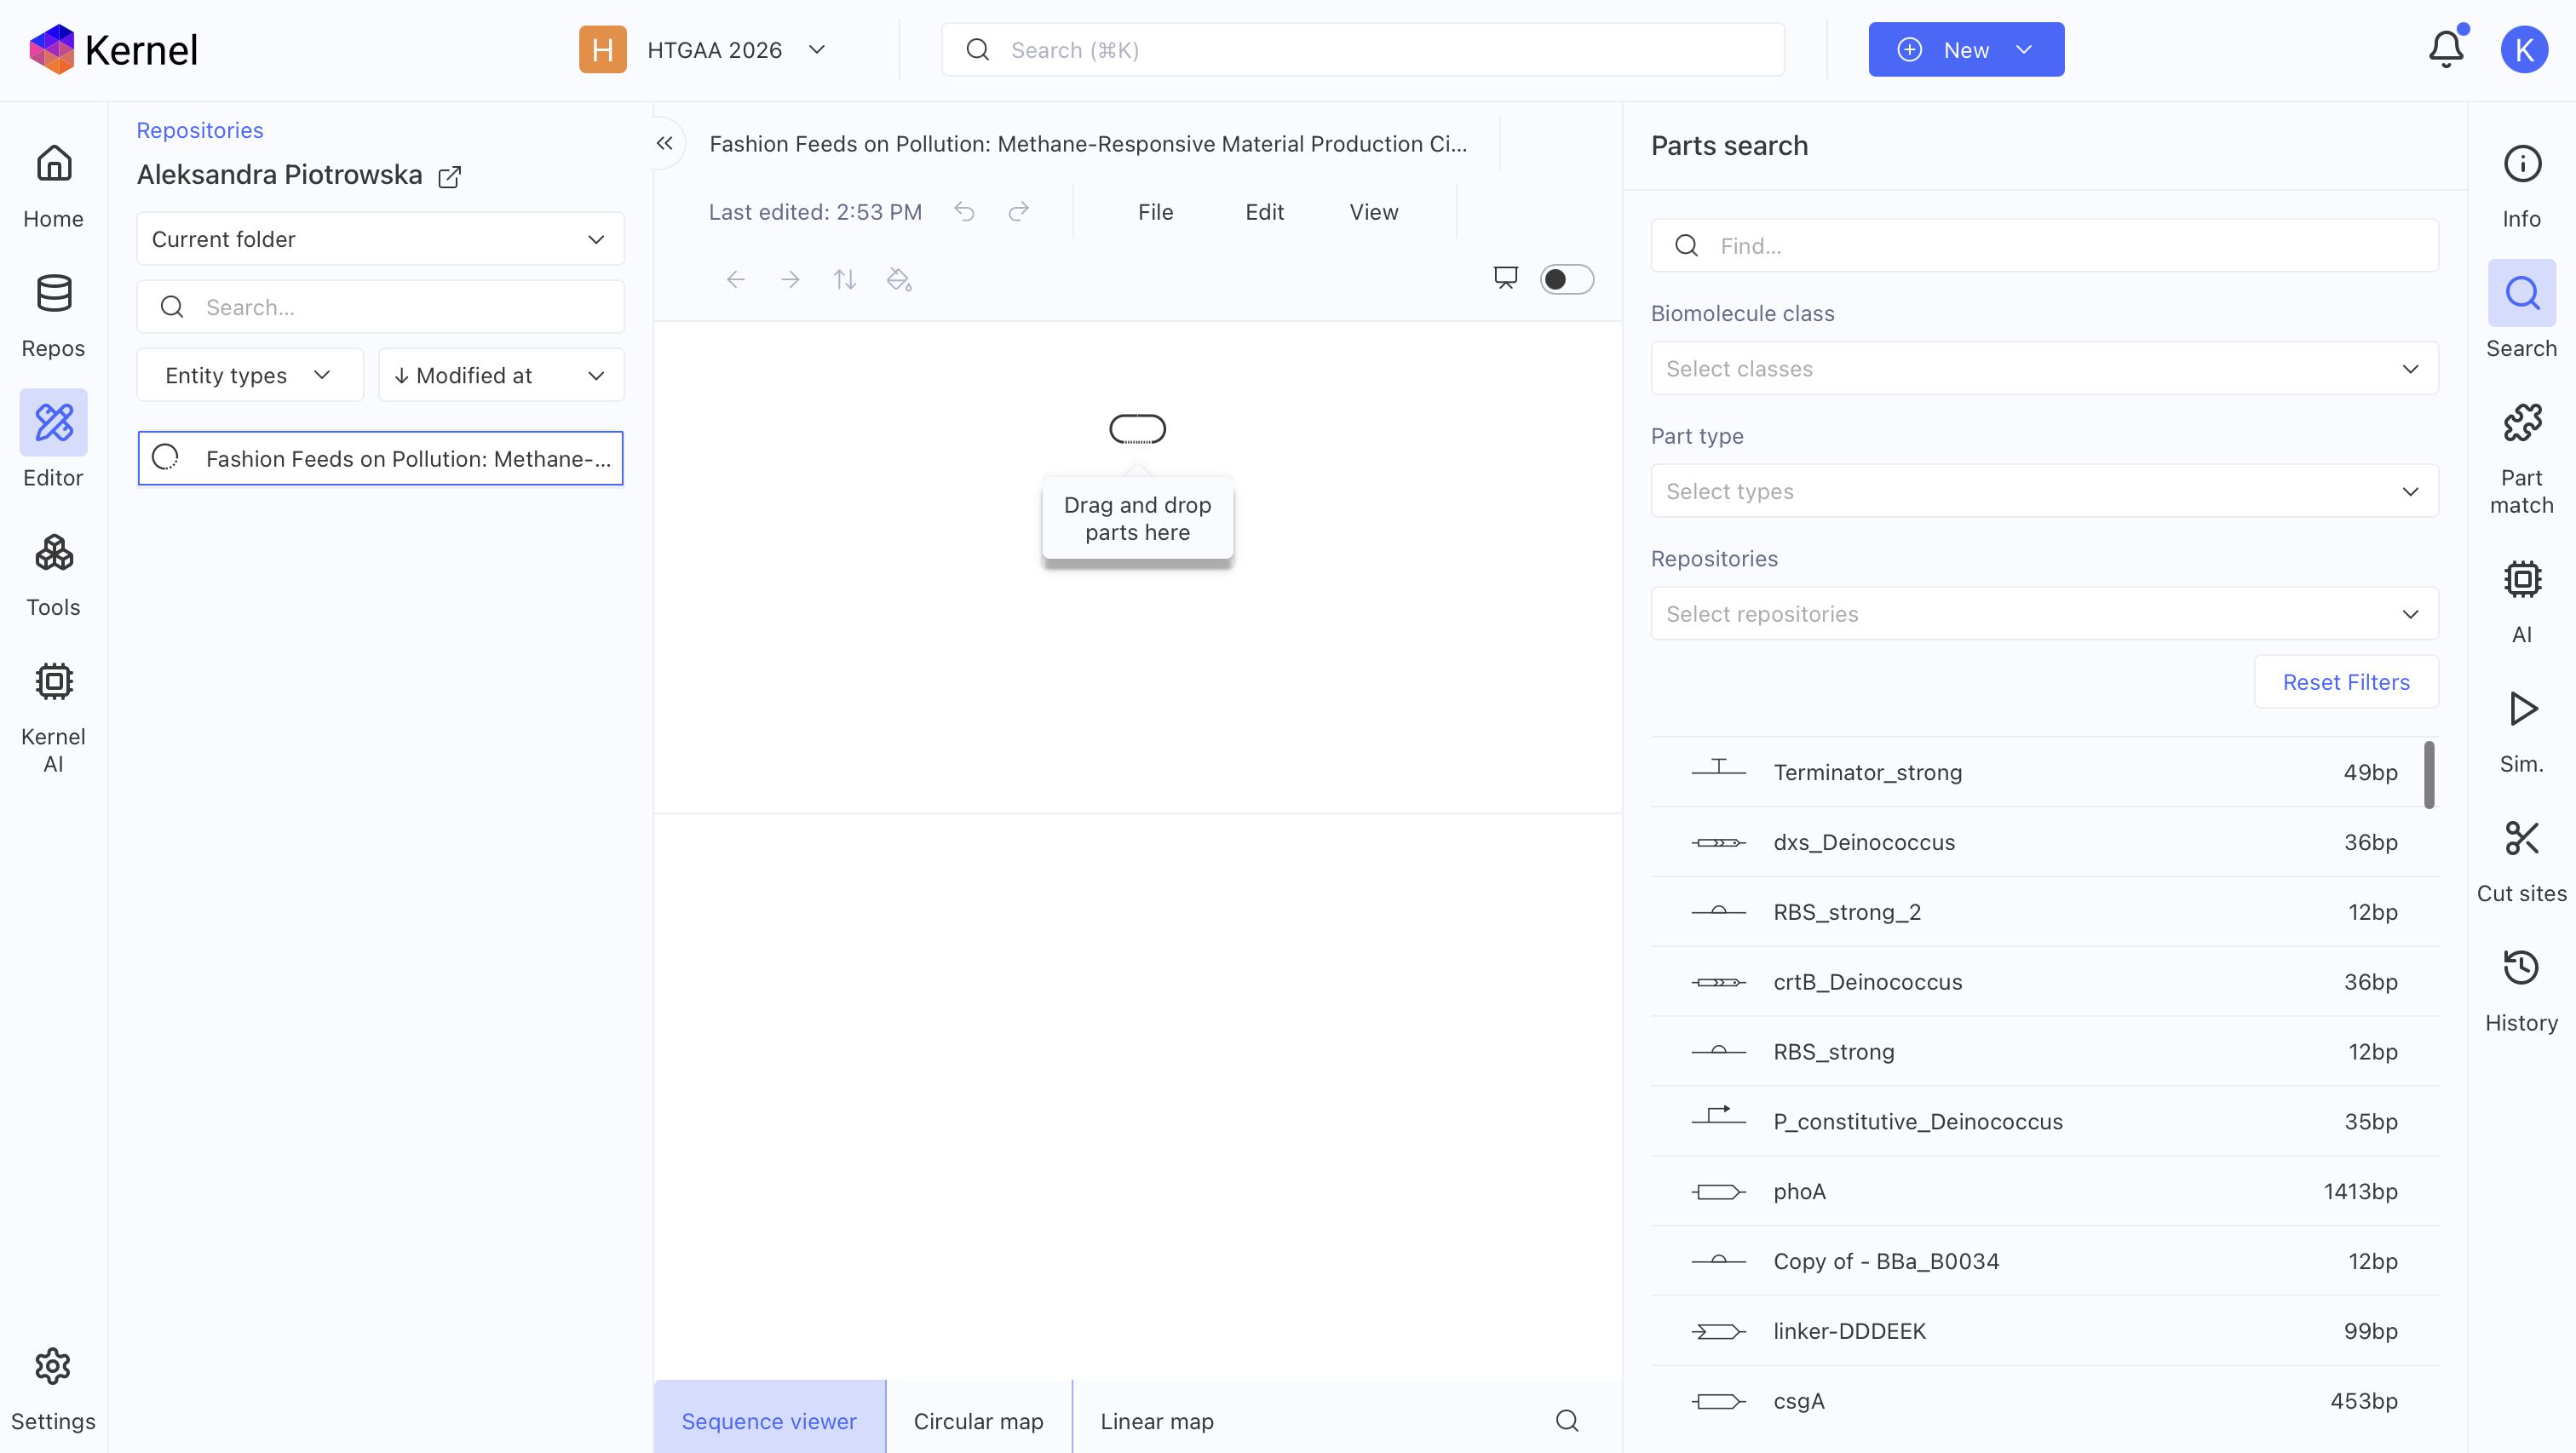
Figure 2. Creating my first blank construct in Kernel.
Although the name connected the exercise to my larger project, I quickly realised that this first circuit should remain much simpler.
Its purpose was to teach me the basic logic of DNA design before attempting a project-specific hypothesis.
Designing the Practice Circuit
For my first circuit I used the basic structure:
Promoter → RBS → Reporter CDS → Terminator
A reporter gene gives the circuit an output that can be measured or observed.
The first question was therefore simply:
Does the circuit behave in the way I expect?
before asking the much more complicated question:
Can biological production eventually be controlled?
1. Choosing a Promoter
The promoter is the first control point in the circuit.
It determines where transcription begins and can influence when a downstream gene is expressed.
Inside Kernel I searched for a characterised bacterial promoter.
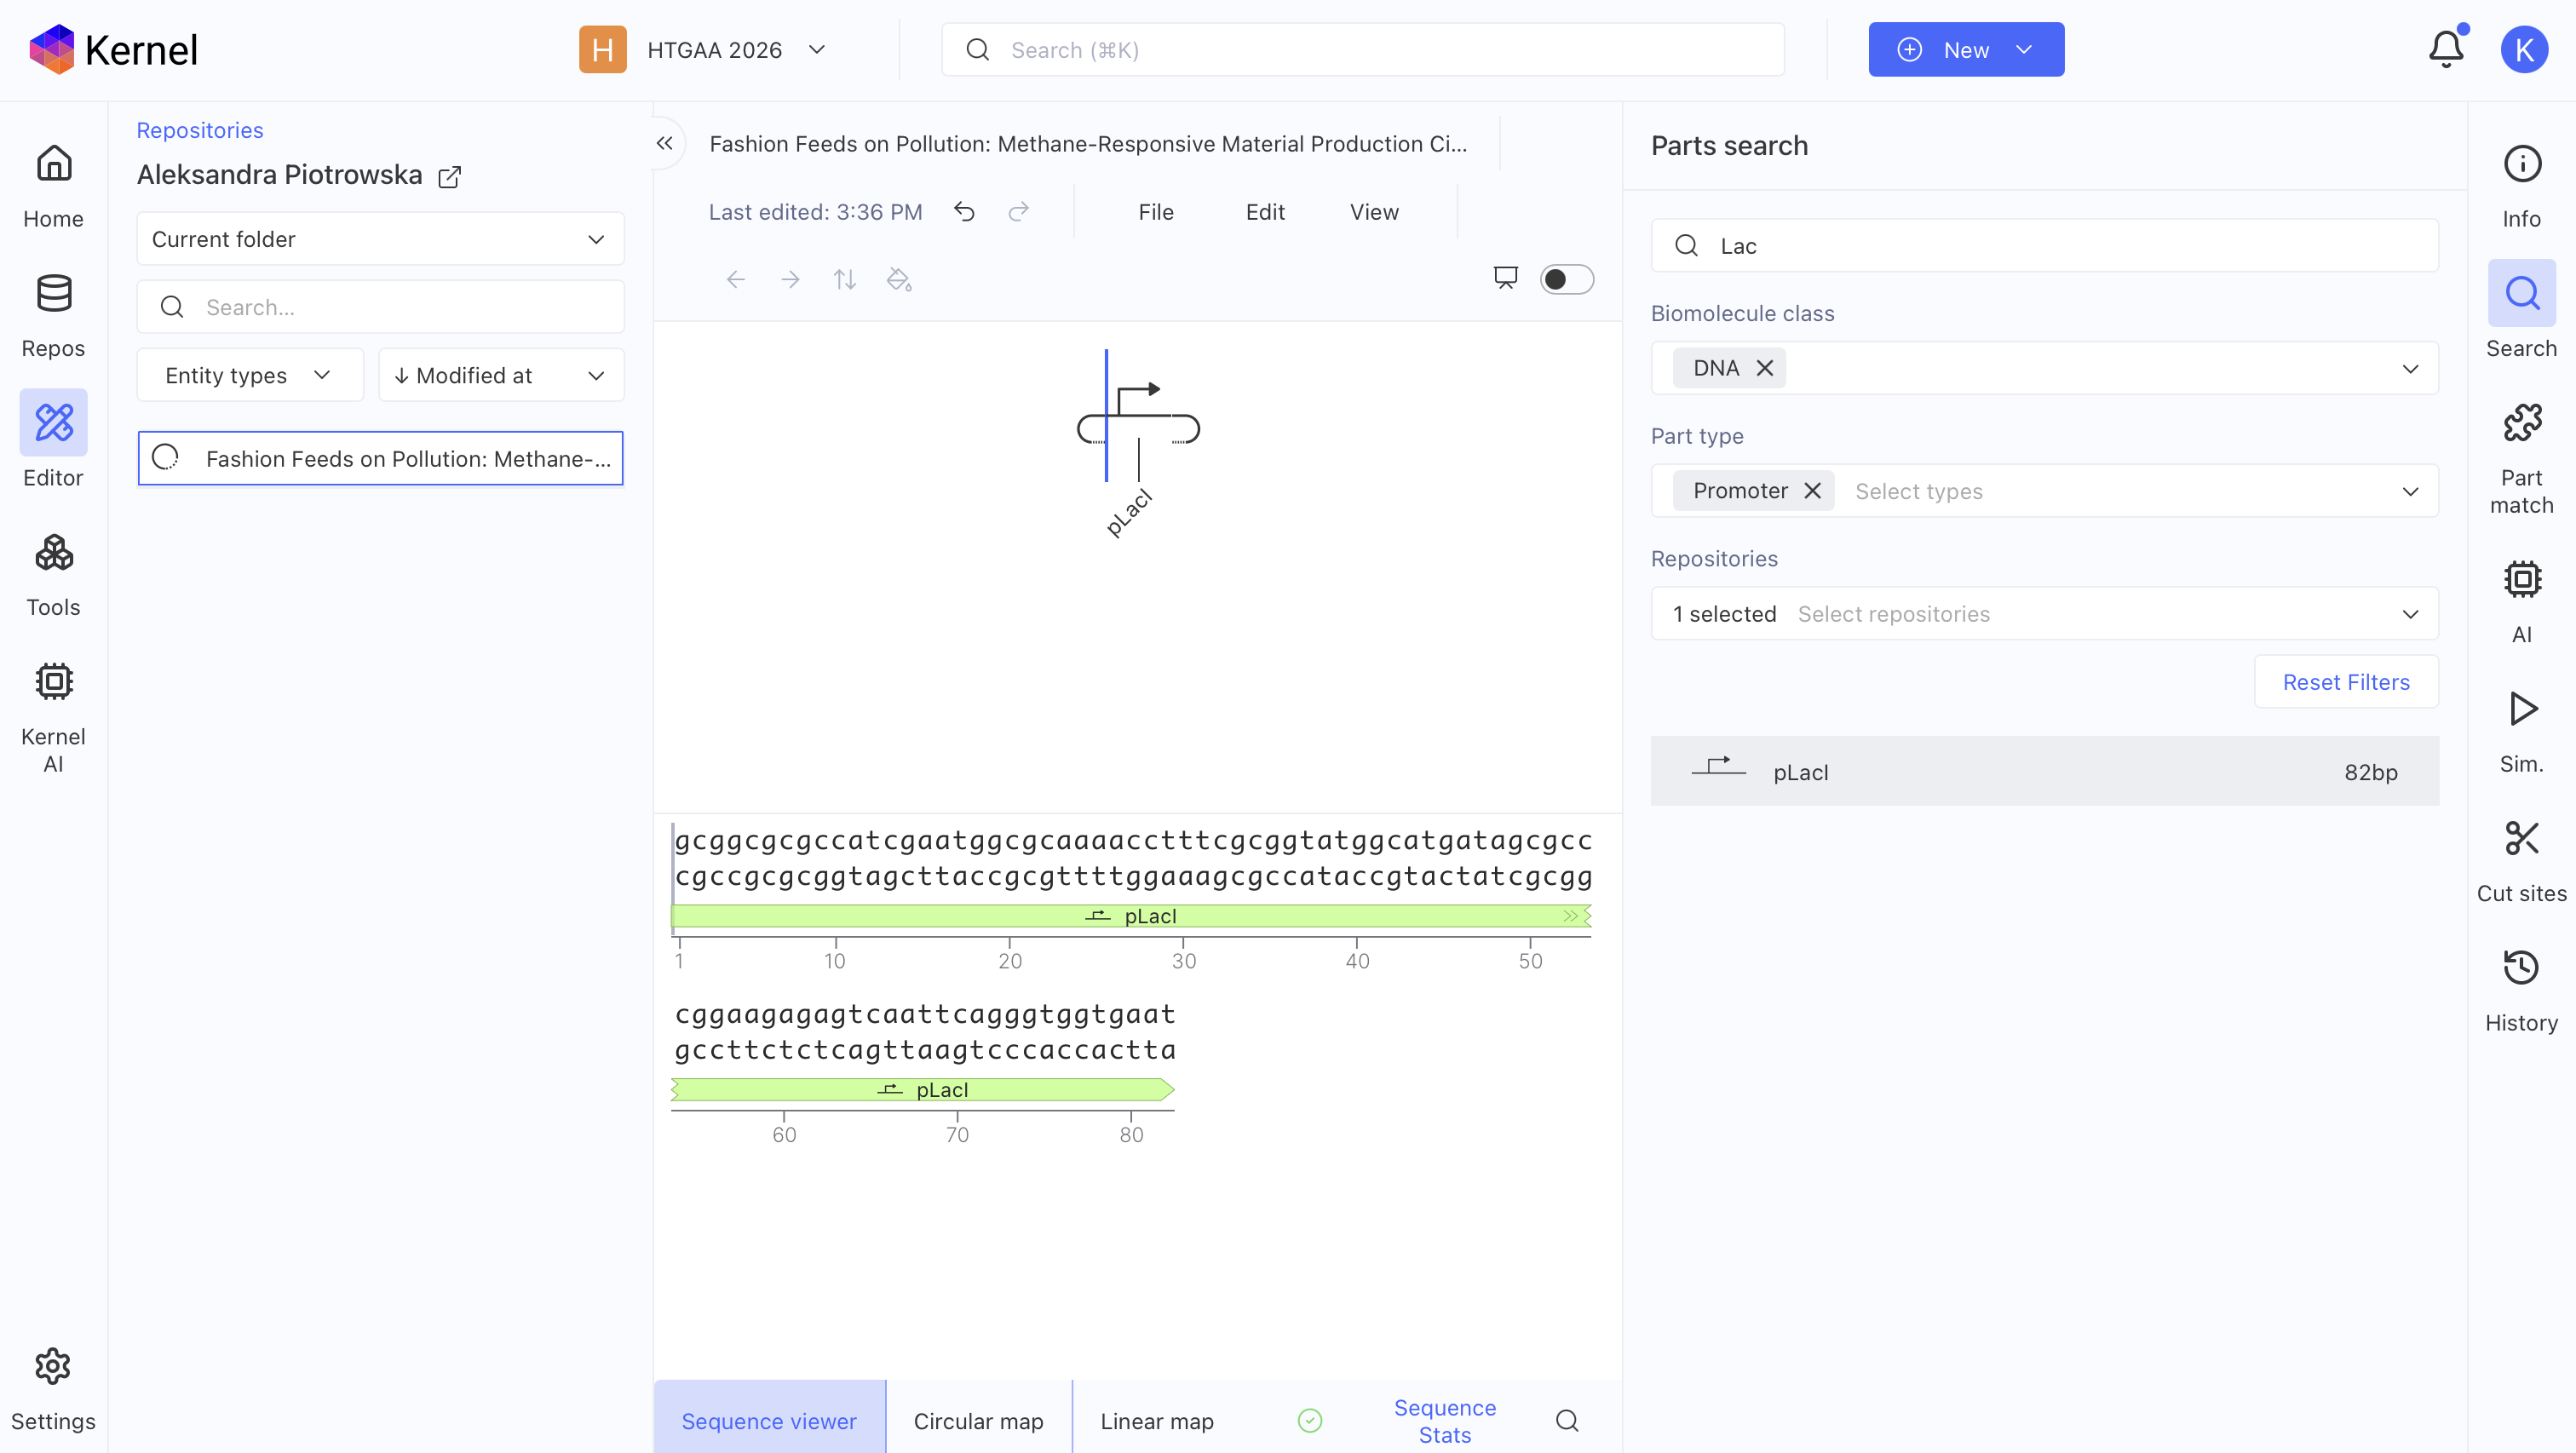
Figure 3. Selecting the characterised pLacI promoter in Kernel.
Selected promoter
pLacI
I chose a regulated promoter because I was already interested in the idea that biological production might eventually be controlled rather than permanently active.
2. Choosing an RBS
Next, I added a Ribosome Binding Site.
The RBS helps the ribosome recognise the mRNA and influences how efficiently the coding sequence is translated into protein.
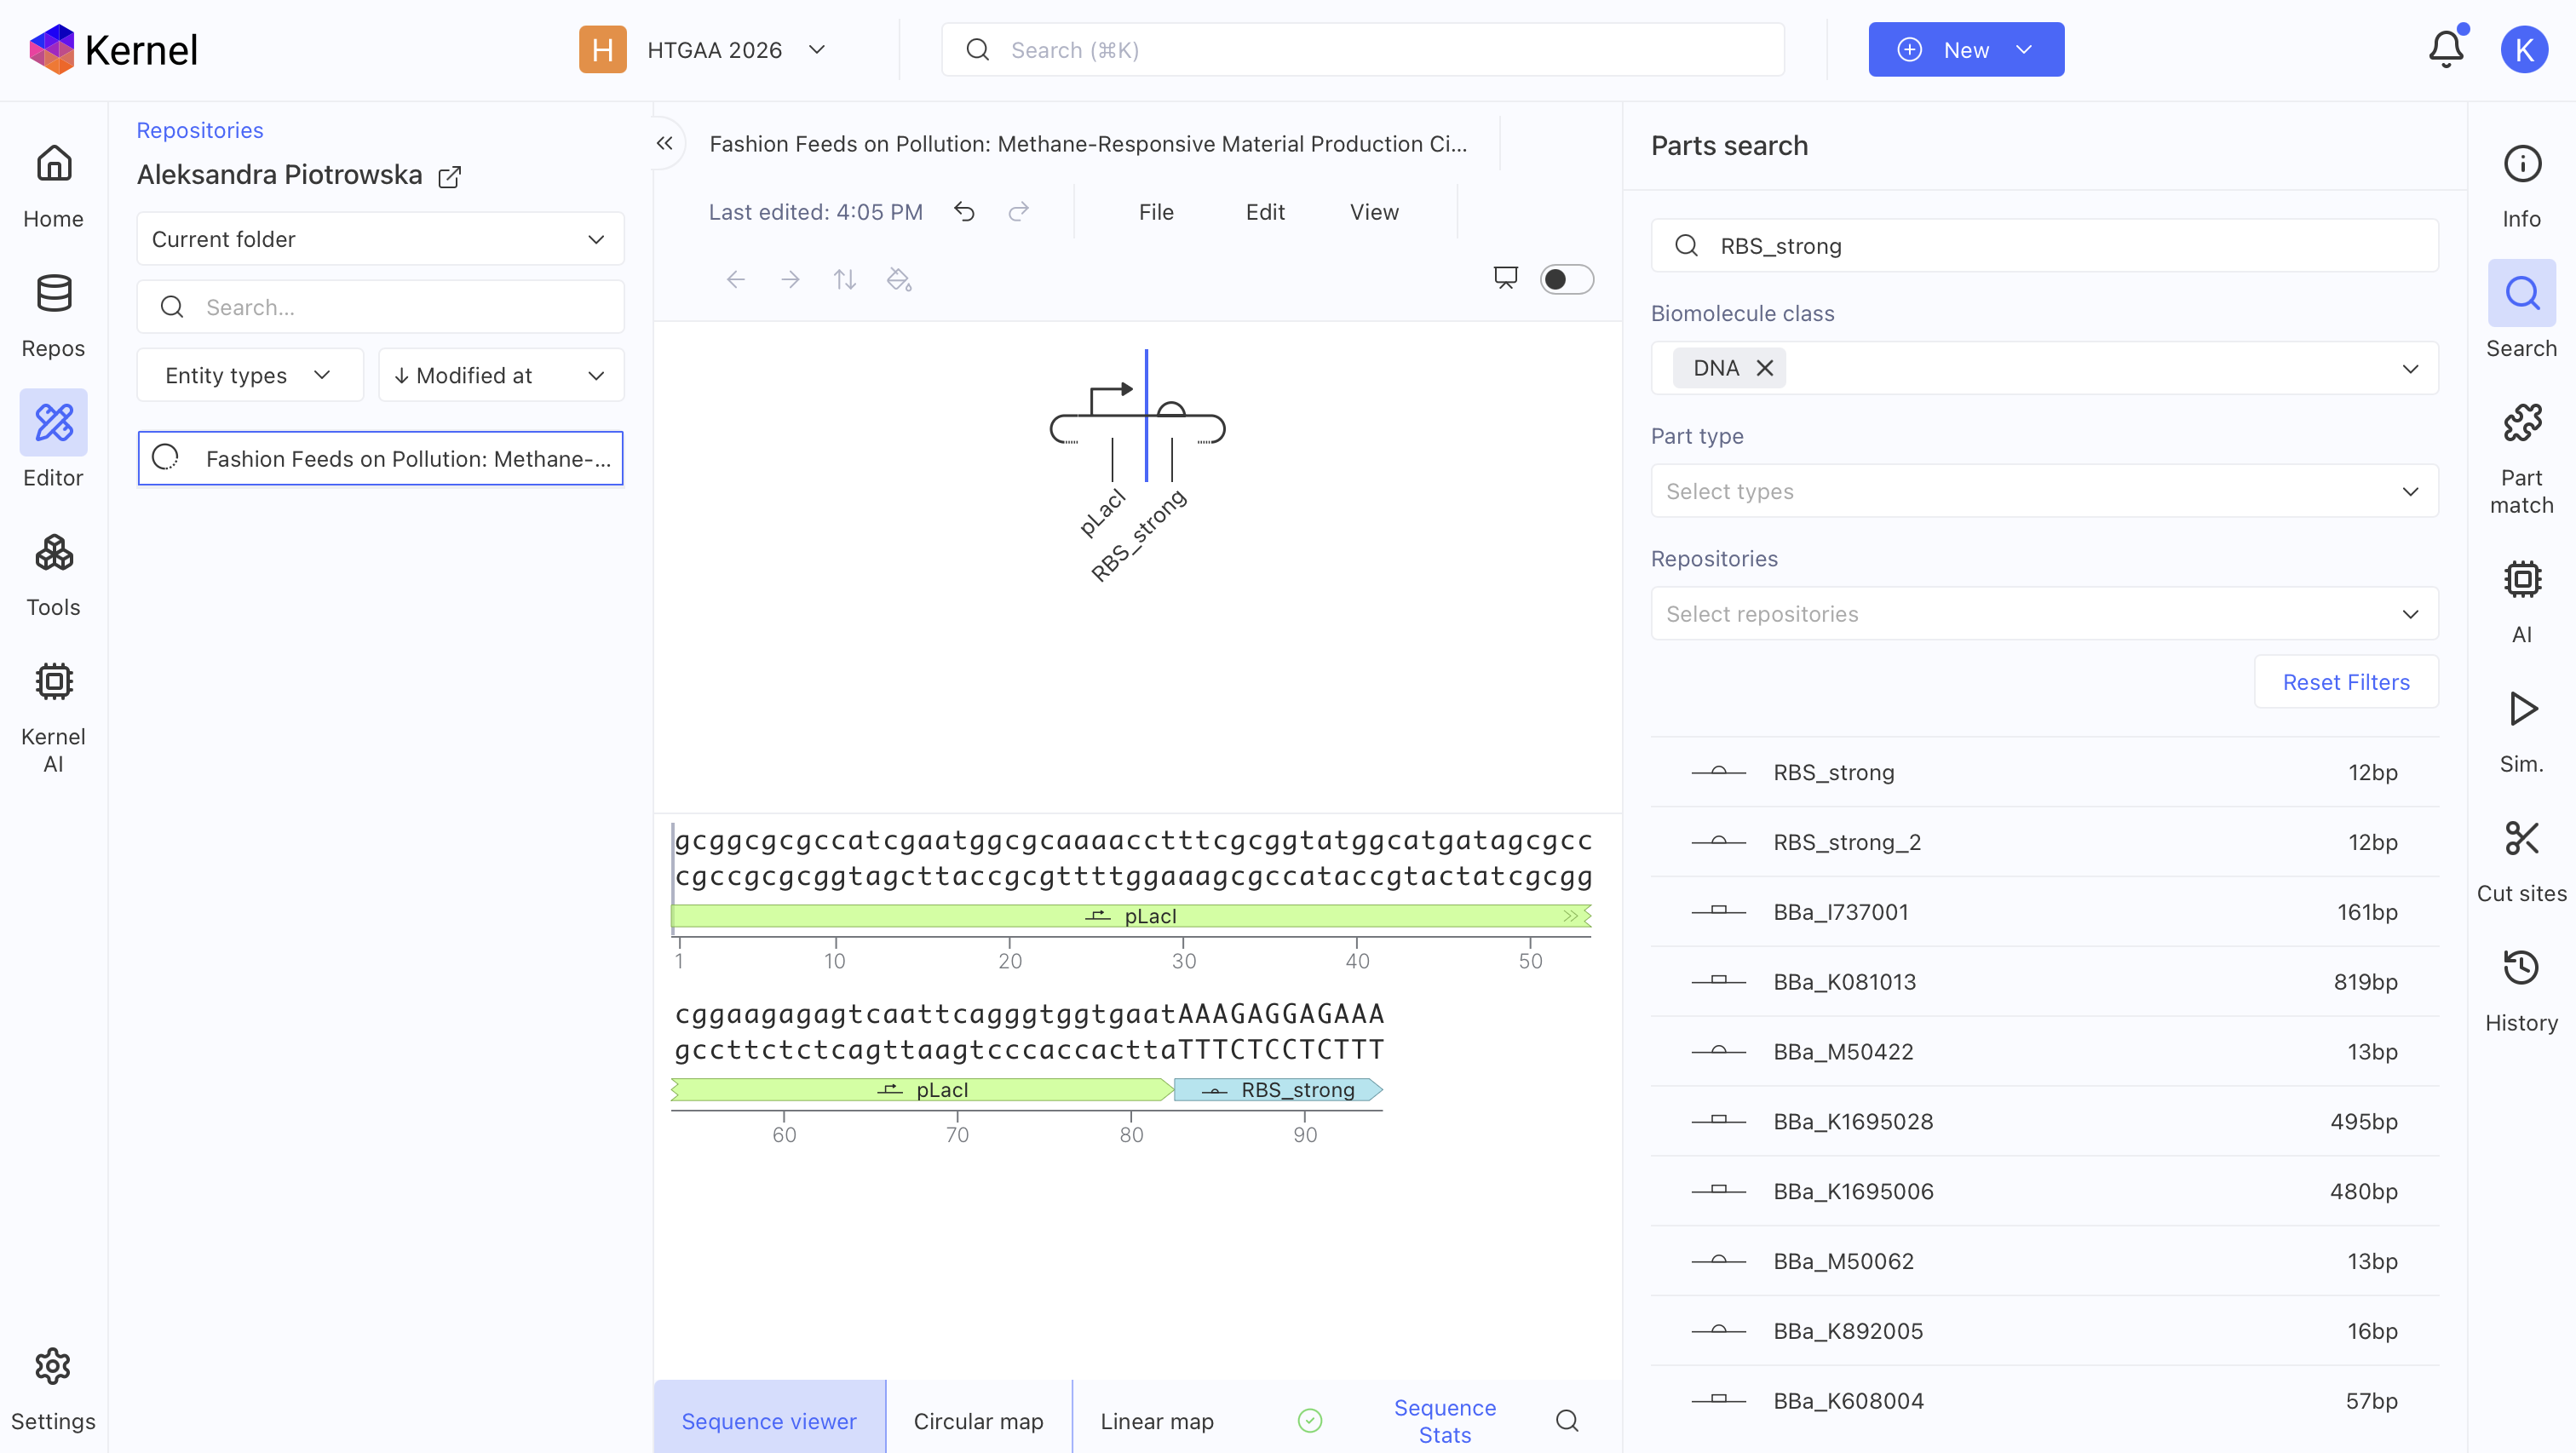
Figure 4. Adding RBS_strong after the promoter.
Selected RBS
RBS_strong
For this first exercise, a strong RBS gave me a simple translation signal with which to observe gene expression.
3. Adding the Reporter
The coding sequence contains the DNA instructions for the protein produced by the circuit.
For this first experiment I used a reporter protein rather than attempting to model material production.
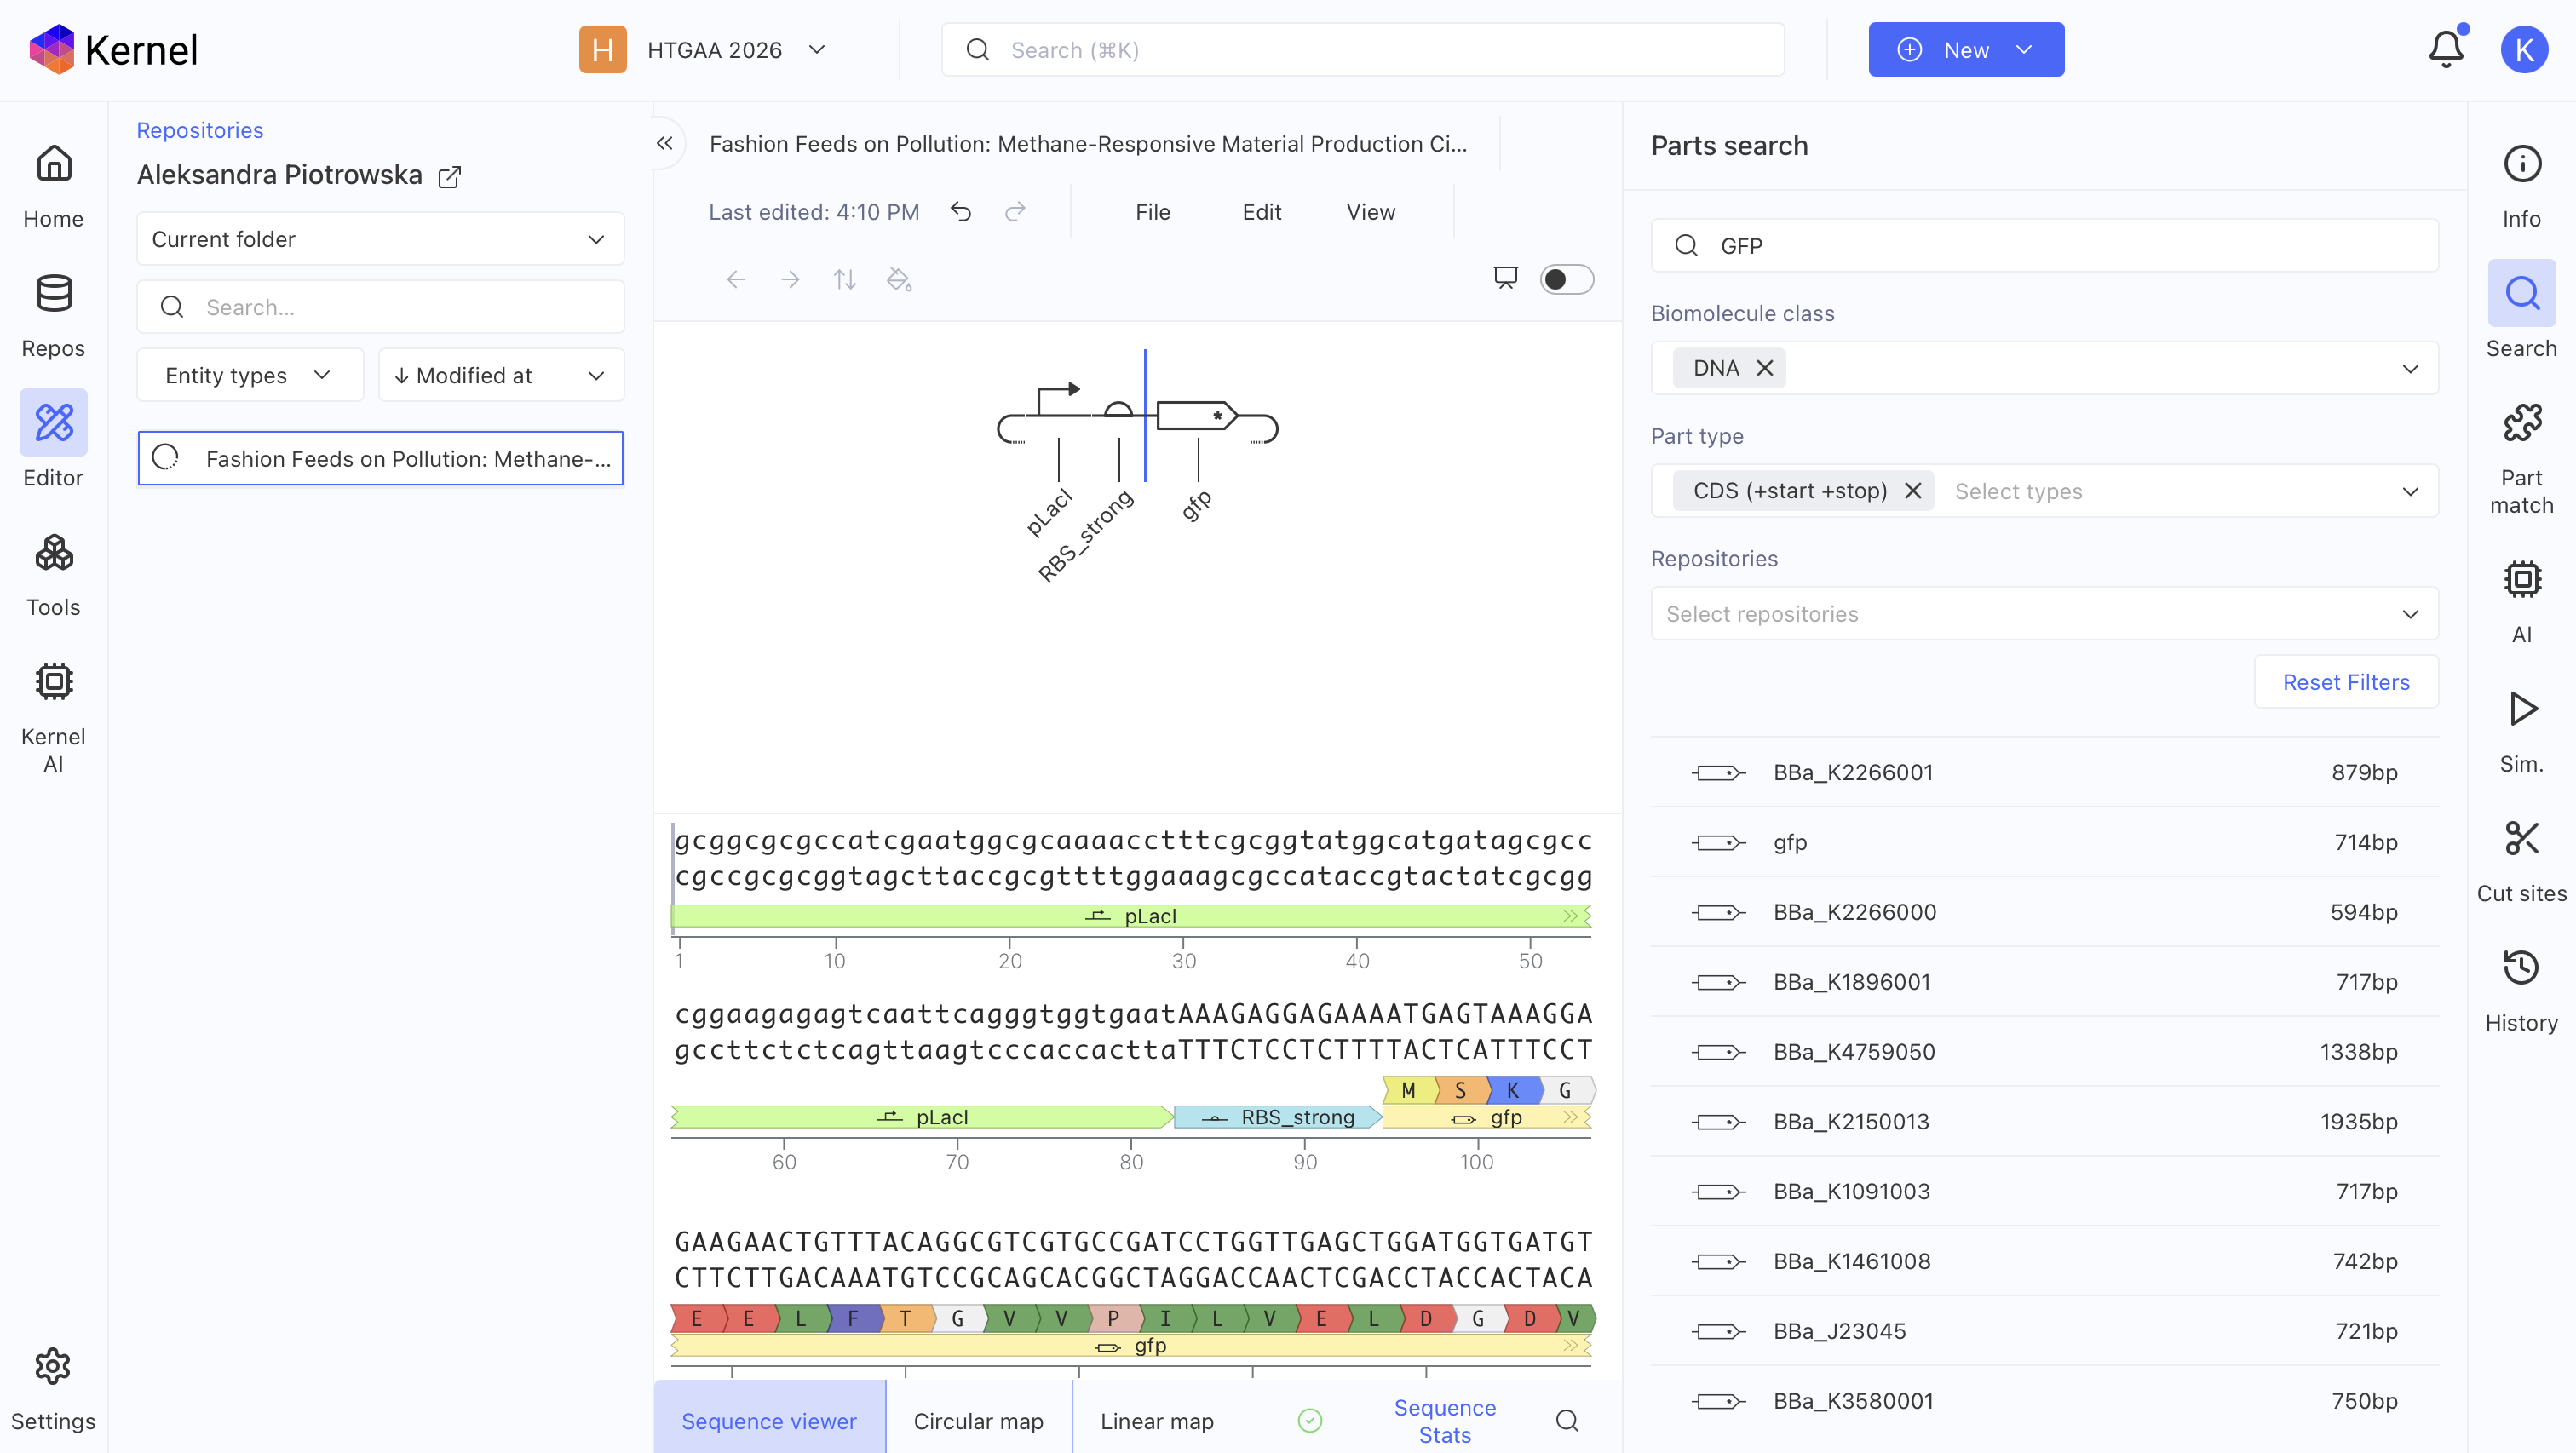
Figure 5. Adding GFP after the promoter and RBS.
Selected reporter
GFP
GFP gives the circuit a simple observable output and allowed me to understand gene expression without immediately introducing the biological complexity of my final project.
4. Adding the Terminator
Finally, I added a transcriptional terminator.
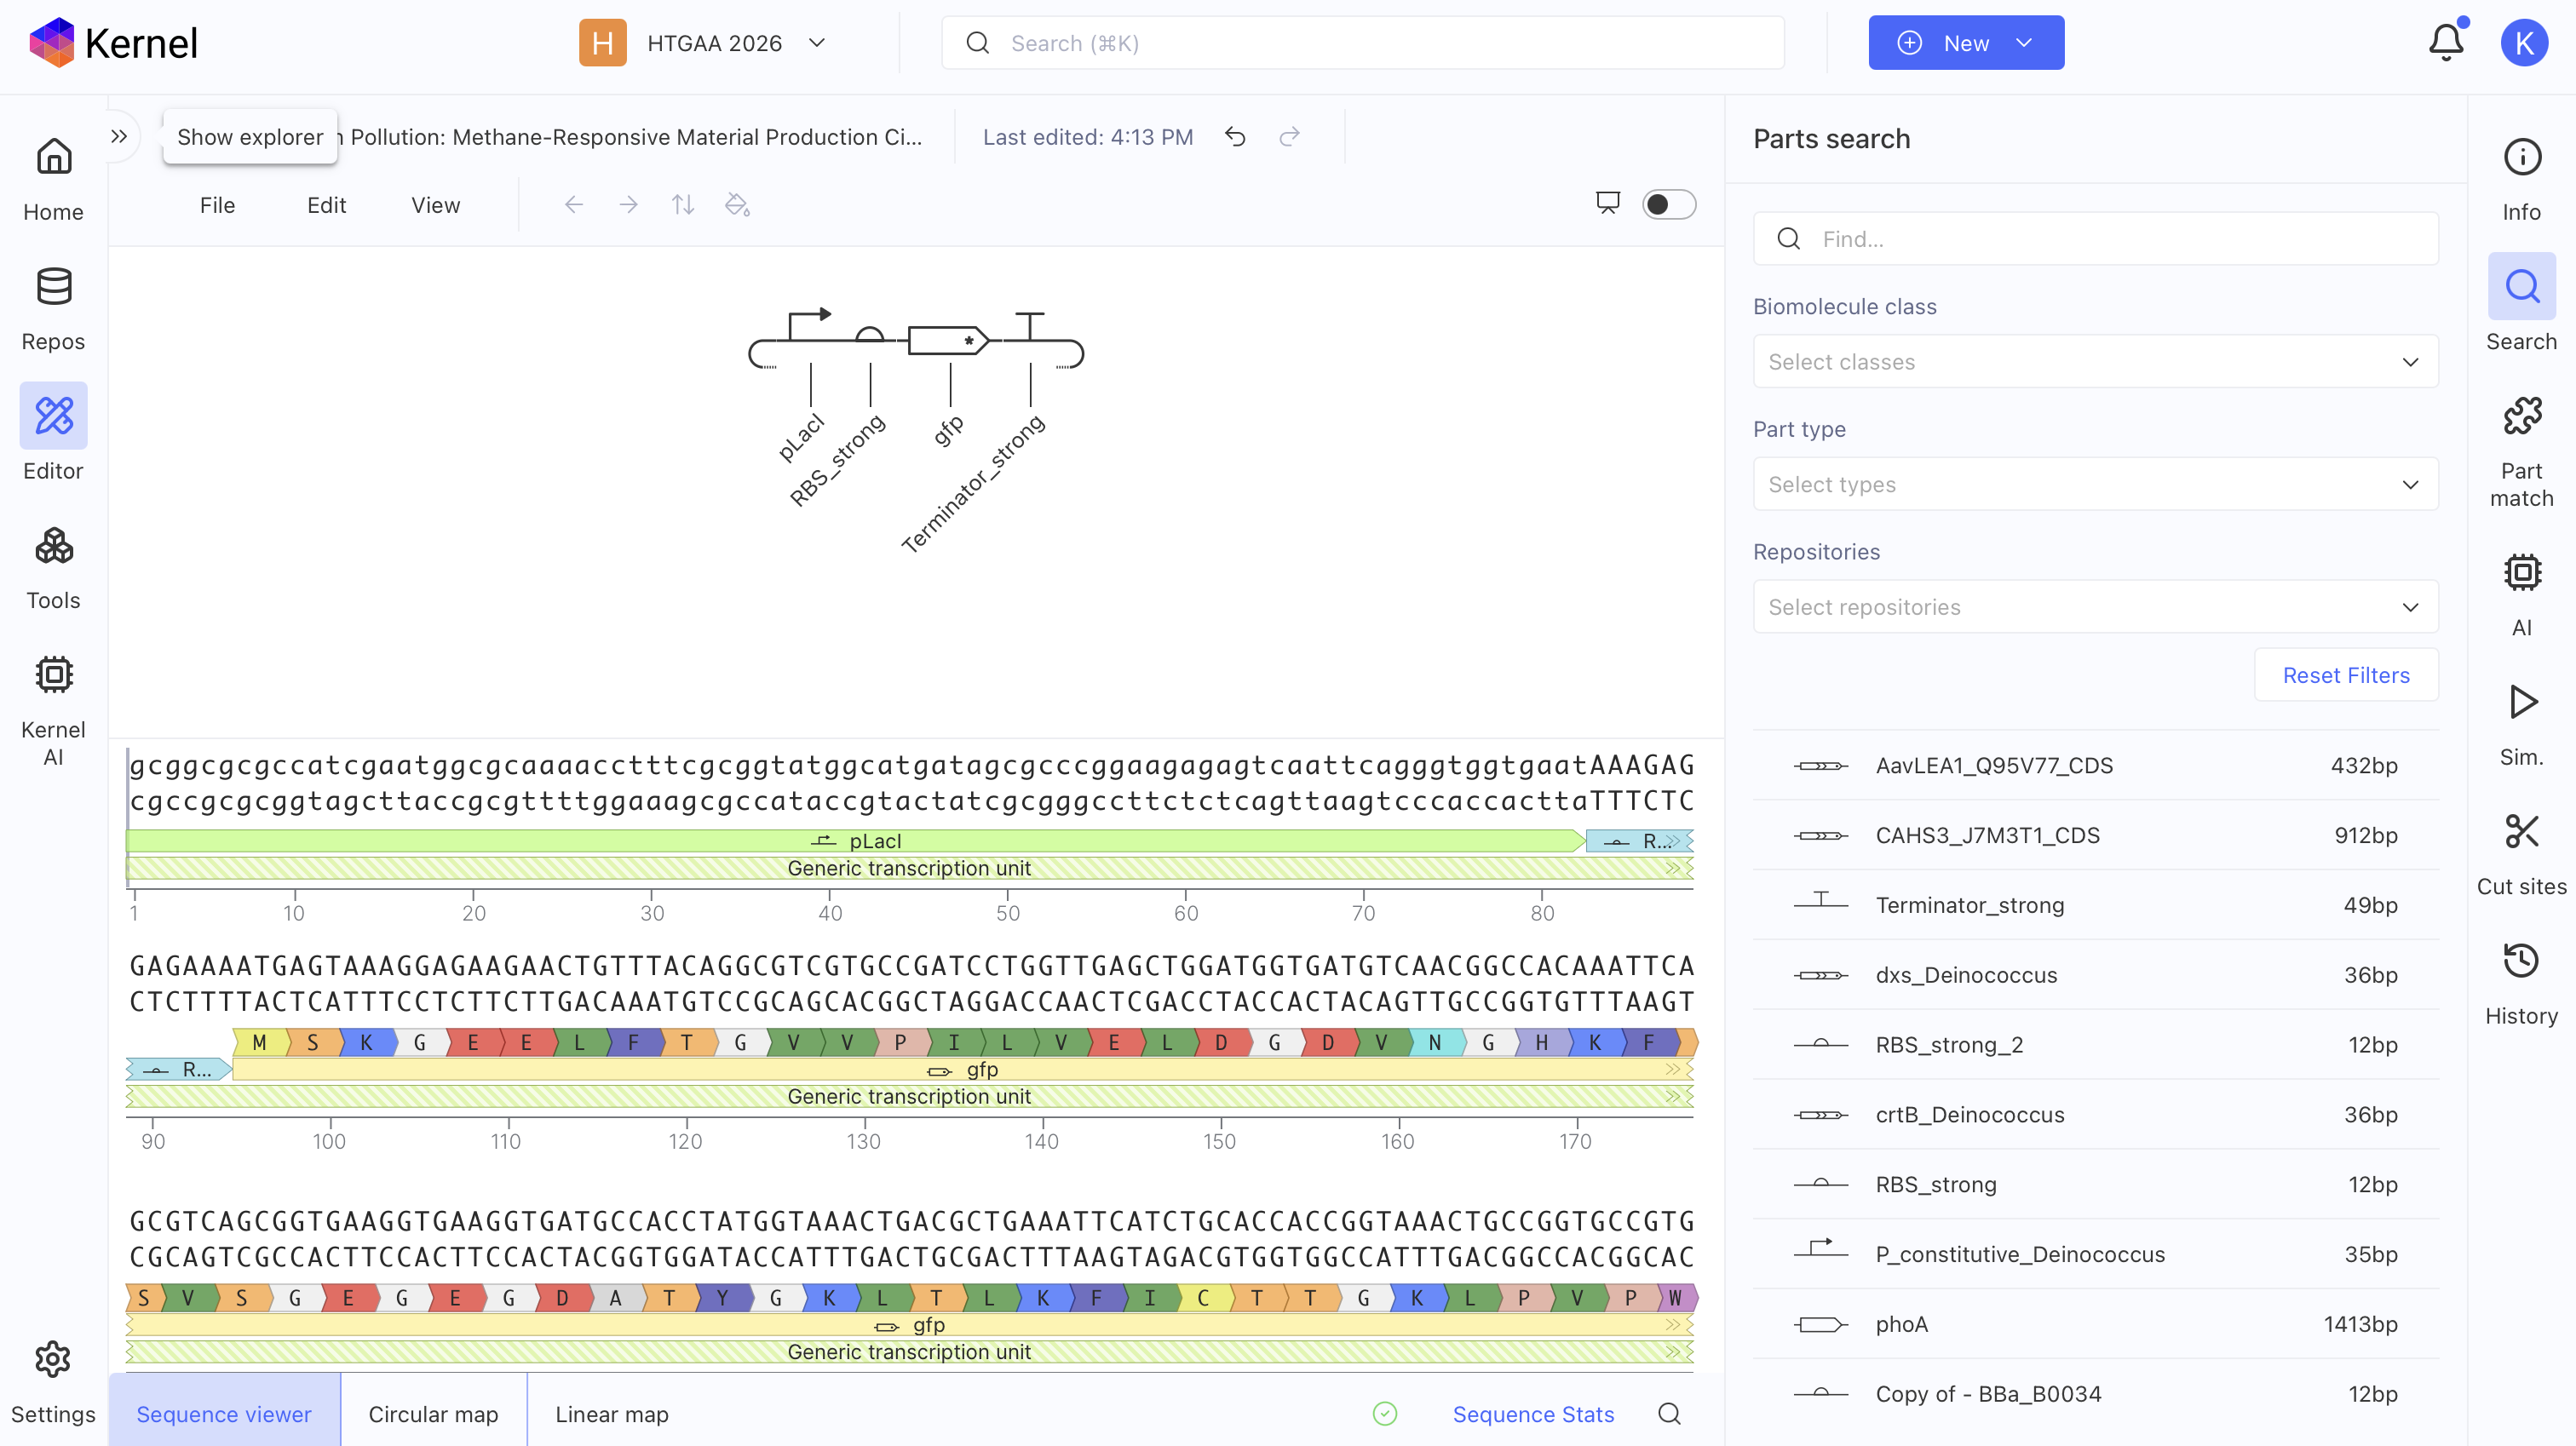
Figure 6. Adding Terminator_strong to complete the transcriptional unit.
Selected terminator
Terminator_strong
The terminator marks where transcription should stop and reduces unwanted transcription beyond the intended unit.
Completed Practice Circuit
The completed practice circuit was:
pLacI → RBS_strong → GFP → Terminator_strong
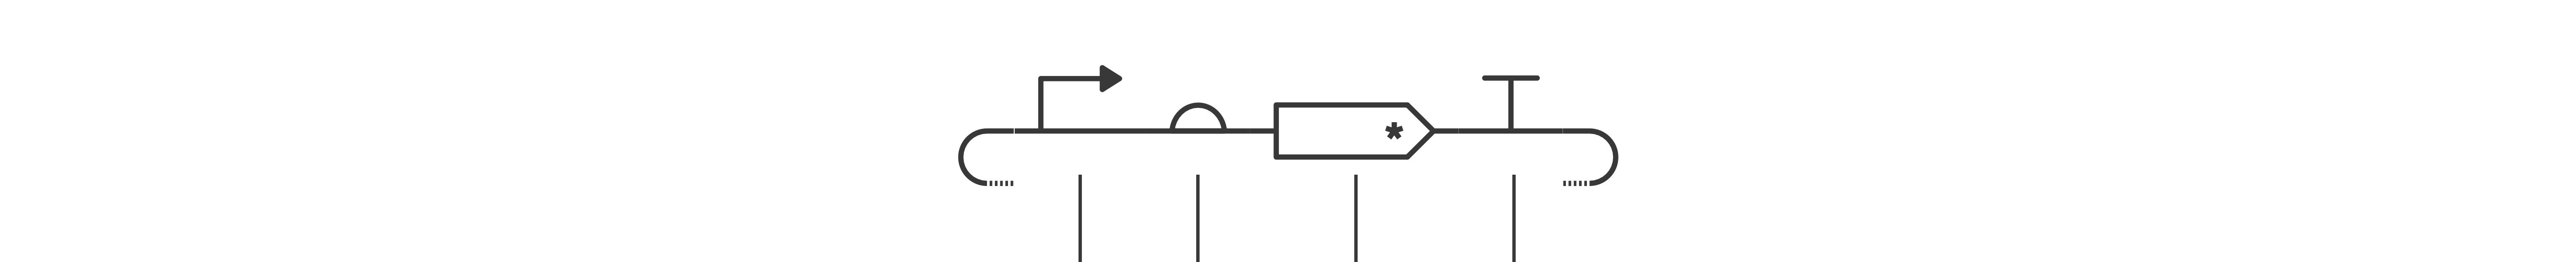
Figure 7. Completed GFP practice circuit in Kernel.
This was my first complete transcriptional unit.
Simulating the Practice Circuit
I then used Kernel’s bacterial simulator to explore the predicted behaviour of the construct.
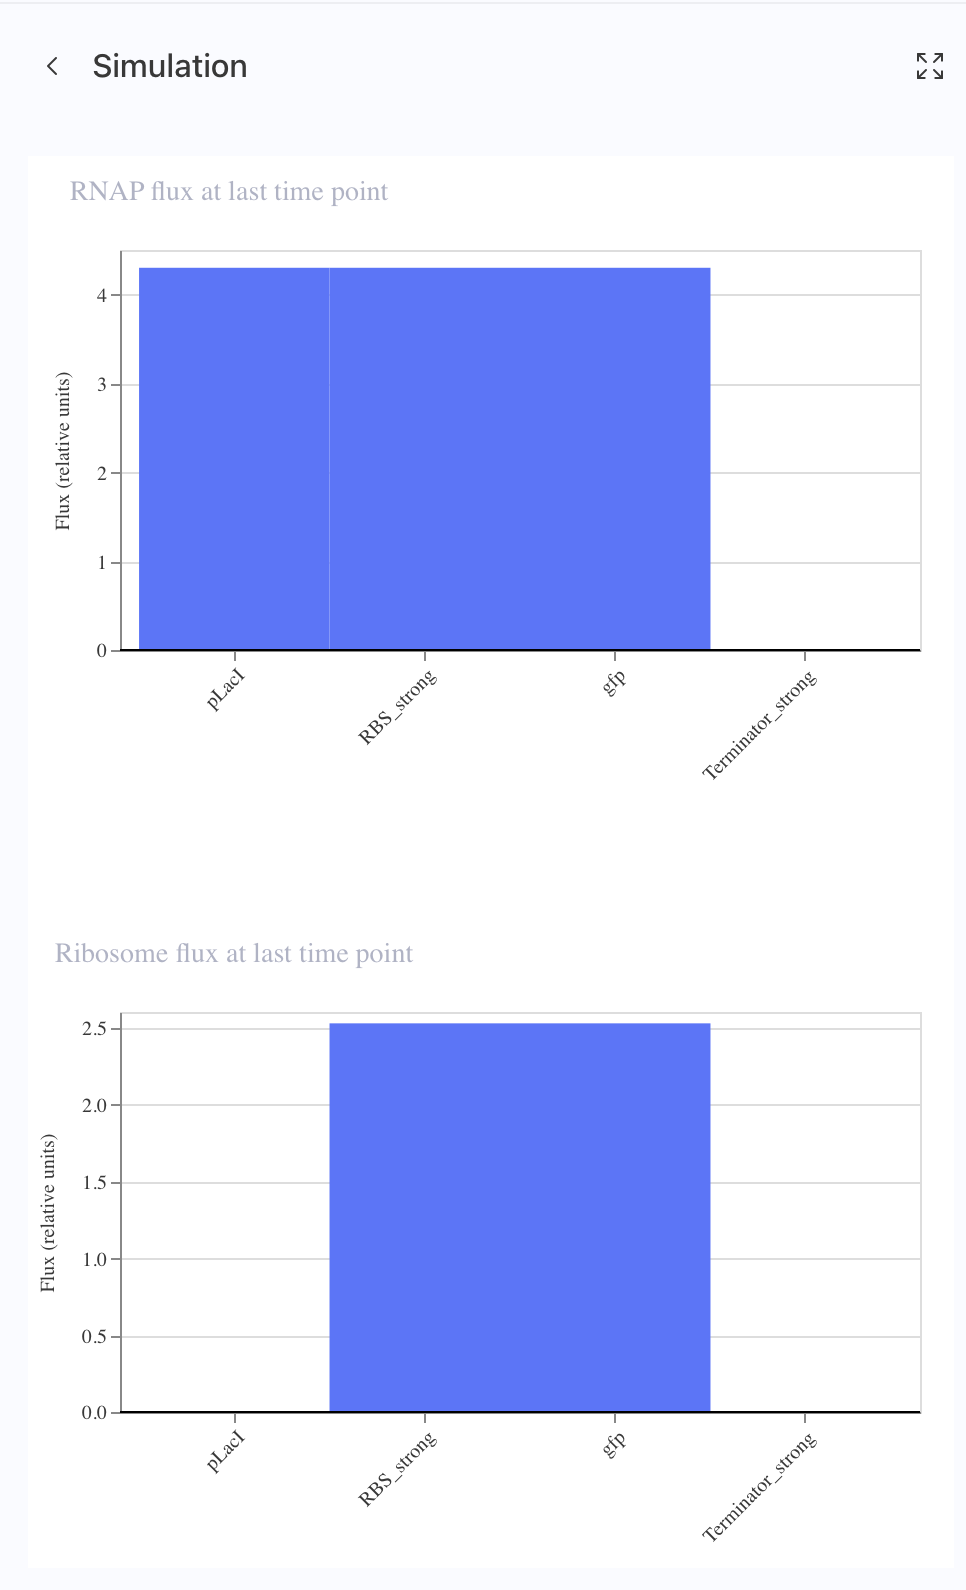
Figure 8. Simulation of the completed practice circuit.
The simulation helped me connect the DNA architecture with different stages of gene expression:
DNA → RNA → PROTEIN
Kernel can predict outputs including RNA polymerase activity, ribosome activity, RNA concentration and protein concentration.
At this point, the simulation was primarily a learning exercise.
I was not yet modelling methane, EPS production or a biomaterial.
Part 2 — From Practice Circuit to Project Circuit
Once I understood the basic structure:
Promoter → RBS → CDS → Terminator
I wanted to move closer to the biological question behind Fashion Feeds on Pollution.
My project asks:
What if methane pollution could become the feedstock for a new flexible biological material for fashion?
Two existing research directions became particularly important to this question.
AirCarbon — Methane Can Become Material
Newlight Technologies’ AirCarbon demonstrates that microorganisms can transform greenhouse-gas carbon into PHB, a biologically produced polymer.
AirCarbon can subsequently be melted and processed into forms including fibre, sheet and solid parts (Newlight Technologies, n.d.).
For me, AirCarbon establishes an important manufacturing precedent:
GREENHOUSE GAS → MICROORGANISM → POLYMER → MATERIAL
However, I do not want simply to reproduce AirCarbon.
Instead, I began asking:
What if the methane-to-material logic demonstrated by AirCarbon could be combined with a different biological production pathway and designed specifically towards a softer, more flexible fashion material?
Girona — A Different Biological Pathway
Recent research from the Catalan Institute for Water Research (ICRA) in Girona investigated the methane-consuming microorganism:
Methylotuvimicrobium alcaliphilum 20Z
Aranda et al. (2026) showed that this methanotroph can produce protein-rich extracellular polymeric substances (EPS) directly from methane.
This is interesting to me because the material is secreted extracellularly rather than following the same intracellular PHB route used by AirCarbon.
The Girona research does not demonstrate a flexible fashion material.
Instead, it creates another biological starting point.
AIRCARBON
greenhouse gas → intracellular PHB → processing → material
ICRA / GIRONA
methane → methanotroph → extracellular polymer
MY QUESTION
methane → controlled extracellular polymer production → material development → flexible fashion application
AirCarbon therefore acts as a precedent for methane / greenhouse-gas-to-material manufacturing, while the Girona research suggests another biological route based on secreted extracellular material.
My project asks what happens when those two lines of thinking are brought together for fashion.
A Geographical Research System
The project is also beginning to connect three places that are relevant to my own trajectory:
SILESIA
the future feedstock ambition — methane associated with the post-coal landscape I come from
↓
CATALONIA
where I am currently based and where emerging methane-to-EPS research is being produced
↓
LONDON
where a future material-development phase could connect the biology with fashion, fabrication and material research
This makes the project not only a biological question, but also a question of how different research and industrial ecosystems might connect.
What Should the Genetic Circuit Do?
I am not trying to design a gene that literally means:
“make a flexible material.”
Flexibility would eventually depend on the composition of the biological material and what happens during recovery, formulation and processing.
The genetic circuit sits earlier in the system.
The question becomes:
What if the microorganism could first grow using methane and then be switched into a material-production state?
Conceptually:
GROWTH
Methane → microbial growth
and later:
PRODUCTION
Control signal → genetic regulation → material-production pathway
This gave me the starting architecture:
Controllable promoter → RBS → candidate production regulator → terminator
The exact genetic control of the methane-derived EPS reported by Aranda et al. (2026) remains poorly characterised.
I therefore treat the circuit as a research hypothesis, rather than pretending that the final biological pathway is already known.
Creating the Project Circuit in Kernel
I created a second construct:
Fashion Feeds on Pollution: Project Circuit
Step 1 — Choosing a Controllable Promoter
For the intended biological system, I am interested in an inducible promoter because the long-term ambition is to explore switching between growth and production states.
Goswami et al. (2024) demonstrated both inducible and constitutive gene-expression tools in Methylotuvimicrobium alcaliphilum, showing that controllable genetic expression in this methanotroph is experimentally possible.
The methanotroph-specific inducible promoter I was interested in was not available as a ready-made part in Kernel.
I therefore used a characterised bacterial promoter as a proxy for the regulatory logic.
I selected:
pTetR
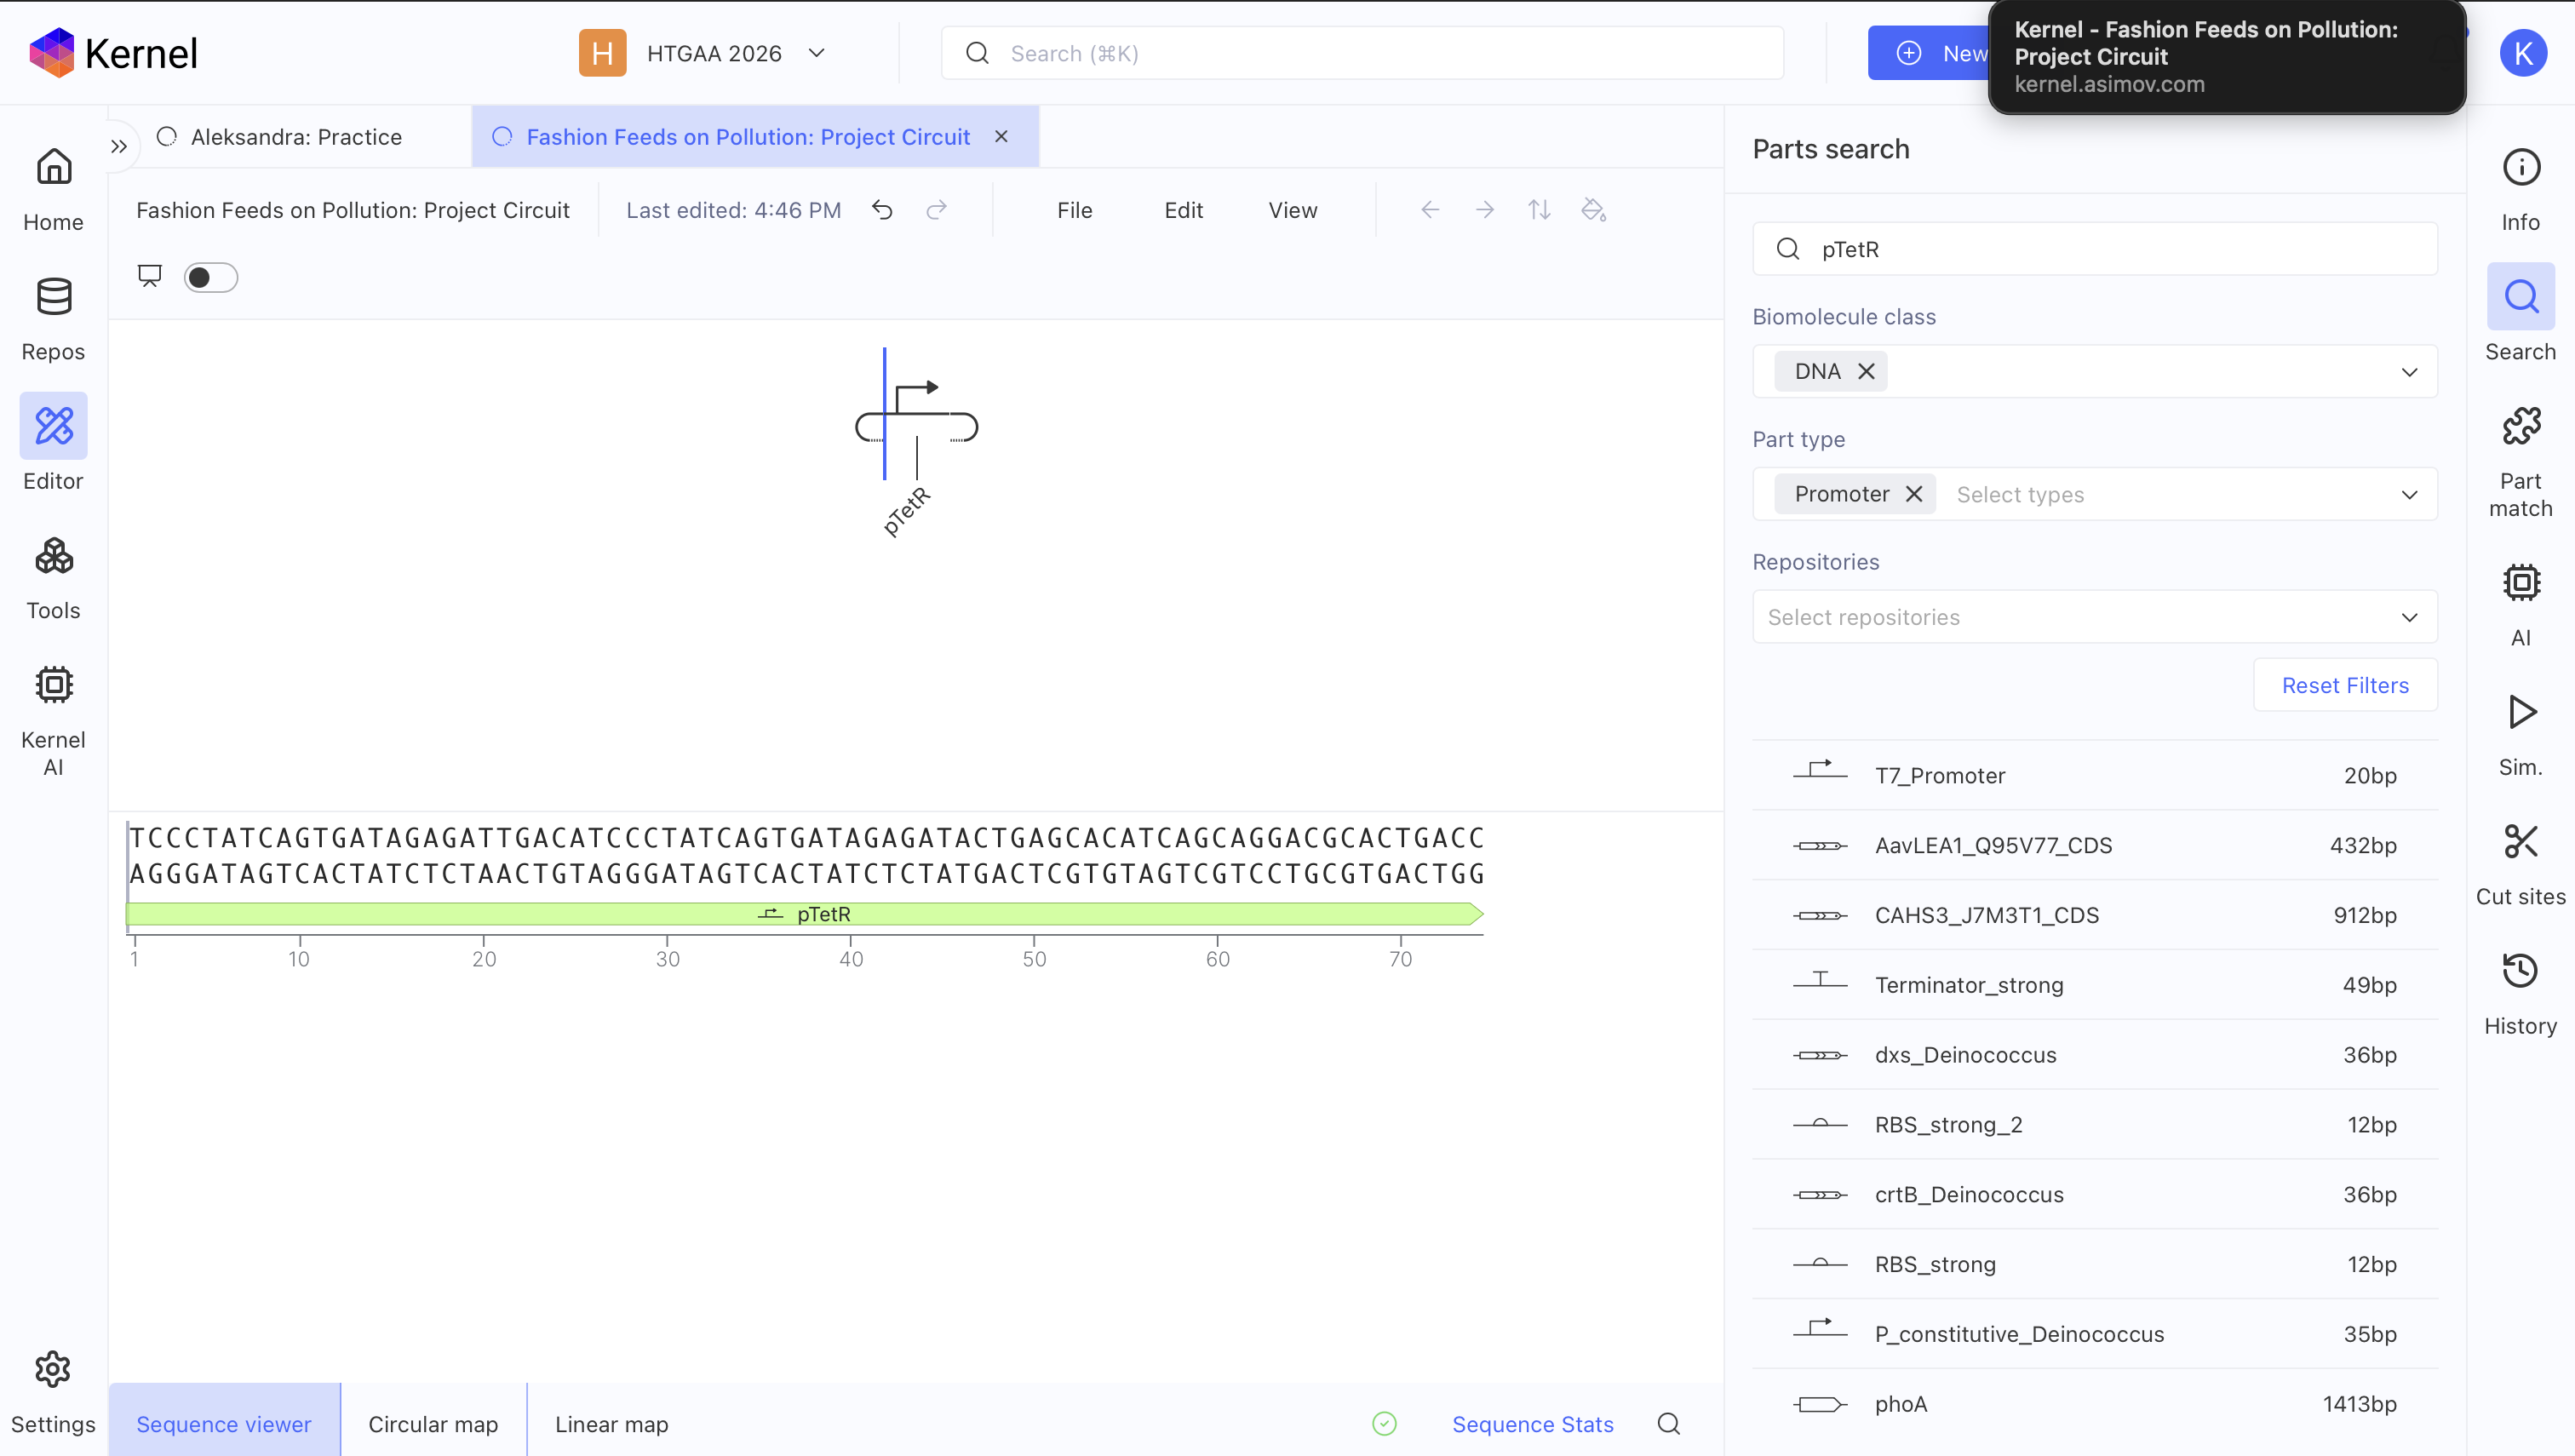
Figure 9. Searching for pTetR in Kernel.
Kernel identifies pTetR as a promoter containing TetO operator sequences and regulated by the TetR repressor.
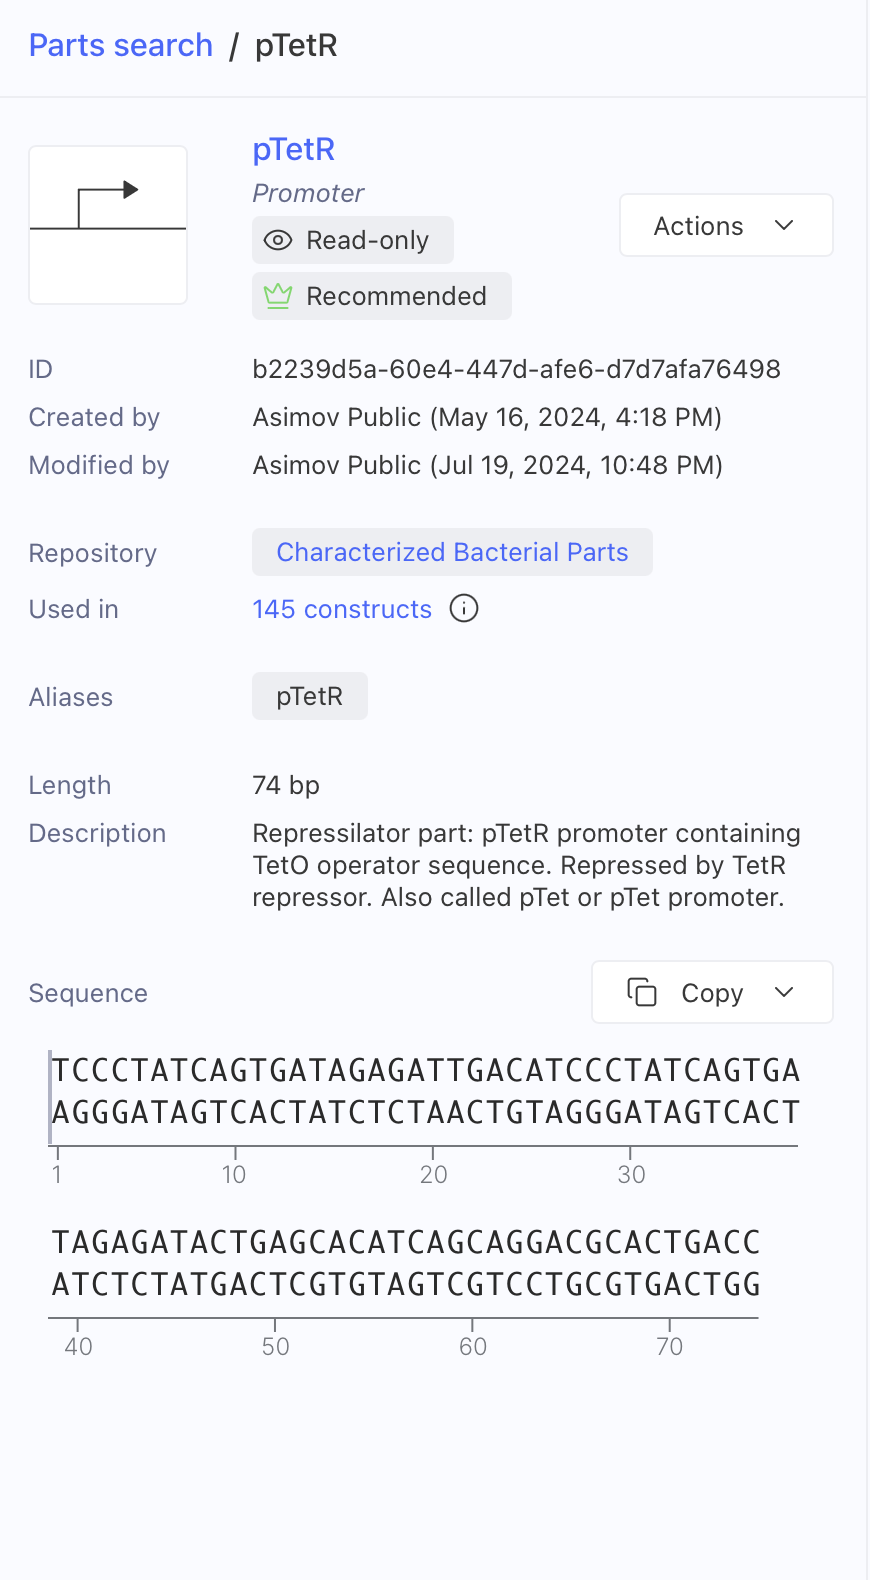
Figure 10. Information panel for the characterised pTetR promoter.
This does not mean pTetR would necessarily be the final promoter used in M. alcaliphilum.
Its purpose here is to let me explore controllable expression architecture.
Step 2 — Adding the RBS
I added:
RBS_strong
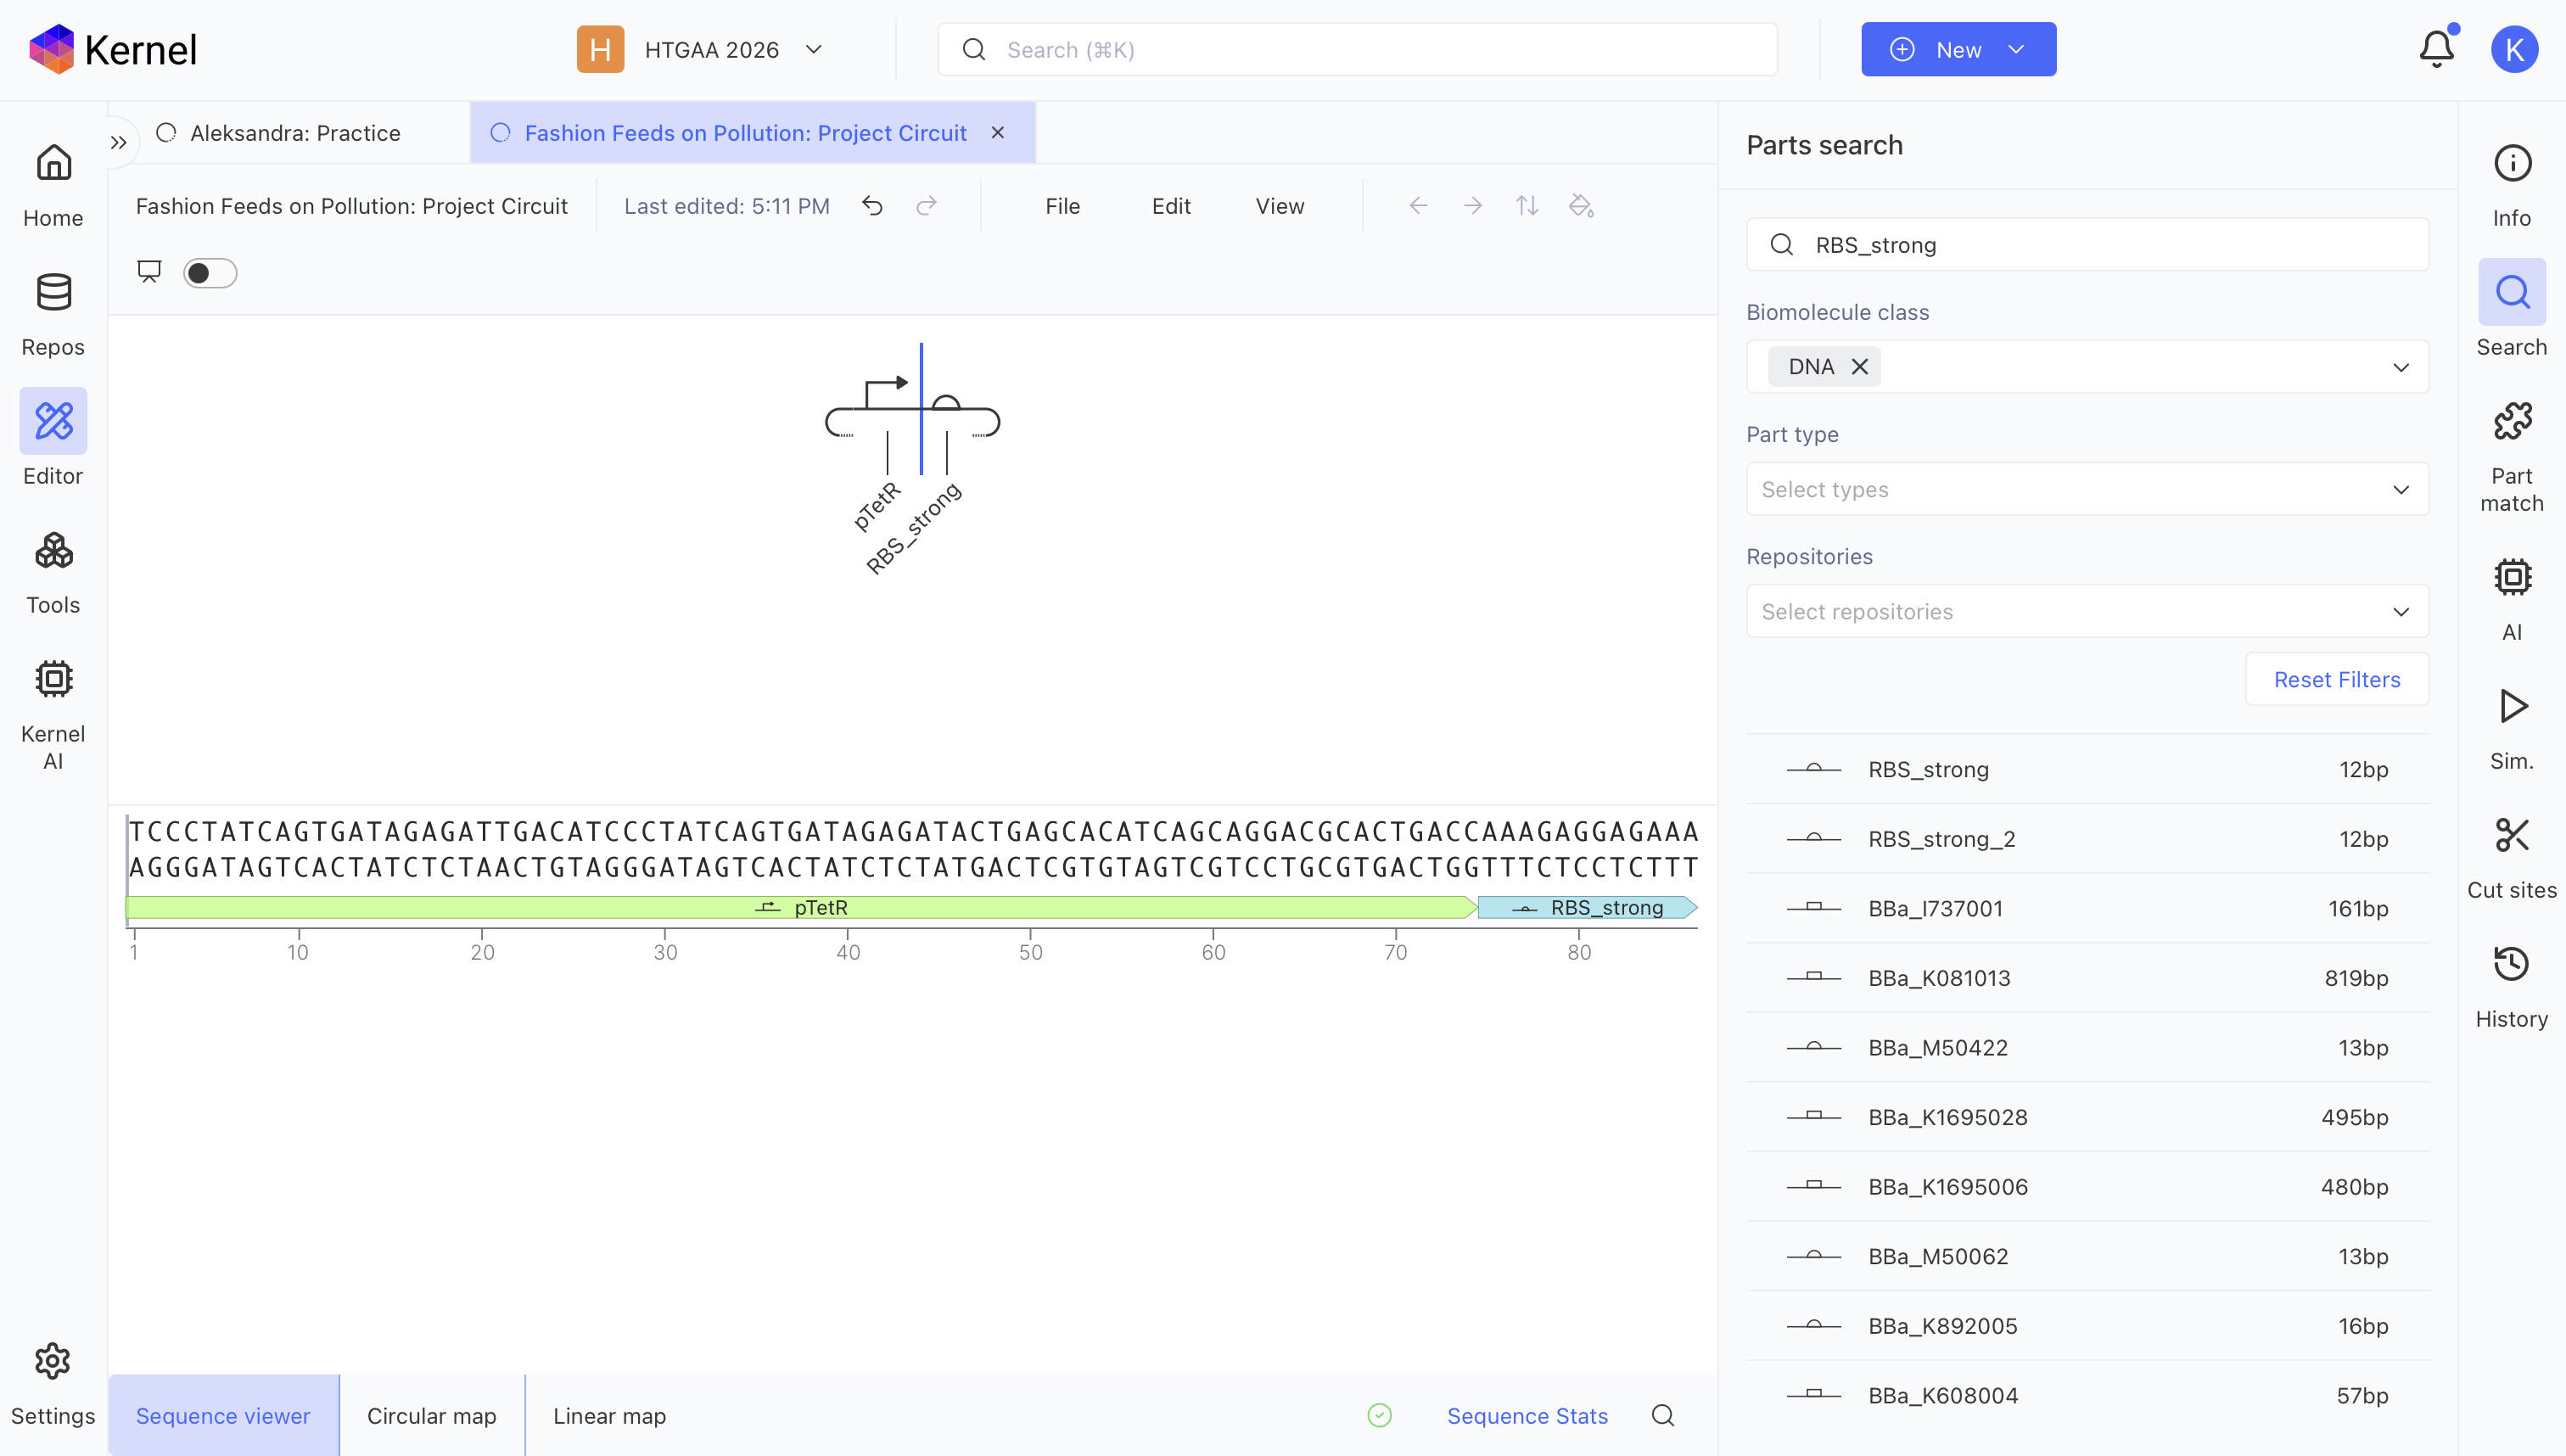
Figure 11. Adding RBS_strong after pTetR.
The circuit now began:
pTetR → RBS_strong → …
Step 3 — Choosing a Candidate Material-Production Regulator
This was the point where the circuit became more project-specific.
Rather than adding another generic reporter, I wanted to explore a gene connected to regulation of extracellular material production.
I selected:
BBa_K1019004 — YdeH Diguanylate Cyclase
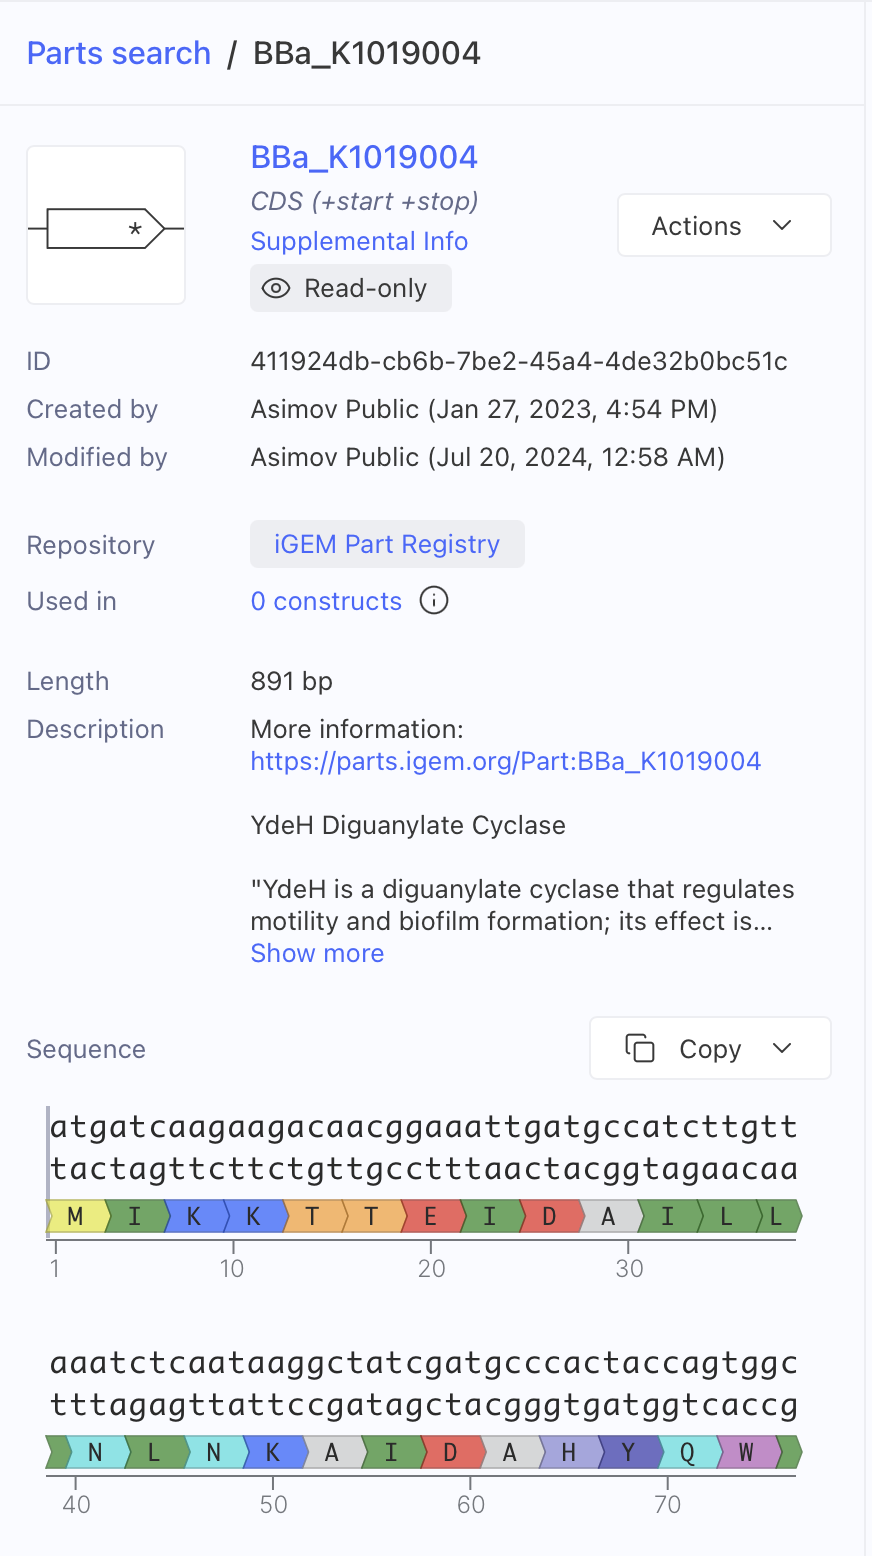
Figure 12. Kernel information panel for the YdeH diguanylate cyclase coding sequence.
YdeH is a diguanylate cyclase from E. coli that produces the bacterial signalling molecule c-di-GMP (Zähringer, Massa & Schirmer, 2011).
c-di-GMP is involved in the regulation of several bacterial extracellular polysaccharide systems, and YdeH has been linked to c-di-GMP-dependent extracellular polysaccharide regulation in E. coli (Poulin & Kuperman, 2021).
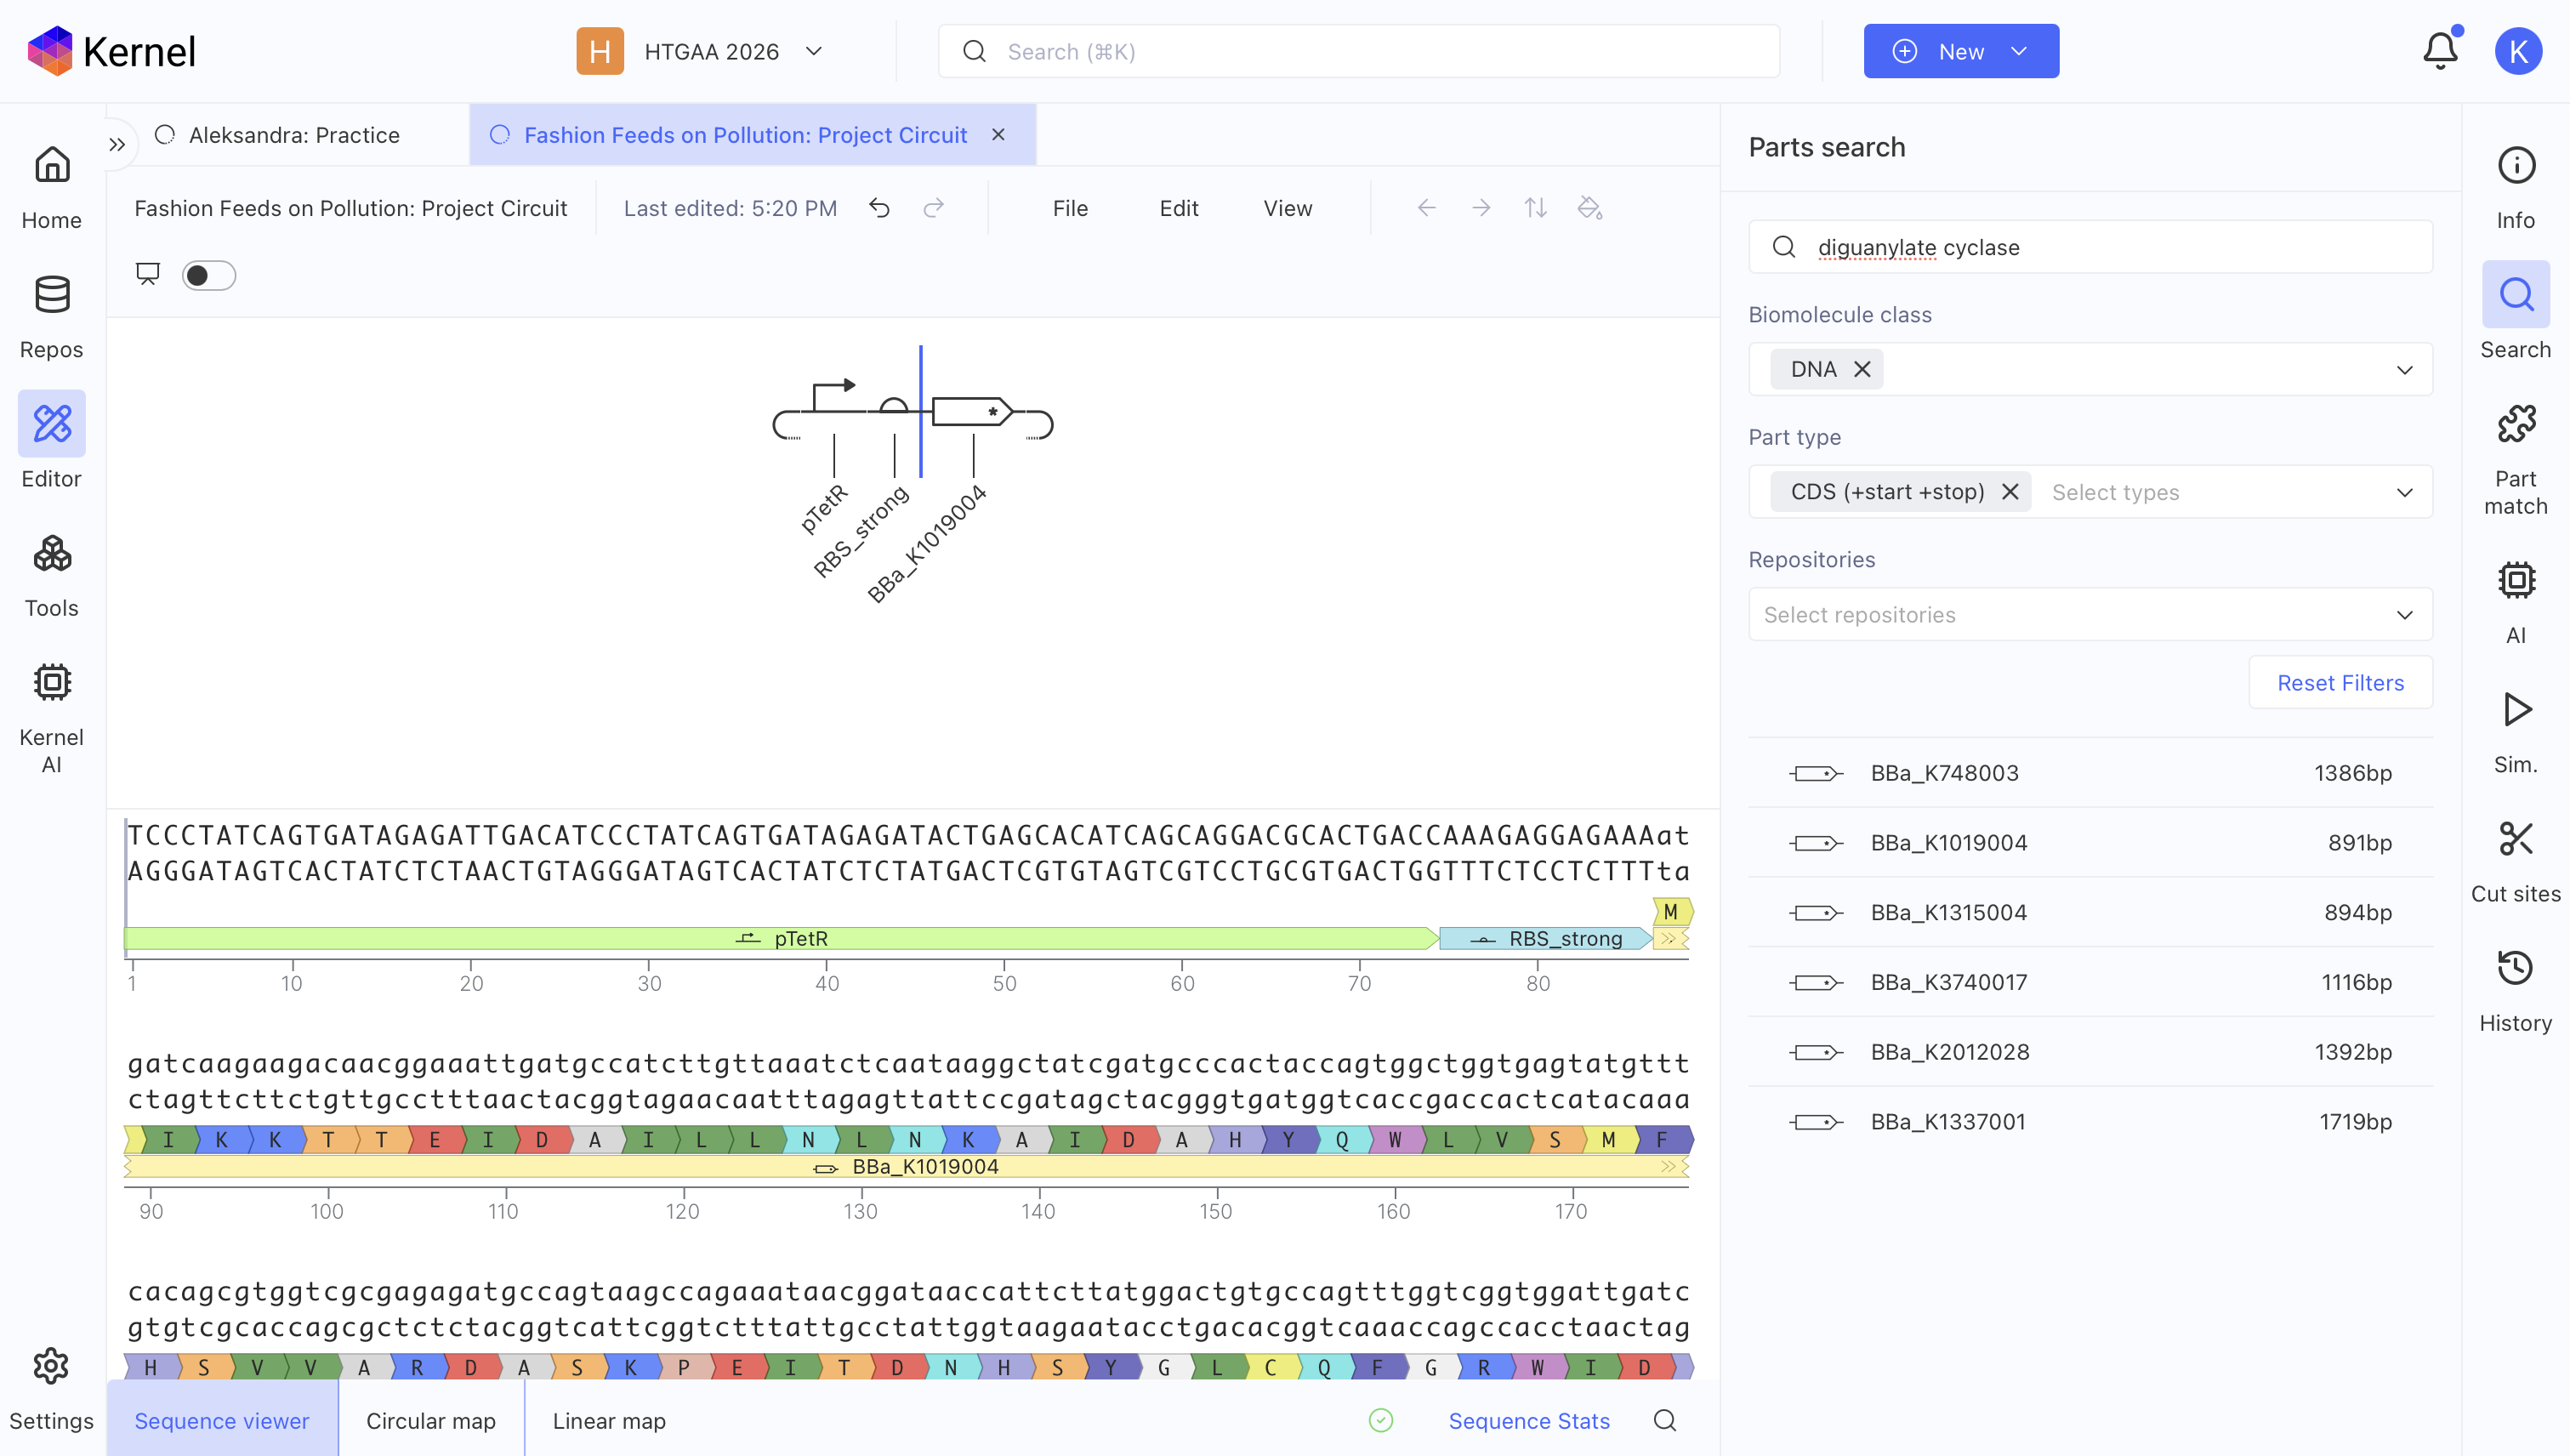
Figure 13. Adding BBa_K1019004 / YdeH to the project circuit.
This distinction is important:
YdeH is not a proven regulator of the protein-rich methane-derived EPS produced by M. alcaliphilum.
I am using it as a proxy for a possible regulatory intervention.
The hypothesis becomes:
What if increasing a biological signal associated with extracellular-matrix production could increase or alter methane-derived EPS production?
Step 4 — Completing the First Production Unit
I added:
Terminator_strong
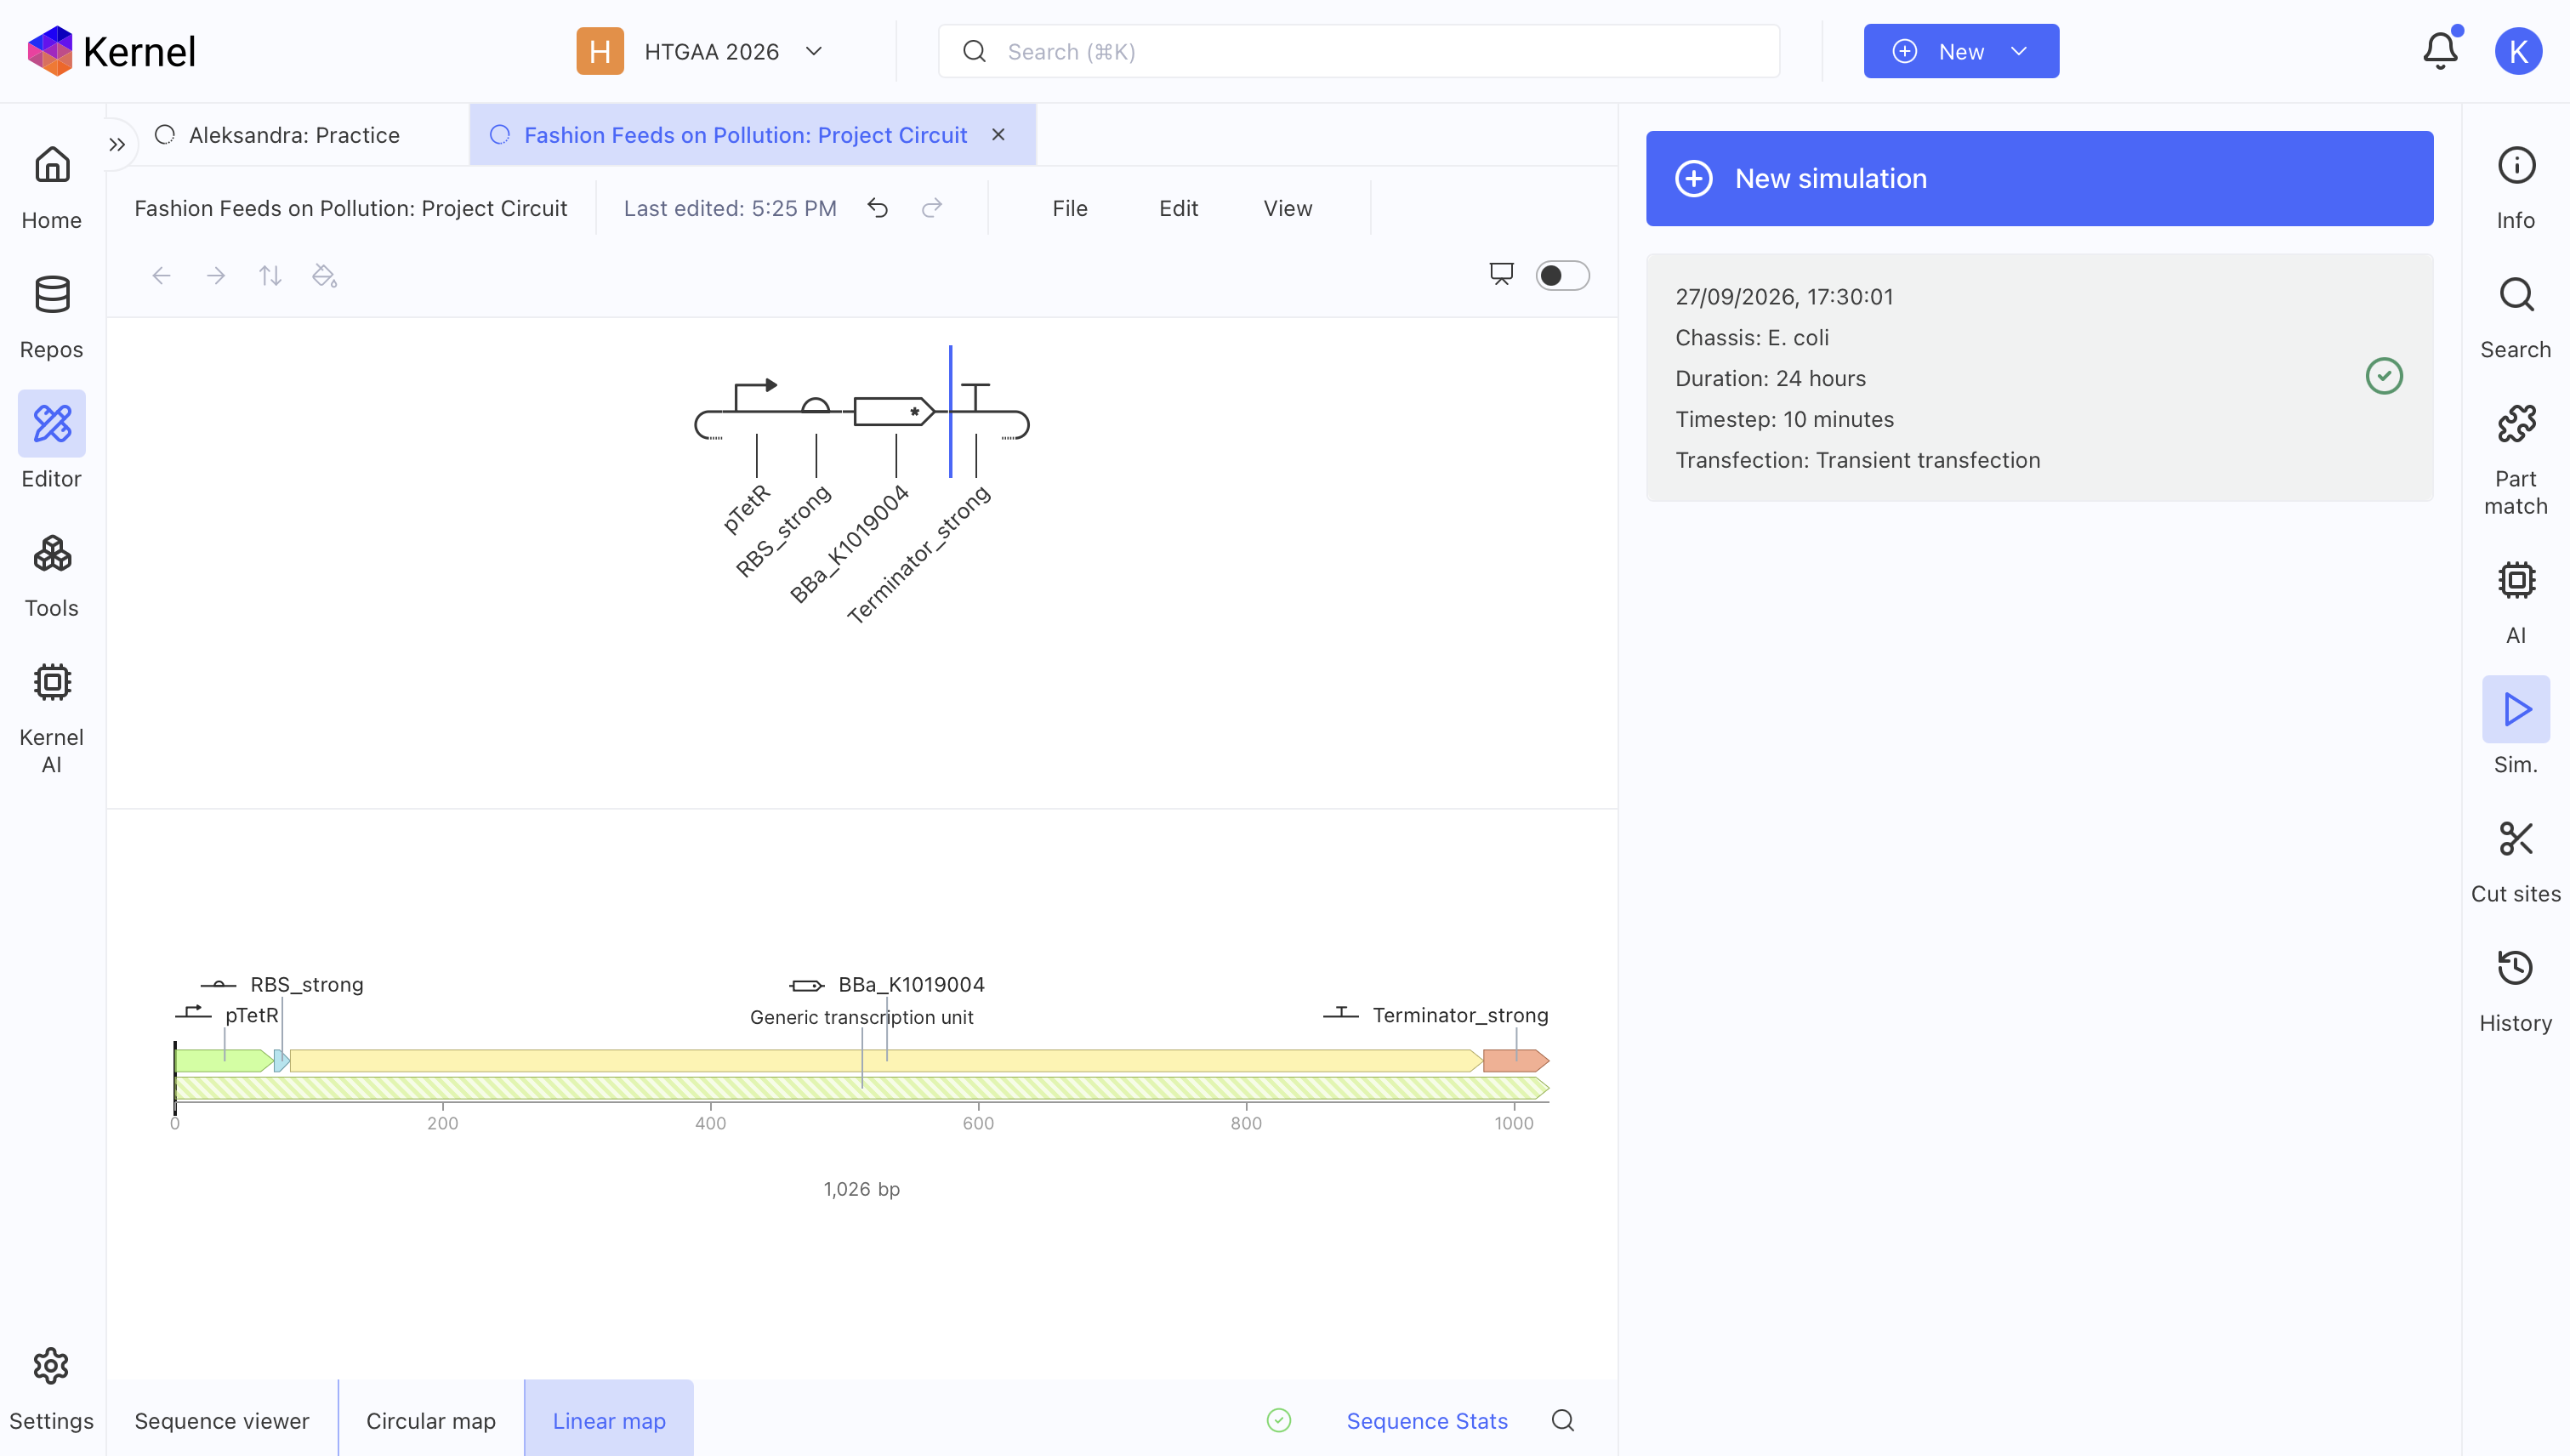
Figure 14. Completed first project-specific production unit.
The first version of the construct was 1,026 bp long:
pTetR → RBS_strong → YdeH → Terminator_strong
The roles of the parts were:
pTetR
↓ controllable transcription
RBS_strong
↓ translation
YdeH
↓ candidate c-di-GMP regulatory intervention
Terminator_strong
↓ stop transcription
This was a testable hypothesis circuit, not a validated methane-to-EPS pathway.
Simulating the First Project Circuit
I simulated the construct using:
- Chassis: E. coli
- Duration: 24 hours
- Time step: 10 minutes
- Transfection type: Transient transfection
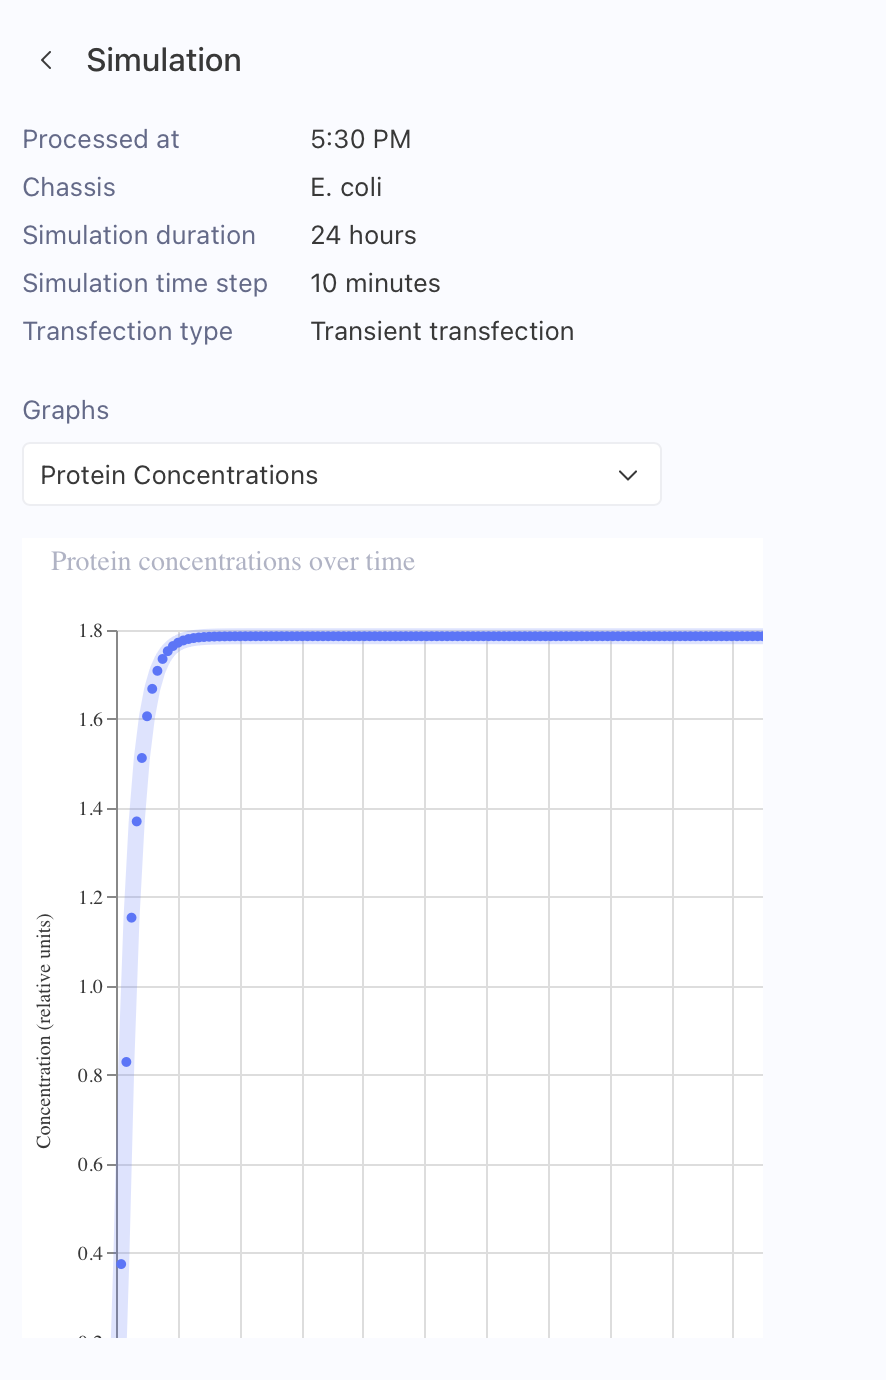
Figure 15. Predicted YdeH protein concentration for the first project circuit.
Kernel predicted that YdeH concentration rapidly increased and then stabilised at approximately:
1.8 relative units
This means Kernel predicted expression of the YdeH protein.
It does not mean that the simulation produced EPS or a biomaterial.
The software was modelling:
GENE EXPRESSION
not:
METHANE → EPS → MATERIAL
There was also an important problem with this first design:
pTetR was present, but TetR was not.
The circuit therefore did not yet contain the repressor needed to turn pTetR into a complete regulatory system.
That created the next design question:
How can I turn the production unit into a controllable genetic switch?
Step 5 — Building the Control Unit
To regulate pTetR, I needed a second transcriptional unit capable of producing the TetR repressor.
I selected the constitutive promoter:
BBa_J23101
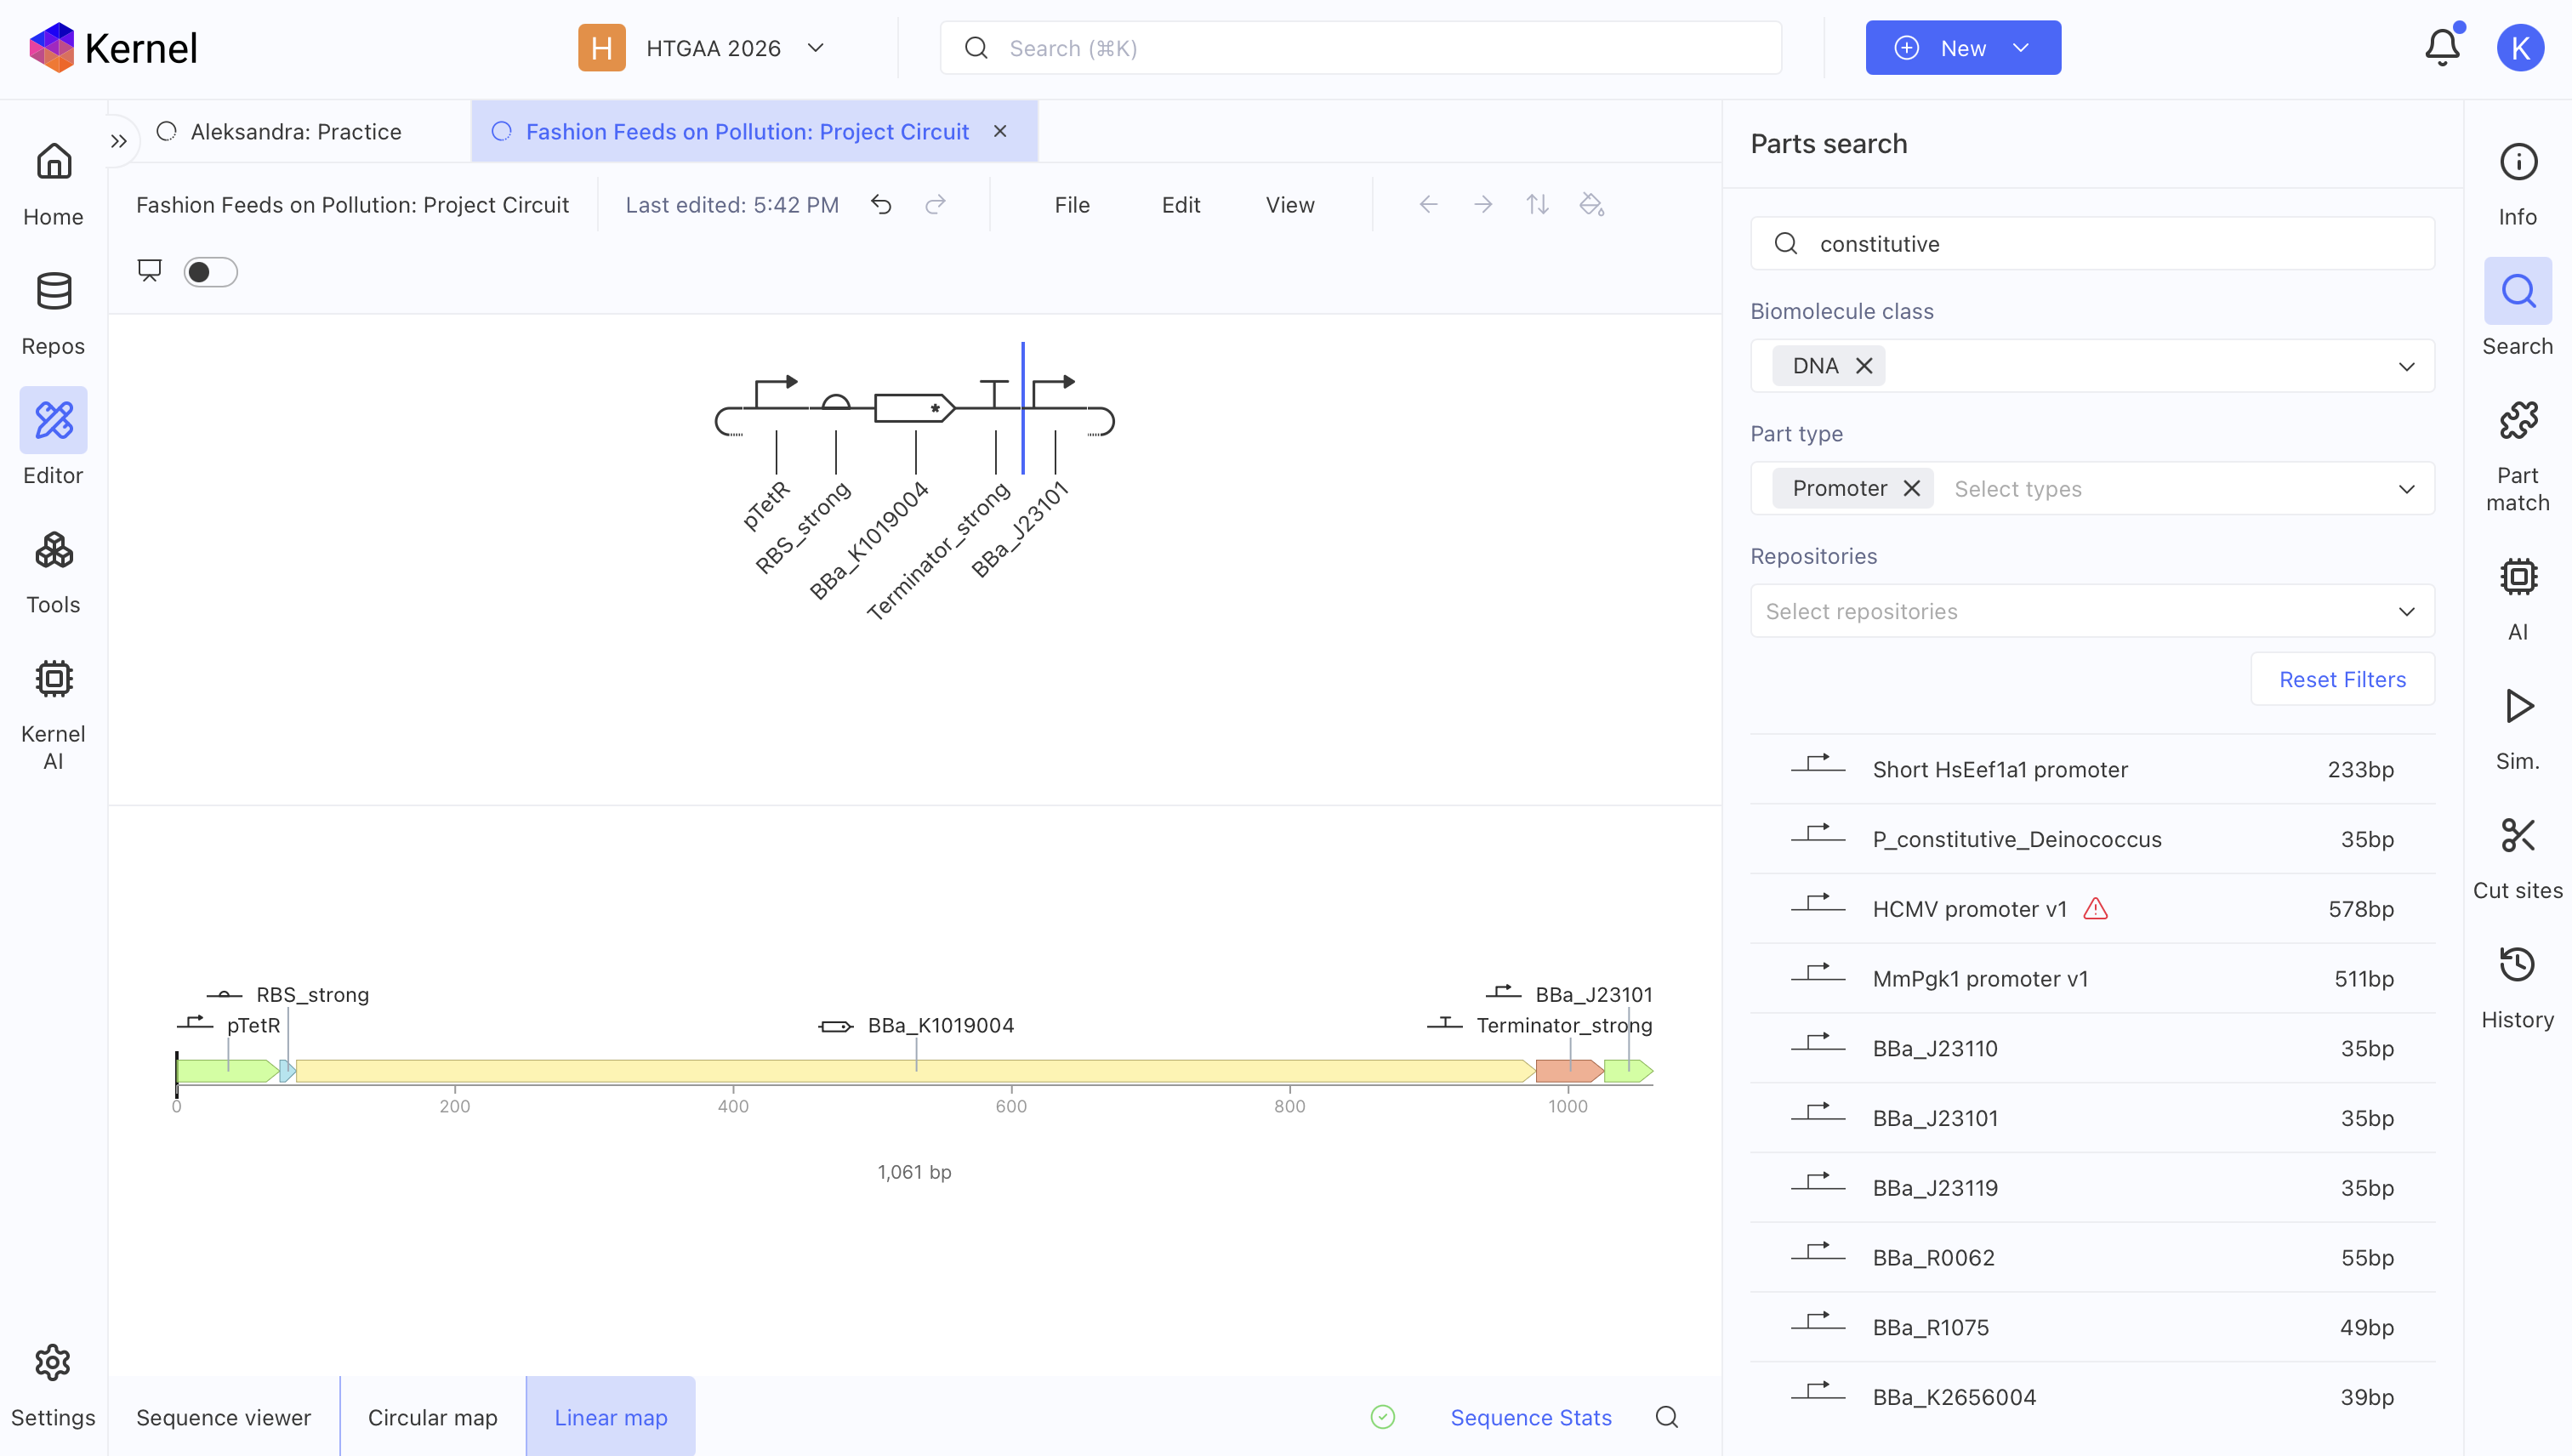
Figure 16. BBa_J23101 selected as the constitutive promoter for the TetR control unit.
A constitutive promoter continuously drives gene expression.
Its role in my circuit was therefore to produce TetR continuously.
Step 6 — Adding an RBS to the Control Unit
I added a second:
RBS_strong

Figure 17. Adding RBS_strong after BBa_J23101.
The second transcriptional unit now began:
BBa_J23101 → RBS_strong → …
Step 7 — Adding the TetR Repressor
Next I added:
TetR
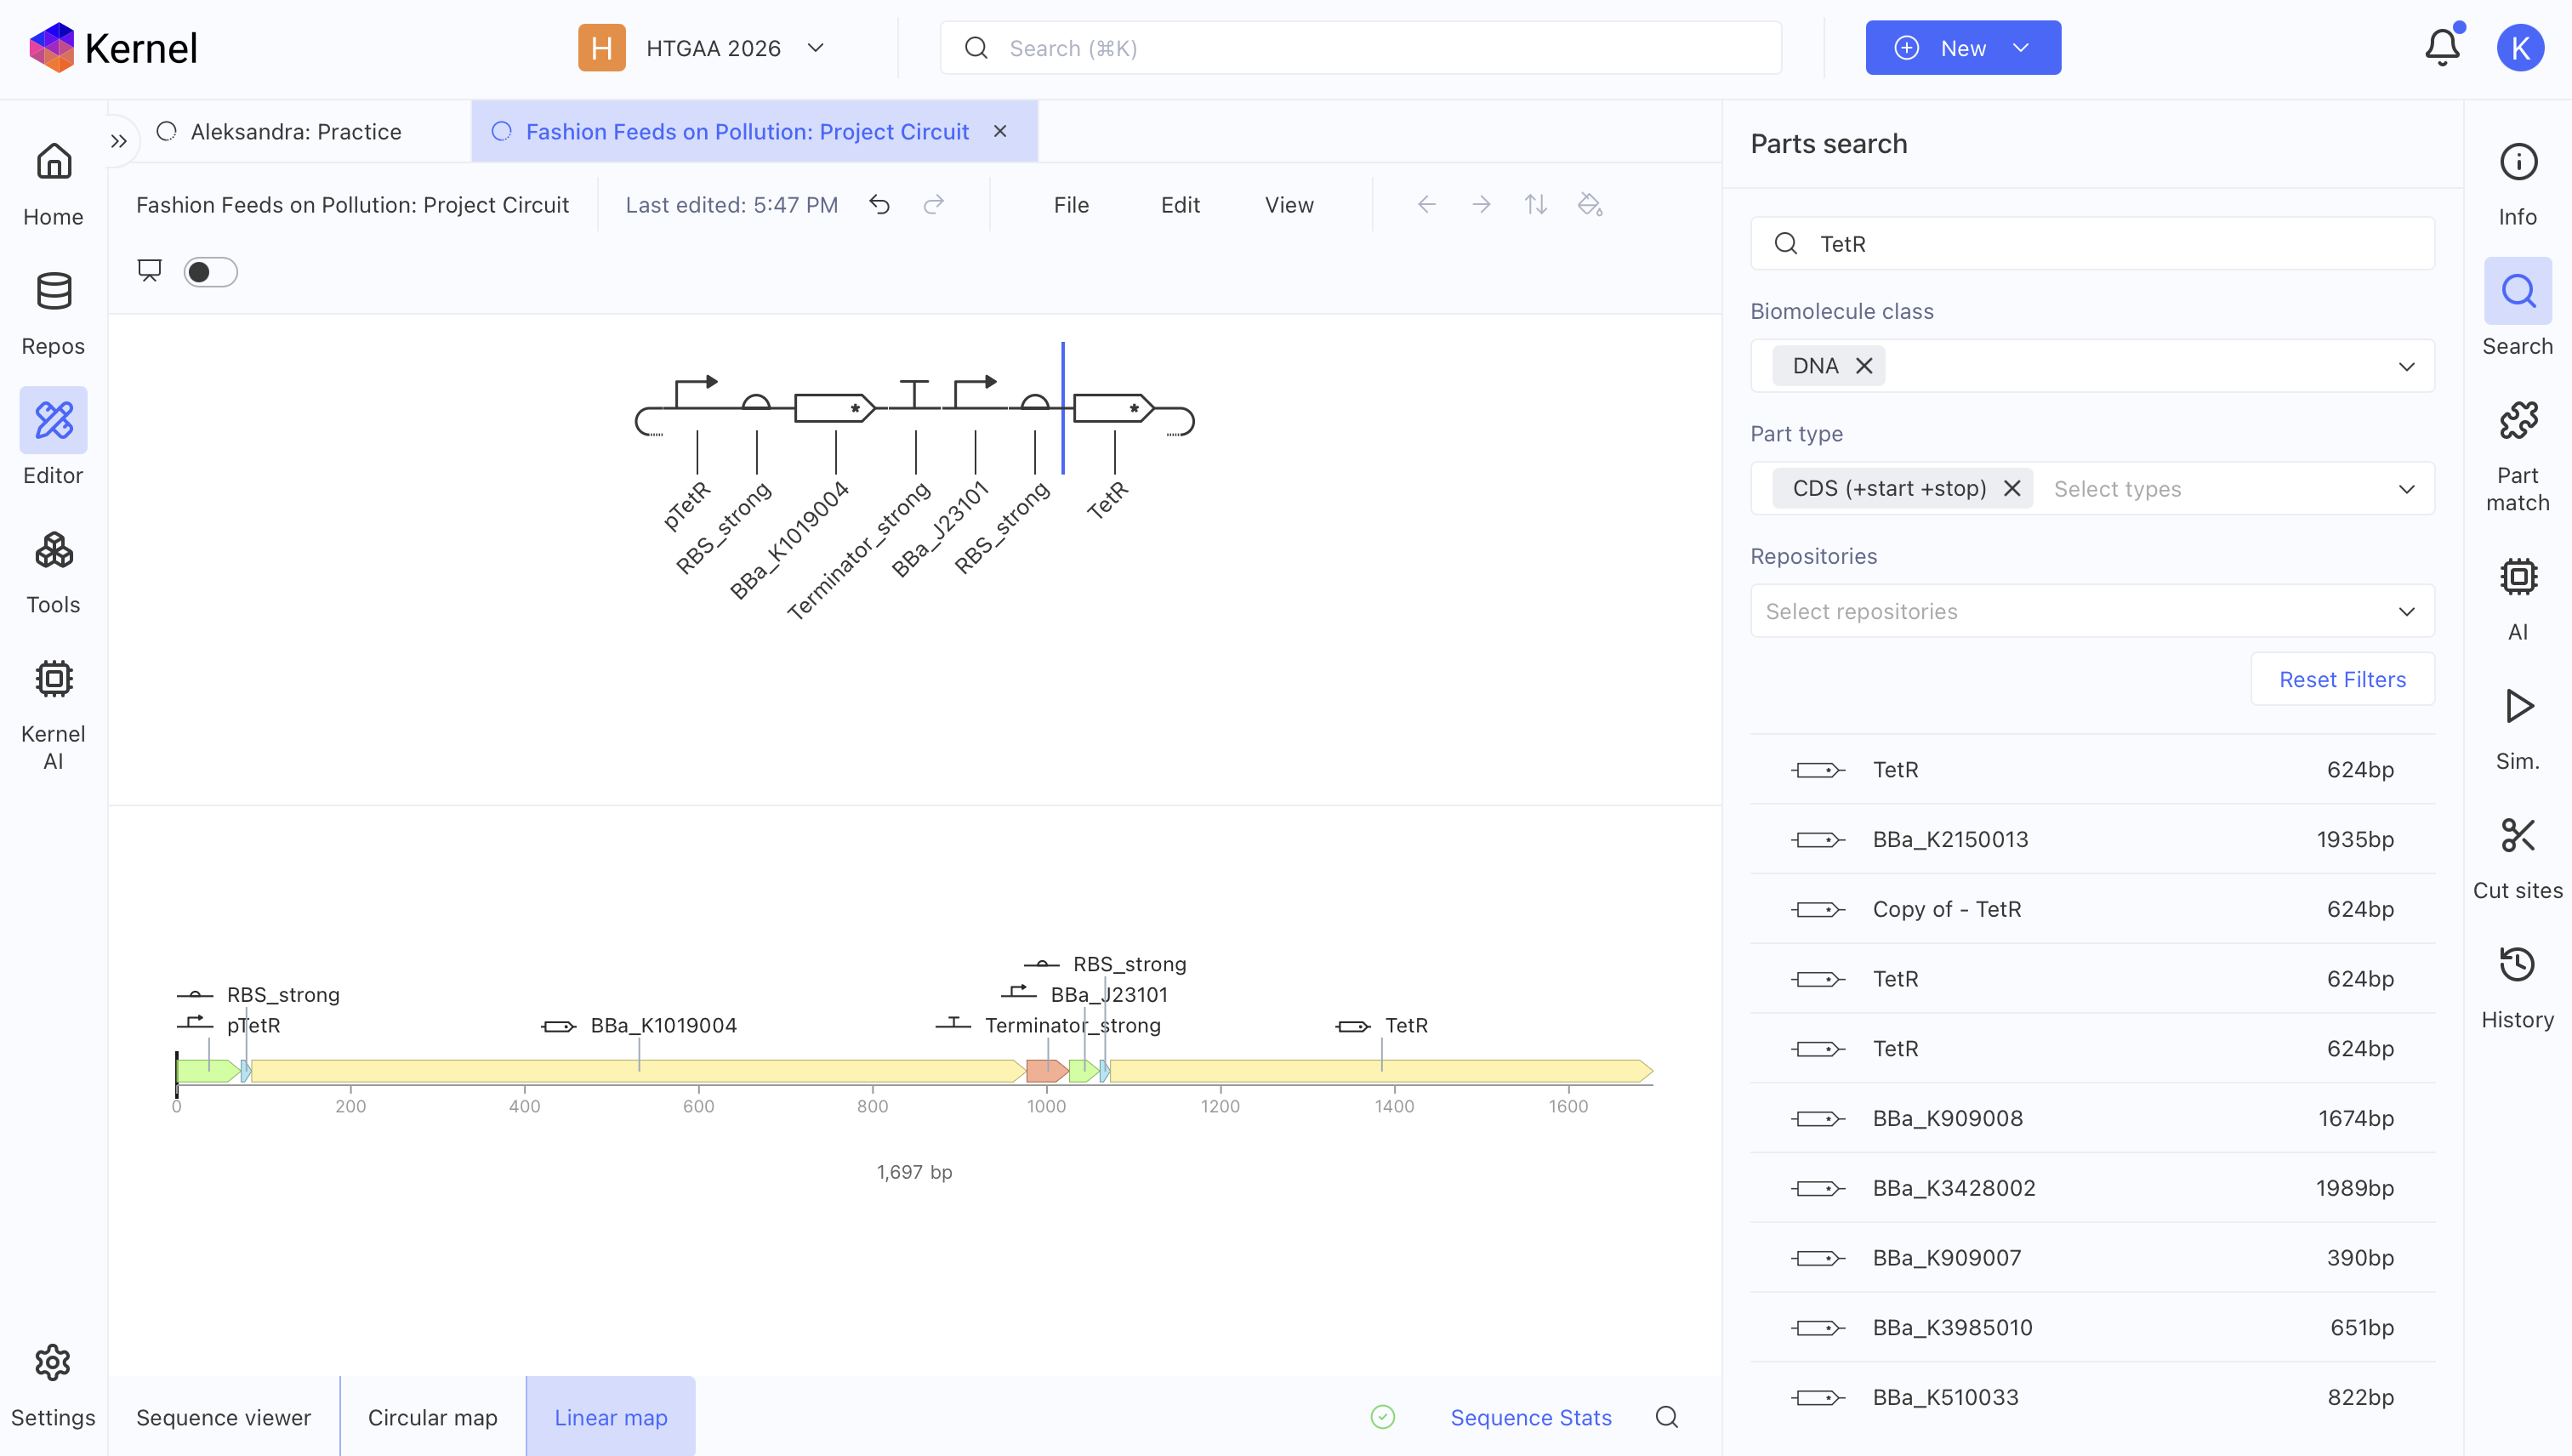
Figure 18. Adding the TetR coding sequence to the control unit.
TetR is the repressor that interacts with TetO operator sequences inside pTetR.
The regulatory relationship becomes:
TetR ┤ pTetR
The circuit now contains two different functions:
PRODUCTION UNIT
pTetR → RBS_strong → YdeH → Terminator
CONTROL UNIT
BBa_J23101 → RBS_strong → TetR → …
Step 8 — Completing the Genetic Switch
Finally, I added another:
Terminator_strong
after TetR.
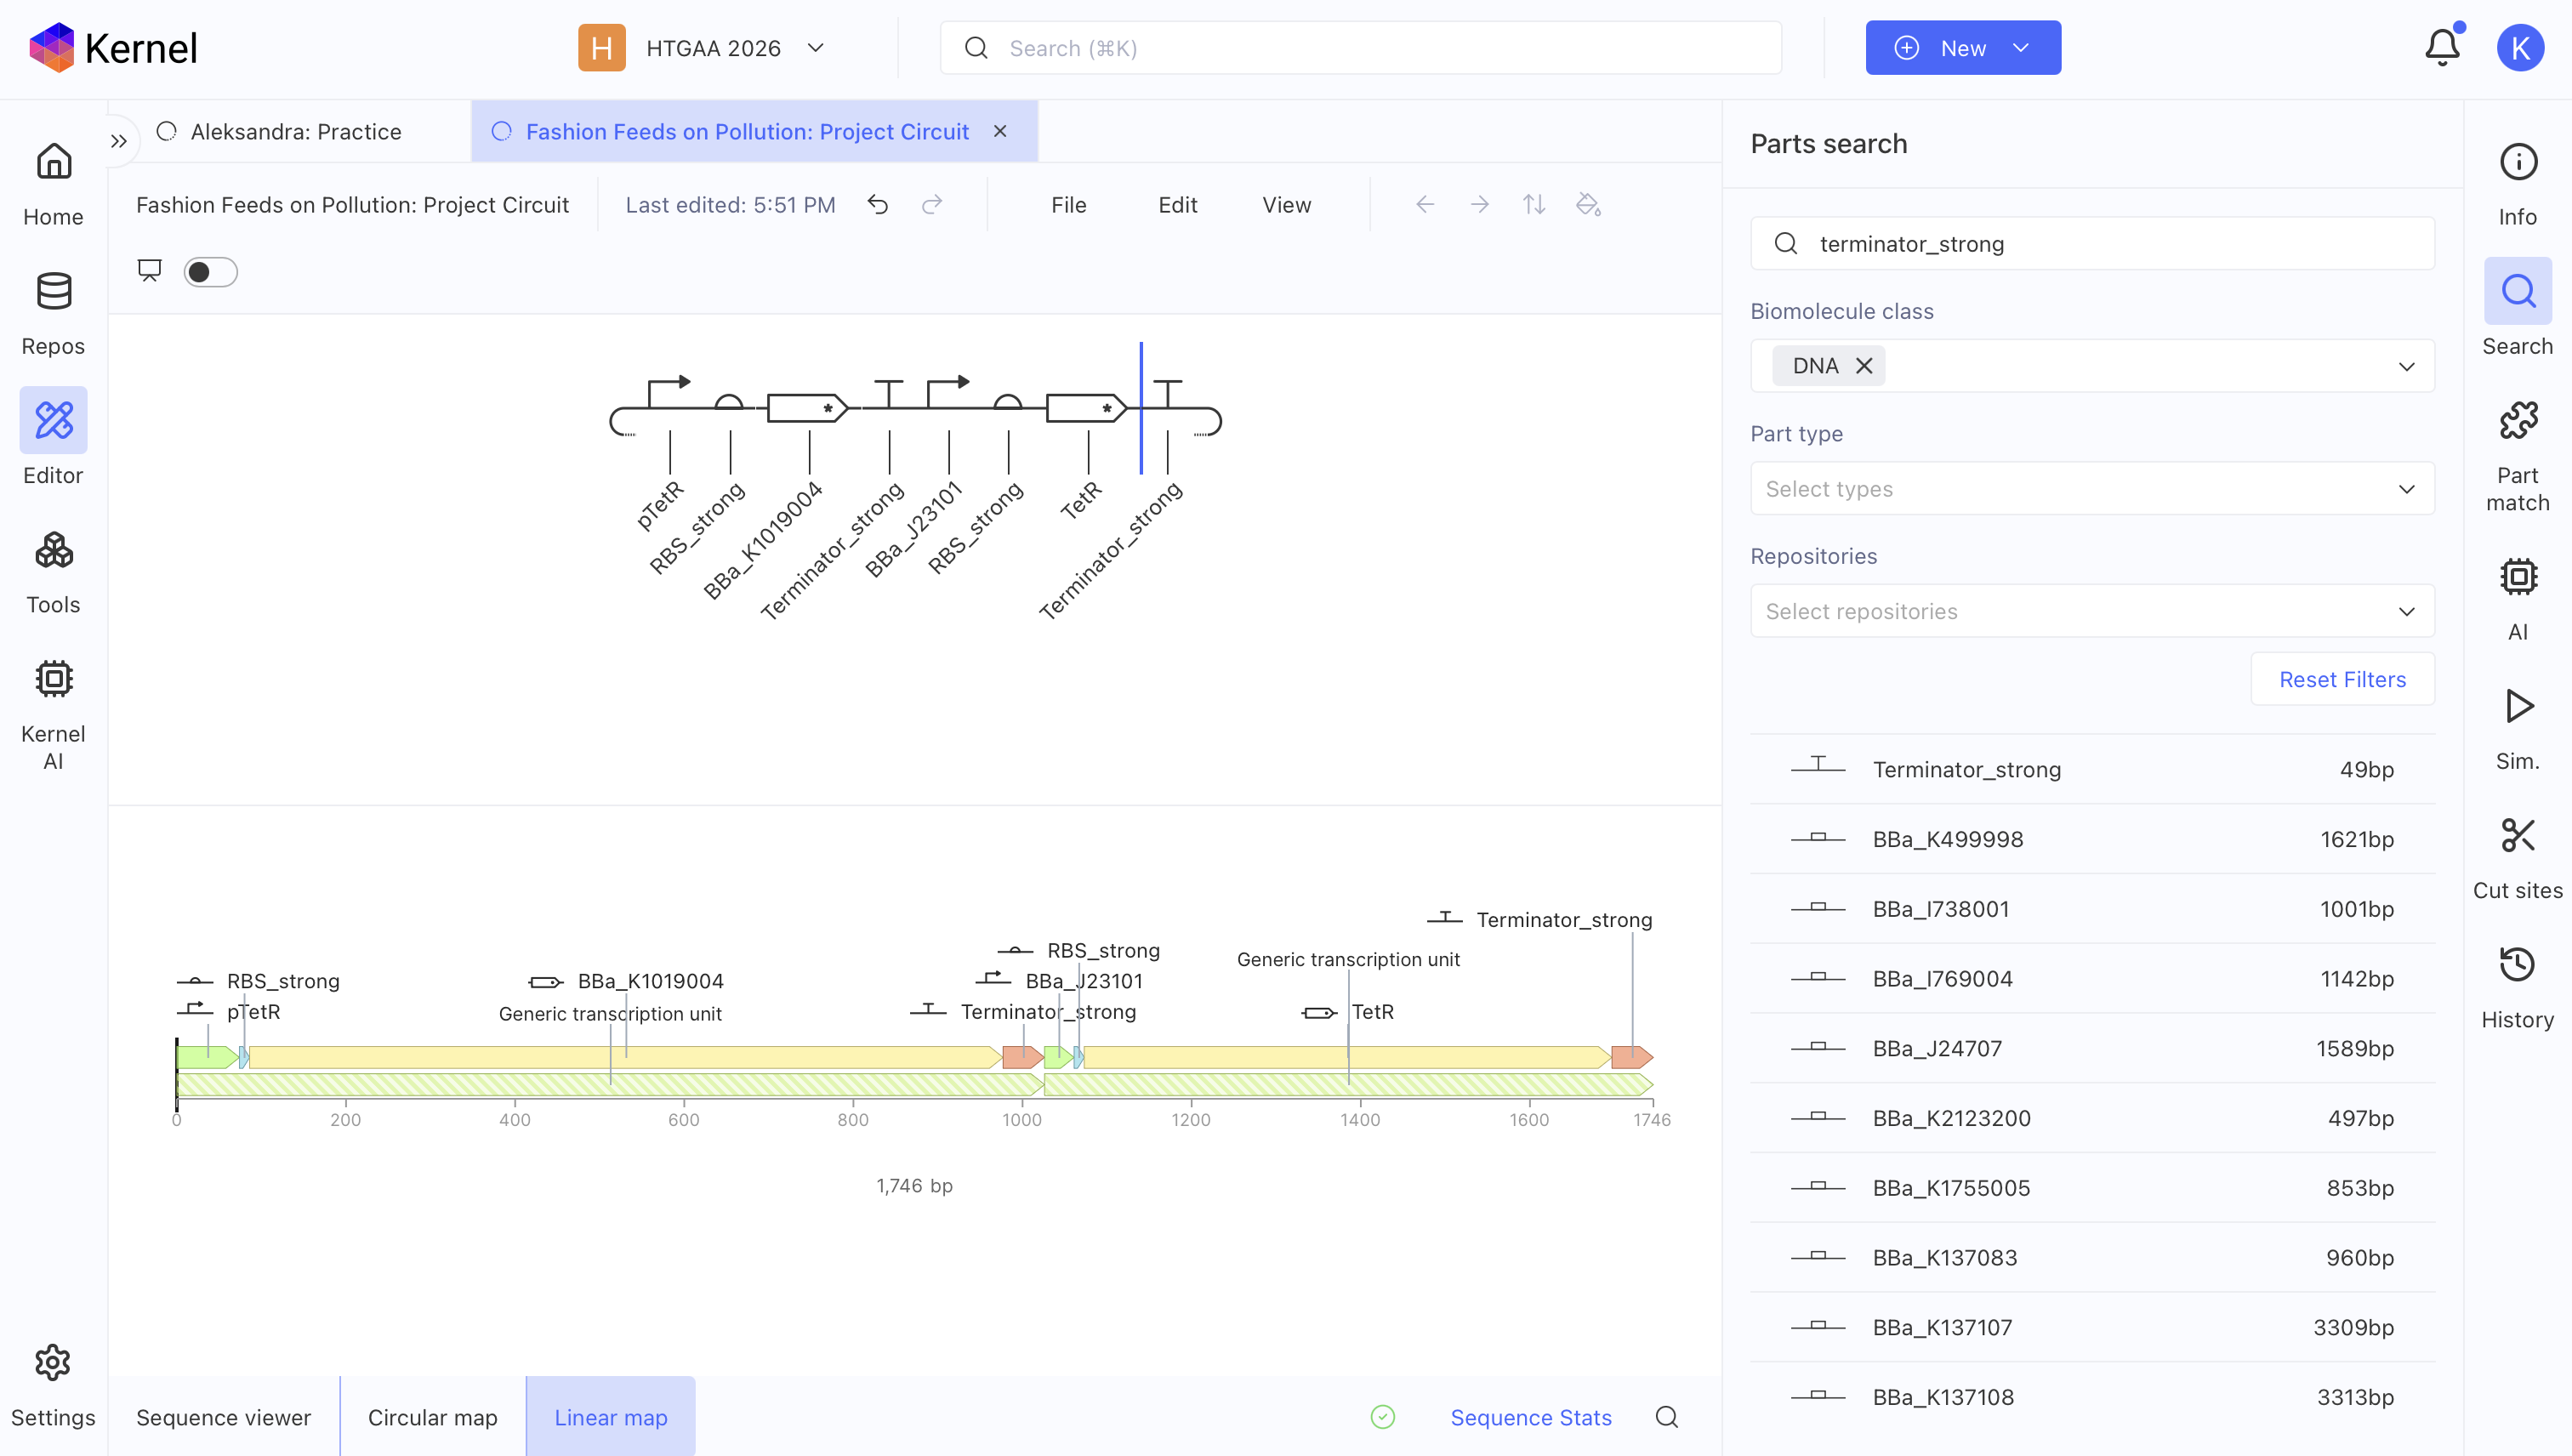
Figure 19. Completed two-unit Fashion Feeds on Pollution genetic circuit.
The complete construct was now 1,746 bp long.
Production unit
pTetR → RBS_strong → YdeH → Terminator_strong
Control unit
BBa_J23101 → RBS_strong → TetR → Terminator_strong
Conceptually:
BBa_J23101 → TetR ┤ pTetR → YdeH
The control unit continuously produces TetR.
TetR can repress pTetR, which controls YdeH expression.
In a future biological system, an induction signal could potentially be used to relieve repression and activate the production state.
For my project, this represents the broader question:
What if methane-consuming cells could first grow and then receive a signal that switches them towards a material-production state?
Testing the Regulatory Circuit
I simulated the complete two-unit circuit using the same conditions as before.
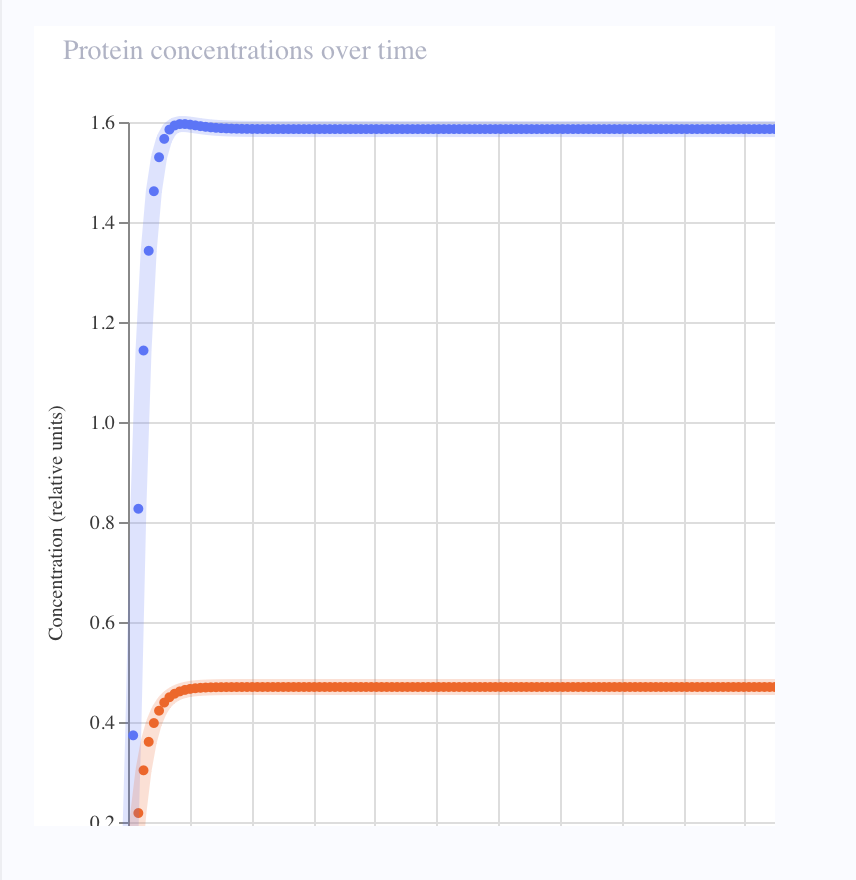
Figure 20. Predicted protein concentrations for the completed regulatory circuit.
The graph produced two protein outputs:
YdeH — blue
approximately 1.6 relative units
TetR — red
approximately 0.47 relative units
Before introducing the TetR control unit, YdeH had reached approximately:
1.8 relative units
With TetR present, YdeH reached approximately:
1.6 relative units
Within the Kernel model, introducing the control unit was therefore associated with a modest reduction in predicted YdeH expression.
Without TetR
pTetR → YdeH
→ YdeH ≈ 1.8
With TetR
TetR ┤ pTetR → YdeH
→ YdeH ≈ 1.6
This was not a complete OFF state.
However, it gave me a computational way to start testing the regulatory logic of the circuit.
Redesigning the Control Unit
I then tested whether changing one component of the control unit would produce a clearer difference between the two states.
First, I replaced the TetR coding sequence with the matching TetR part from Kernel’s Characterized Bacterial Parts collection.
The predicted concentrations remained almost unchanged:
- YdeH ≈ 1.6
- TetR ≈ 0.47
Changing the TetR sequence itself therefore did not substantially alter the simulation.
I moved to another design variable:
the promoter controlling TetR expression
Redesign — Changing the TetR Promoter
The original control unit used:
BBa_J23101 → RBS_strong → TetR → Terminator
I replaced BBa_J23101 with another constitutive promoter from the same Anderson promoter family:
BBa_J23119
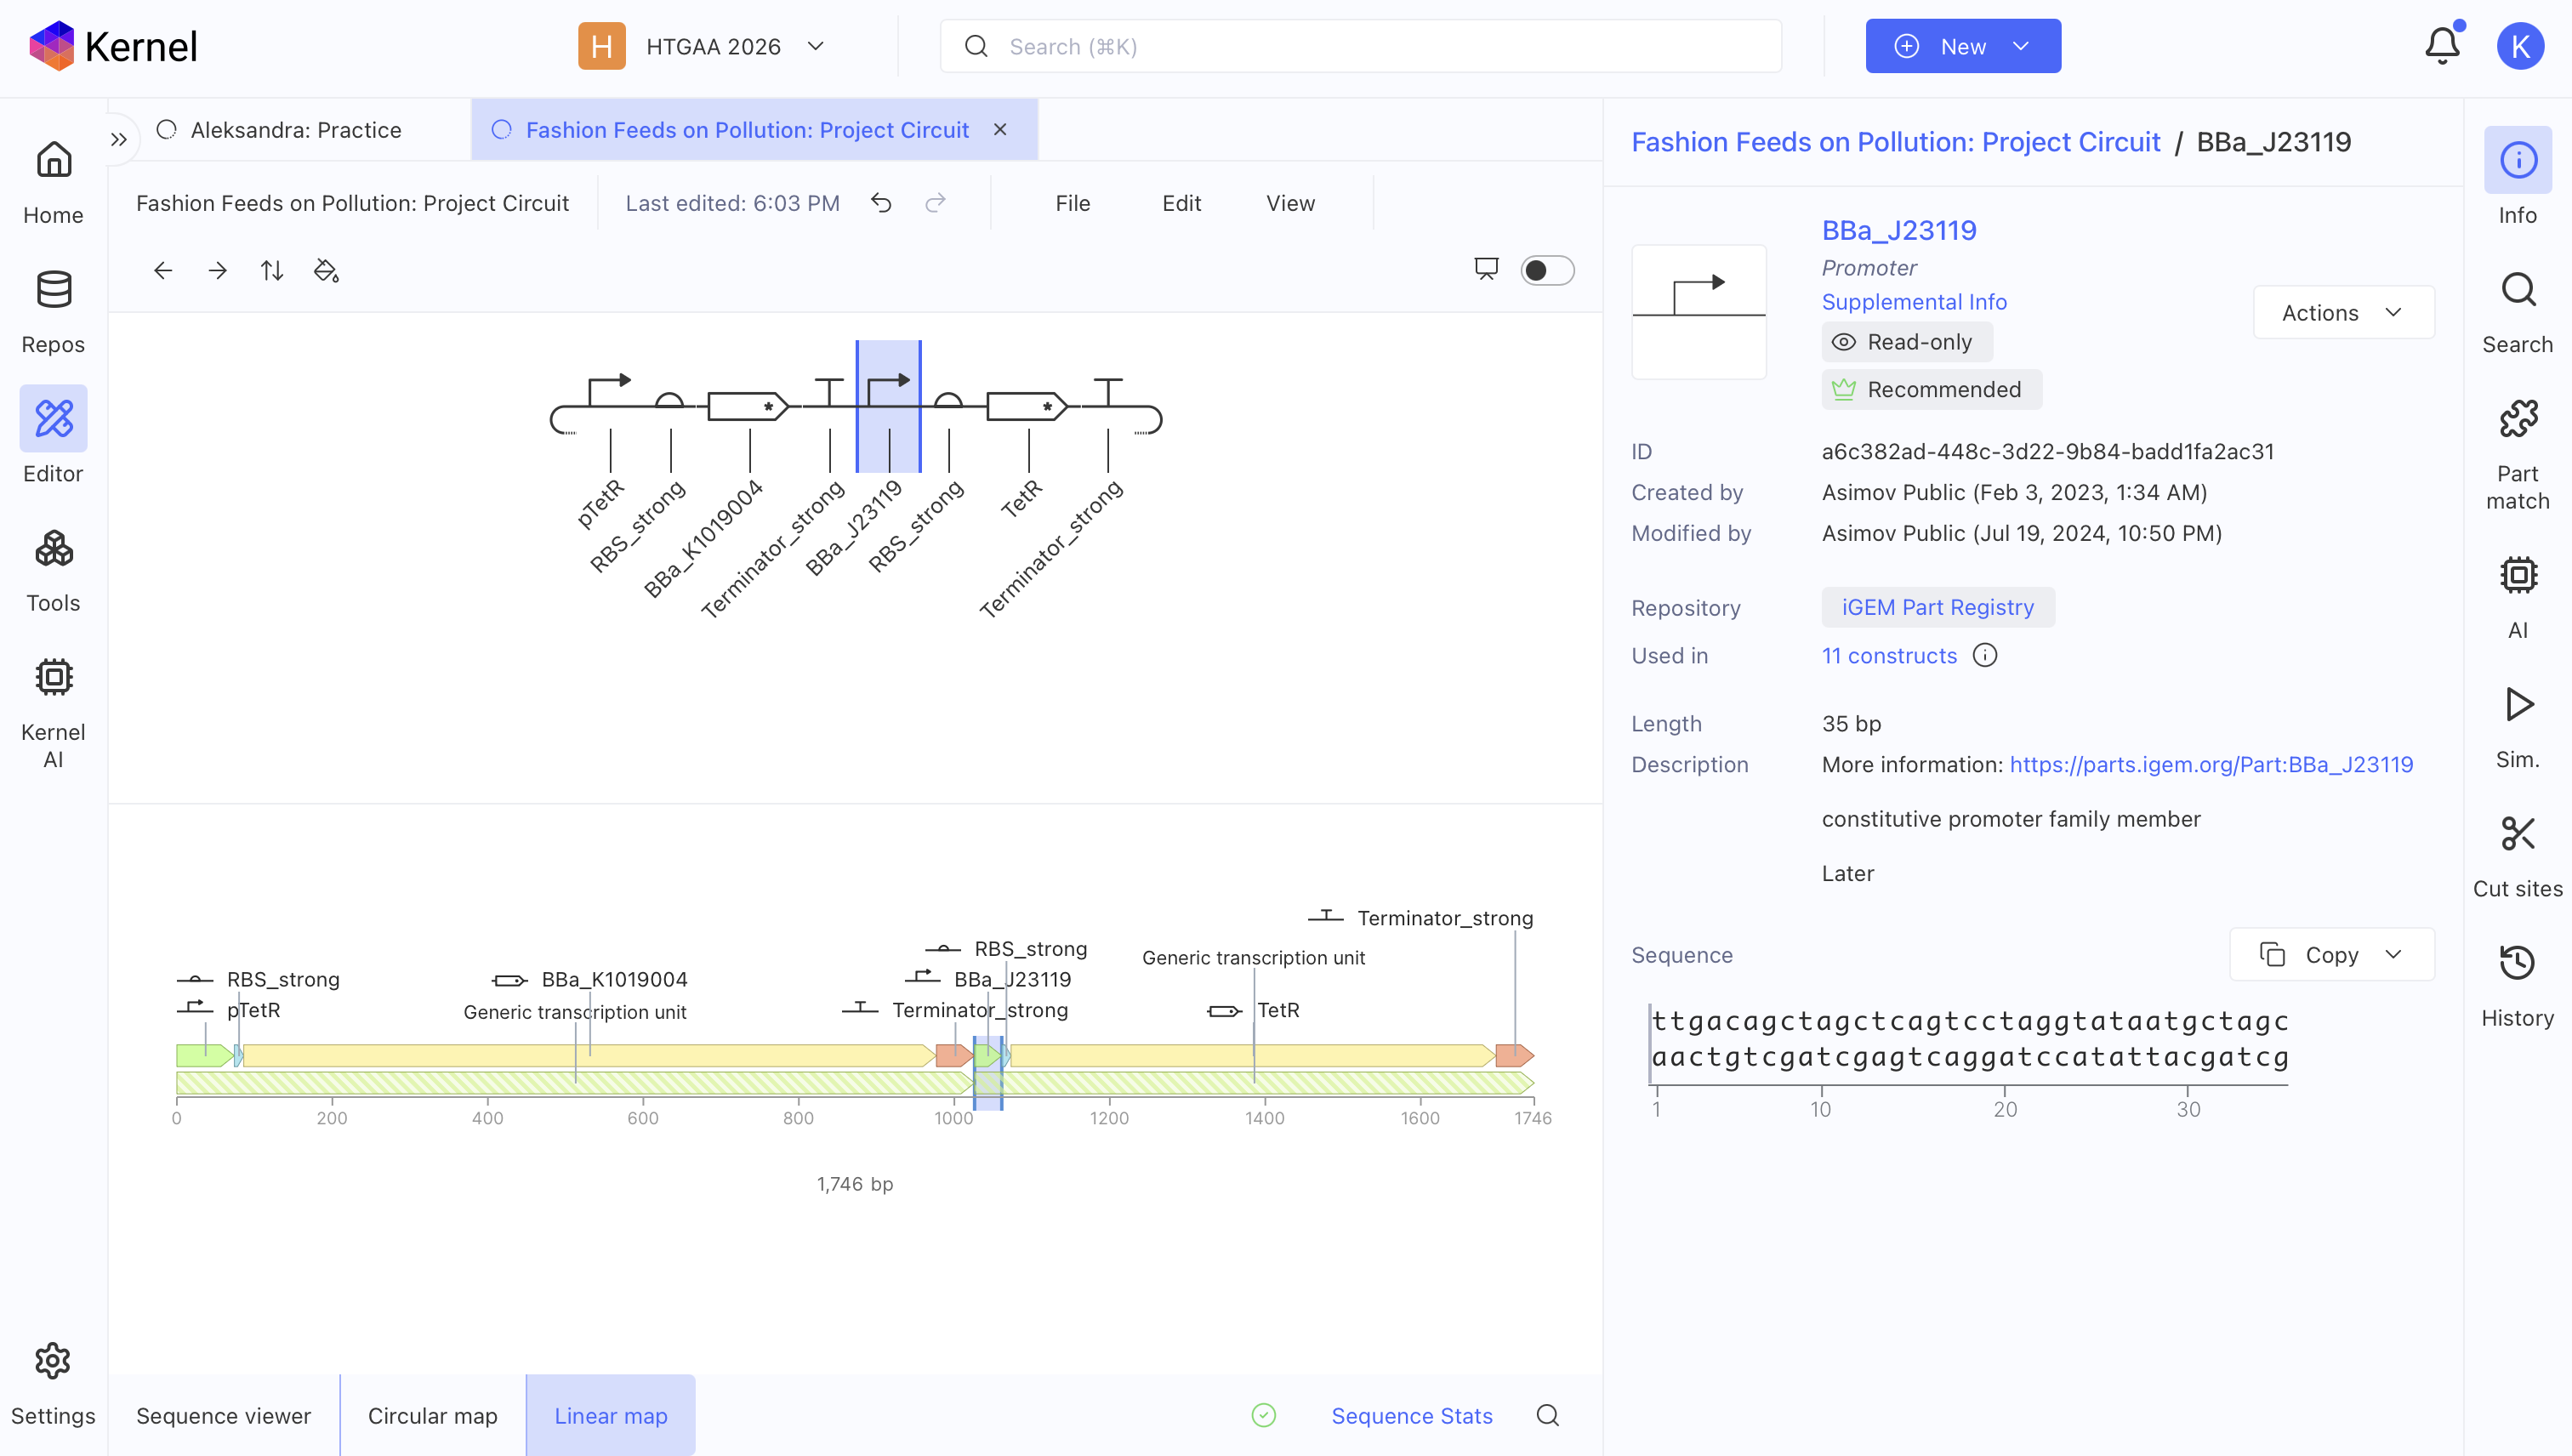
Figure 21. BBa_J23119 selected as an alternative promoter for the control unit.
Rather than assuming that J23119 would improve the circuit, I treated the replacement as an experiment.
The redesigned unit became:
BBa_J23119 → RBS_strong → TetR → Terminator
The question was:
Will changing the promoter driving TetR alter repression of the YdeH production unit?
Testing the Redesign
I repeated the simulation under the same conditions.
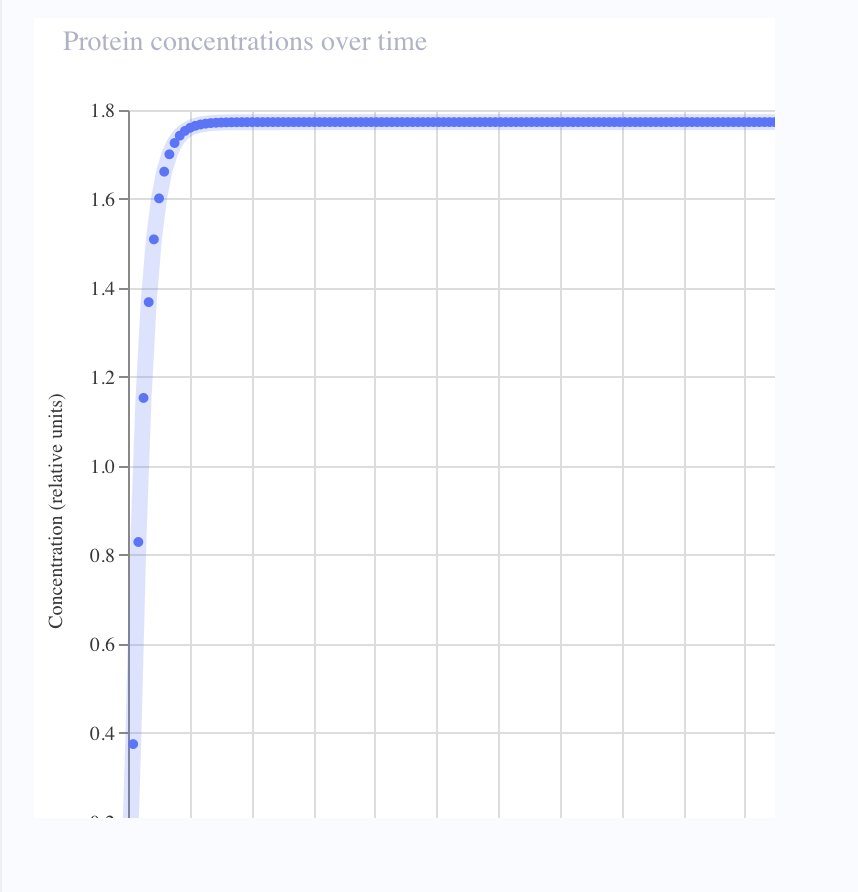
Figure 22. Protein-concentration simulation after replacing BBa_J23101 with BBa_J23119.
The predicted YdeH concentration reached approximately:
1.78 relative units
This was higher than the approximately 1.6 relative units predicted with J23101 and very close to the approximately 1.8 relative units observed before adding the TetR control system.
The redesign therefore did not improve repression in the Kernel model.
My three iterations produced:
| Design | Predicted YdeH |
|---|---|
| No TetR control unit | ~1.8 |
| J23101 → TetR | ~1.6 |
| J23119 → TetR | ~1.78 |
For this model, the J23101 architecture produced the clearest reduction in predicted YdeH expression.
I therefore returned to J23101 for the final construct.
This was useful because it showed me that DNA design is not simply about choosing a part that sounds stronger.
The behaviour of the whole system has to be tested.
Final Circuit
My final exploratory circuit is:
Production unit
pTetR → RBS_strong → BBa_K1019004 / YdeH → Terminator_strong
Control unit
BBa_J23101 → RBS_strong → TetR → Terminator_strong

Figure 23. Completed final Fashion Feeds on Pollution circuitt in Kernel.
The complete construct is:
1,746 bp
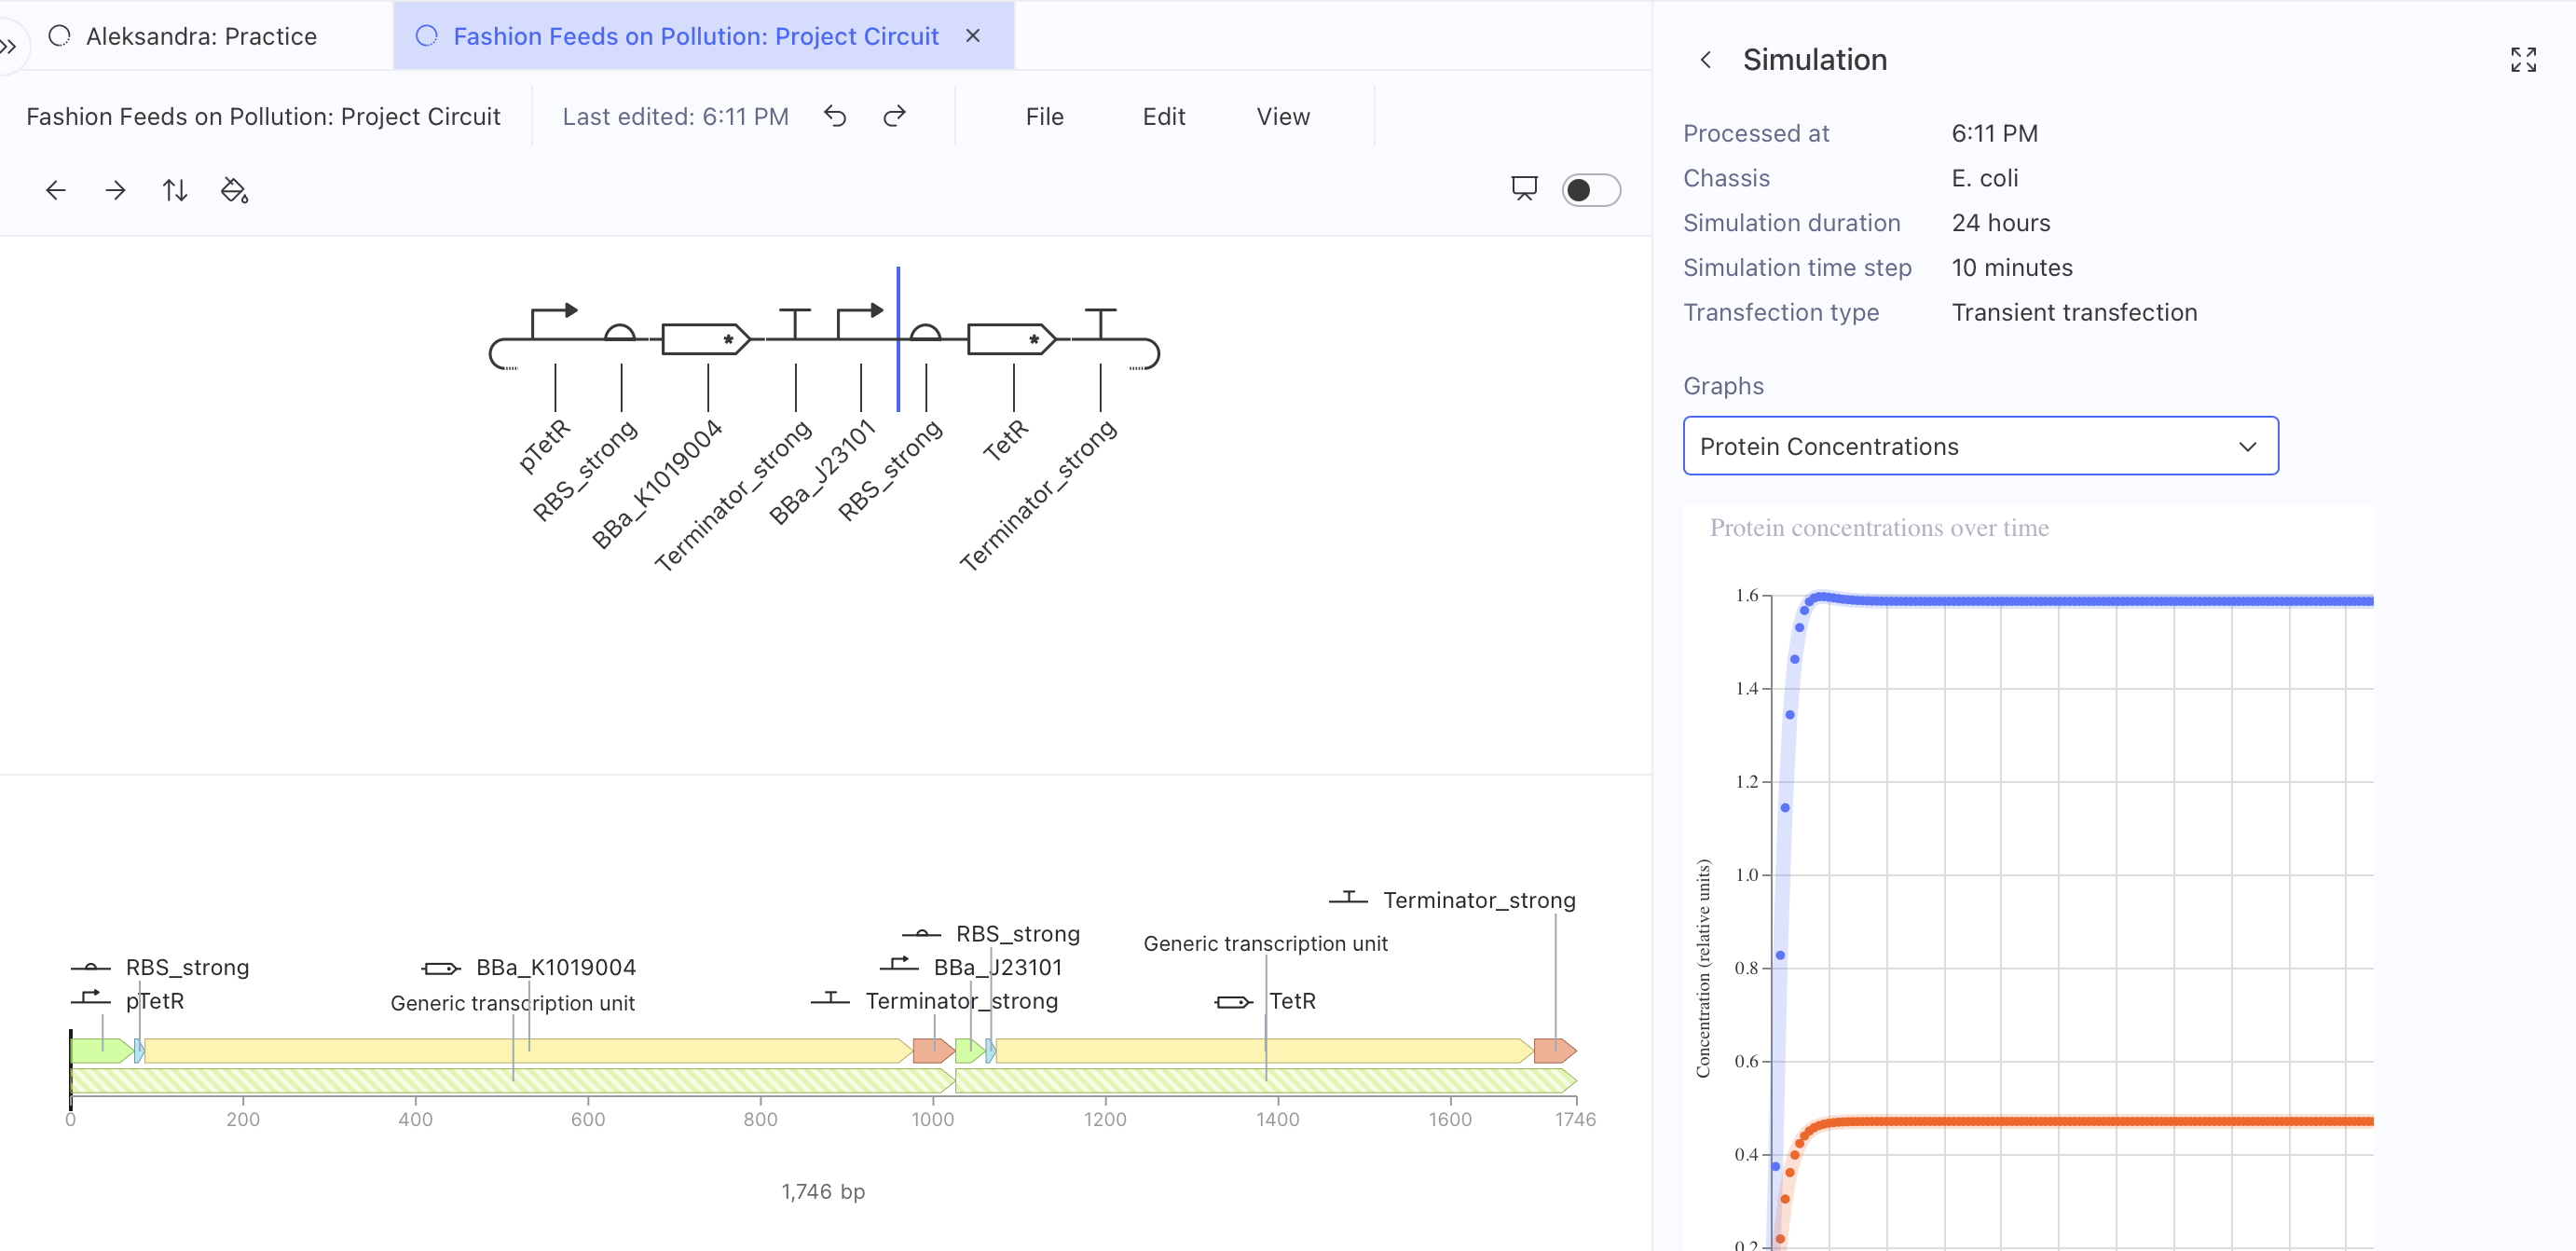
Figure 24. Final Fashion Feeds on Pollution circuit and protein-concentration simulation in Kernel.
The final simulation predicted:
YdeH ≈ 1.6 relative units
TetR ≈ 0.47 relative units
The production of TetR was associated with a modest reduction in predicted YdeH expression compared with the first circuit without the TetR control unit.
This is not a complete ON/OFF switch.
It is a first computational exploration of how a regulatory architecture might influence expression of a candidate material-production regulator.
Design → Test → Redesign
The most useful part of this exercise was not creating one supposedly “correct” circuit.
It was moving through iterations.
1 — LEARN
pLacI → RBS → GFP → Terminator
I learned the basic vocabulary of genetic circuits.
2 — TRANSLATE
pTetR → RBS → YdeH → Terminator
I connected the exercise to my material-production hypothesis.
3 — ADD CONTROL
BBa_J23101 → RBS → TetR → Terminator
I added a second transcriptional unit capable of regulating the first.
4 — TEST
The simulation changed predicted YdeH expression from approximately 1.8 → 1.6.
5 — REDESIGN
I changed J23101 to J23119.
Predicted YdeH increased again to approximately 1.78.
6 — LEARN
I returned to the J23101 architecture.
My process became:
DESIGN → TEST → LEARN → REDESIGN → COMPARE
This is very close to the way I already understand innovation strategy: a proposed solution is not valuable because it sounds convincing, but because assumptions can be made visible and tested.
What Does This Mean for Fashion Feeds on Pollution?
The circuit does not prove that I can genetically engineer a flexible methane-derived fashion material.
Instead, it represents an early biological hypothesis behind the project.
AirCarbon shows that greenhouse-gas carbon can become a biologically produced material.
The Girona research shows that Methylotuvimicrobium alcaliphilum 20Z can produce extracellular polymeric substances directly from methane.
My project asks:
What if that extracellular production pathway could eventually be biologically controlled and developed specifically towards flexible material properties?
The circuit designed this week begins to investigate the control part of that question.
Conceptually:
TetR regulates pTetR
↓
pTetR controls YdeH expression
↓
YdeH represents a hypothesis for modifying c-di-GMP signalling associated with extracellular-matrix production
The next biological question is therefore:
Would manipulating this type of regulatory pathway actually change the amount or composition of methane-derived EPS in M. alcaliphilum?
Only after that question is answered would the project move towards material development:
BIOLOGY → EPS → RECOVERY → FORMULATION → FLEXIBILITY TESTING → FASHION
Limitations
This circuit is an exploratory computational model, not a validated genetic system for Methylotuvimicrobium alcaliphilum.
Kernel simulated the construct using:
E. coli
rather than my intended methanotroph.
Several components are also being used as proxies for the regulatory architecture I ultimately want to investigate.
Most importantly:
YdeH has not been demonstrated to regulate the specific protein-rich methane-derived EPS reported by the Girona research team.
YdeH is an experimentally supported diguanylate cyclase in E. coli, and c-di-GMP has an established role in regulating multiple bacterial exopolysaccharide systems.
Connecting this mechanism to the EPS of M. alcaliphilum is therefore a hypothesis, not an established fact.
That uncertainty is not something I want to hide.
It defines the next research question.
Future work would require identifying candidate regulatory pathways directly in M. alcaliphilum, potentially using transcriptomic data collected under different methane and EPS-producing conditions.
What I Learned
Before this week, promoters, RBSs, coding sequences, repressors and terminators were mostly new concepts to me.
Using Kernel helped me understand them visually as parts of a system rather than as isolated biological terminology.
The biggest shift was understanding that DNA design is not simply about selecting a gene.
It is about designing relationships between biological instructions.
I started the week asking:
How do I make a cell produce something?
I finished it asking:
How could I control when and how a cell produces a material?
That is where DNA design begins to connect with my existing background in innovation, systems thinking and material design.
References
Aranda, A., Primo-Catalunya, D., Sánchez-Melsió, A., Balcázar, J. L., & Pijuan, M. (2026). Exploring the capabilities of Methylotuvimicrobium alcaliphilum 20Z to produce exopolymeric substances from methane. Enzyme and Microbial Technology, 199, 110893.
https://doi.org/10.1016/j.enzmictec.2026.110893
Asimov. (2026). Kernel Documentation.
https://docs.kernel.asimov.com/
Goswami, S., Singer, S. W., Simmons, B. A., & Awasthi, D. (2024). Optimization of electroporation method and promoter evaluation for type-1 methanotroph, Methylotuvimicrobium alcaliphilum. Frontiers in Bioengineering and Biotechnology, 12, 1412410.
https://doi.org/10.3389/fbioe.2024.1412410
HTBAA 2026. (2026). DNA Design / Kernel introduction and genetic circuit design lecture. How to Grow (Almost) Anything, MIT.
Newlight Technologies. (n.d.). AirCarbon.
https://www.newlight.com/aircarbon
Poulin, M. B., & Kuperman, L. L. (2021). Regulation of biofilm exopolysaccharide production by cyclic di-guanosine monophosphate. Frontiers in Microbiology, 12, 730980.
https://doi.org/10.3389/fmicb.2021.730980
Zähringer, F., Massa, C., & Schirmer, T. (2011). Efficient enzymatic production of the bacterial second messenger c-di-GMP by the diguanylate cyclase YdeH from E. coli. Applied Biochemistry and Biotechnology, 163(1), 71–79.
https://doi.org/10.1007/s12010-010-9017-x
AI Use
I used ChatGPT as a learning, research and documentation assistant while completing this assignment.
As I am approaching synthetic biology from an innovation and design background rather than molecular biology, I used AI primarily to:
- explain unfamiliar biological terminology in accessible language;
- understand the Kernel workflow;
- distinguish between experimentally supported biology and speculative project hypotheses;
- identify relevant literature;
- connect DNA design to my methane-to-material research question;
- structure and edit my documentation.
Examples of prompts included:
“Explain a promoter, RBS, CDS and terminator in simple terms.”
“Help me connect a simple bacterial circuit to my methane-to-material research without inventing biological mechanisms.”
“What does the Kernel protein-concentration simulation actually show, and what can I reasonably conclude from it?”
“Compare my circuit iterations and help me document the Design → Test → Redesign process.”
Scientific claims were checked against the course material and the references listed above. AI-generated suggestions were treated as starting points for research rather than as experimental evidence.