Hello, My name is Mohammedhussein, but you can call me Hussein!
I am a medical doctor practising since 2020 and I took internal medicine residency. Now plannig to move to germany to live and work there.
I have a growing interest in molecular biology, genetics, biotech and regenerative medicine, the reason is that I believe these fields helps with the innovation and finding more solutions in medicine and clinical practice.
Iam so happy to get accepted in the program and glad to get to know the participants!
My contact infos ar below.feel free to communicate with me
{{Email: husseinem95@gmail.com-
Instagram: @hussein.bnb}} Contact info
Homework, Labs, and Projects
See the nav bar on the left to look through my work for How To
Biomanufacture Almost Anything (Fall 2026)!
Subsections of <Mohammedhussein Albaghdadi> — HTBAA Fall 2026
Week 1 HW: Final Project Ideas
What you would like to biomanufacture and why?
Target Product:
Rapid, on-demand recombinant human desB30-insulin (a fully functional, active 51-amino-acid insulin analog with an intact disulfide architecture missing only ThrB30).
Intended Users:
Diabetic patients in low- and middle-income regions, remote clinical sites, or emergency crisis zones facing acute medicine supply chain disruptions.
Motivation & Importance:
Over 96% of the global insulin volume is monopolized by three pharmaceutical conglomerates, resulting in inflated pricing, chronic rationing (affecting 1.3 million Americans alone), and clinic availability dropping as low as 55% in LMICs.
Conventional cell-based biomanufacturing relies on centralized multi-thousand-liter bioreactors and requires weeks to extract, denature, refold, sulfitolyze, and polish insulin from E. coli inclusion bodies.
By producing therapeutic-grade mature insulin locally in under 24 hours, a point-of-care cell-free platform decentralizes biomanufacturing, bypassing cold-chain fragility and single-supplier bottlenecks.
What Living System Would You Use?
Chassis Platform: A purified E. coli-derived cell-free protein synthesis (CFPS) chassis (PUREfrex® 2.1) coupled to an on-column enzymatic conversion matrix.
System Inputs: Linear or plasmid DNA encoding an engineered proinsulin precursor construct (His-R-IP; ~10.85 kDa). 36 purified E. coli transcription and translation enzymes, ribosomes, tRNAs, amino acids, and NTPs (void of endogenous proteases/peptidases).
Downstream reagents: Immobilized Metal Affinity Chromatography (IMAC) Ni-NTA resin and sequencing-grade trypsin.
Biological & Biochemical Processes:
Transcription/Translation & Assisted Folding: T7 RNA polymerase transcribes the plasmid, and ribosomal machinery translates the construct. DsbC alongside Skp/FkpA stabilizes nascent hydrophobic regions (e.g., A13–A19, B9–B19) to correctly orchestrate native disulfide bridges ($A7\text{–}B7$, $A20\text{–}B19$, and $A6\text{–}A11$) while preventing irreversible aggregation.
Affinity Capture: The N-terminal $6\times\text{His}$ tag captures soluble proinsulin onto a Ni-NTA matrix without prior cell lysis or inclusion body denaturation.
On-Column Digestion: Reconstituted trypsin cleaves at the engineered Arg13 and the C-peptide flanking dibasic cleavage sites. An engineered K78A mutation eliminates unwanted side-products like Arg-A0-insulin.
System Outputs: Mature human desB30-insulin (~5,717 Da) and cleaved by-products ($6\times\text{His}$ leader, C-peptide).
How would you use automation?
Prototyping Stage (Bench Screening & Optimization): A desktop liquid-handling robot (e.g., Opentrons OT-2 / Flex) automates micro-scale titration arrays (chaperone stoichiometry, redox ratios, DNA templates, and trypsin digestion times) directly into 96-well plates to maximize active monomer fractions.
An automated, closed-loop microfluidic synthesis and purification device (such as the Bio-MOD platform).
Workflow Automated:** Automated metering and fluidic mixing of lyophilized cell-free extract with DNA and chaperone reconstitution buffers.
Temperature-controlled incubation ($37^\circ\text{C}$ for 16 hours).
Pressure-driven solid-phase loading across a single-use Ni-NTA affinity column.
Timed perfusion of trypsin digestion buffers (2.5 hours at $37^\circ\text{C}$), followed by automated low-pH quenching and elution.In-line spectrophotometric QA/QC and flow-through sterile filtration.
4. Scale and Production Timeline Calculations
(a) How Much?
Defined Clinical Scope: Emergency localized supply for a regional clinic supporting 1,000 insulin-dependent diabetic patients for 30 days.
Dosage Assumptions (Borhani et al., 2025):Average daily therapeutic dose per patient $\approx 1.4\text{ mg}$ (equivalent to ~40 IU).
(b) How long: about 20 hours
Empirical Process Yields from Literature (Borhani et al., 2025):
Overall on-column capture and conversion efficiency $= 9.7%$.
Net mature desB30-insulin yield per liter:$$\text{Net Yield} = 0.0351\text{ g/L} \times 0.097 \approx 0.0034\text{ g/L} = 3.4\text{ mg/L}$$
Production Time Calculation:
Batch Cycle Time per Run:CFPS Reaction: $16.0\text{ hours}$
Column Capture & Wash: $0.75\text{ hours}$
On-Column Trypsin Digestion: $2.5\text{ hours}$
Elution & CEX Polishing: $0.75\text{ hours}$
Total Cycle Time $\approx \mathbf{20\text{ hours}}$.
What don’t you know yet?
Unintended Divalent Cation Chelation on Ni-NTA: Mature desB30-insulin retained unexpected affinity for the Ni-NTA column following cleavage due to endogenous metal-coordinating residues (HisB10, GluB13), demanding an imidazole elution step instead of purely autonomous release. Shifting to an orthogonal capture chemistry (e.g., Strep-Tag II / Strep-Tactin) must be experimentally validated.
Co-Chaperone Antagonism and Low Conversion Efficiency (9.7%): Combining Skp and FkpA resulted in lower monomer yields than Skp alone, and significant product was lost to non-covalent proinsulin-insulin heterodimers (~16.7 kDa) and incomplete cleavage intermediates. Optimizing the trypsin-to-protein ratio and introducing β-trypsin variants will require systematic kinetic screening.
Oxygenation and Mass Transfer Scaling Limitations: Scaling cell-free reactions above micro-volumes often leads to titer drop-offs due to insufficient surface-area-to-volume ratios and oxygenation constraints necessary for energy cofactor regeneration. Overcoming this requires testing thin-film, bubble-free, or microfluidic bioreactor geometries.
AI Used
Gemini pro
Week 2 HW: DNA Design
Part 1: Expression target
Molecule: A tagged proinsulin precursor called His-R-IP (10.85 kDa; theoretical mass 10,848 Da). It is converted on a Ni-NTA column into the mature product, desB30-insulin (about 5.7 kDa).
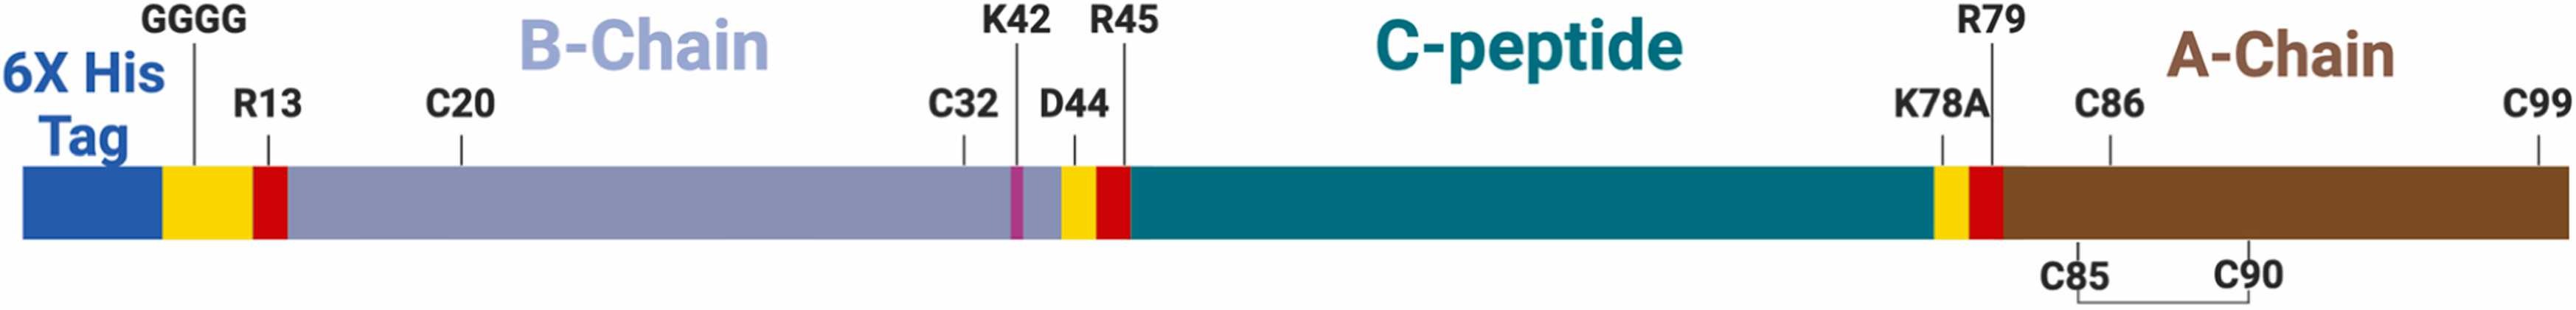
Sequence: The construct is derived from human proinsulin >(UniProt P01308), with these changes (Fig. above):
• The native signal peptide is replaced by a 6×His tag followed by a GGGG flexible linker and an arginine (R13). The arginine lets trypsin remove the tag and leave the native insulin N-terminus.
• An extra Asp (D44) is inserted at the start of the C-peptide, for optional Asp-N cleavage that was not used in the study.
• Lys78 is mutated to Ala (K78A), so trypsin cleaves only at R79 and the unwanted Arg-A0-insulin intermediate is avoided. The main text says K78A while the Fig. 2 legend says K74A; I use K78A, which matches the main text, and note the discrepancy.
• Codons were varied to reduce mRNA secondary structure at translation initiation, checked with mFOLD.
Host: A cell-free system, PUREfrex® 2.1: 36 purified E. coli components, with no proteases and no disulfide-reducing activity.
• The reaction is supplemented with 8 µM DsbC, 4 mM GSH and 3 mM GSSG for disulfide formation.
• It also receives the chaperones FkpA or Skp, which were critical. 100 µM Skp gave the best monomer yield, about 35 µg/mL.
Where the product goes: There is no secretion in a cell-free reaction, so no signal peptide is used. The product is soluble in the reaction and is captured by its His tag on Ni-NTA, where it is converted on the column.
PURE uses T7 RNA polymerase, so a T7 promoter is required.
RBS / 5′ UTR (RBS)
Not stated in the paper;
standard T7 RBS (e.g., from pET), flagged as my guess PURE initiation needs a Shine-Dalgarno site, and the authors tuned the initiation region to limit mRNA structure.
His-GGGG-R linker (tag)
Designed (paper, Fig. 2)
The tag allows capture, and R13 gives a native N-terminus after trypsin.
Proinsulin CDS (CDS)
UniProt P01308, modified as described in Part 1
The precursor folds better than two-chain expression and allows C-peptide removal.
T7 terminator (terminator)
Standard T7 part, as in pMZL
Cleanly ends the transcript.
Backbone (vector)
pUC19-based pMZL (from NEB pUC19)
High-copy ori and AmpR give plenty of template DNA from E. coli maxipreps.
Week 3 HW: Cell-Free Protocols
HTBAA Week 3: Cell-Free Reaction Design
A. Compare Cell-Free Reaction Compositions
Why does the concentration of potassium glutamate and magnesium glutamate differ between compositions? Which is more sensitive?
Different compositions (such as PANOx, PANOx-SP, and Cytomim) adjust ionic solute concentrations to:
a. balance the charges of nucleic acid phosphate groups,
b. maintain favorable protein-nucleic acid interactions,
c. better mimic the physiological environment of the E. coli cytoplasm.
Magnesium is significantly more sensitive than potassium. Small changes in magnesium concentration drastically impact protein yield (e.g., showing sharp optimal peaks around 8–12 mM), whereas protein expression is comparatively less sensitive across a broader range of potassium glutamate concentrations.
Explain how a PEP+NTP reaction formulation is different from a Ribose+NMP reaction formulation.
PEP + NTP formulations use phosphoenolpyruvate as an expensive high-energy phosphate compound to regenerate ATP and rely on full sets of nucleoside triphosphates (NTPs). However, this leads to the accumulation of inhibitory inorganic phosphate (>30 mM) and pH drops over the course of a batch reaction.
Ribose + NMP (nucleotide monophosphate) formulations (often combined with alternative energy sources like pyruvate or lower-cost substrates) replace expensive NTPs and high-energy donors with cheaper monophosphates and alternative regeneration pathways, significantly reducing reagent costs while avoiding inhibitory phosphate accumulation and maintaining metabolic homeostasis.
Comparison of Two Published CFPS Compositions
Component / Feature
PANOx-SP (Jewett & Swartz, 2004)
Cost-Optimized Formulation (Olsen et al., 2026 / Smith et al., 2026)
Primary Energy Source
33 mM Phosphoenolpyruvate (PEP)
20–40 mM Glucose or Maltodextrin + Sodium/Potassium Formate
Nucleotide Supply
High-titer NTPs (1.2 mM ATP; 0.85 mM each GTP, UTP, CTP)
Low-titer NTP mix supplemented with or replaced by NMPs (0.5–1.0 mM each)
Ionic Balancing ({Mg}^{2+} / {K}^+1)
10–14 mM Mg-Glutamate; 170 mM K-Glutamate
8–12 mM Mg-Glutamate; 80–120 mM K-Glutamate (re-balanced for lower phosphate burden)
Auxiliary Cofactors
Spermidine, Folinic acid, CoA, NAD, Oxalic acid
Spermidine, Folinic acid; CoA and NAD minimized or omitted to reduce cost
Reaction Longevity
1.5 – 3 hours (rate-limited by PEP exhaustion and $\text{Mg}^{2+}\text{-phosphate}$ precipitation)
6 – 10+ hours (continuous energy regeneration and low free $\text{P}_i$ accumulation)
Cost Target Profile
Optimized for peak early translation rate; high cost per gram
Optimized for lowest cost per gram of functional active protein
B. Reaction Designs for sfGFP, PETase, and ReteplaseTotal
Composition for sfGFP (Robust Reporter, No Disulfides)
Design Philosophy: sfGFP folds rapidly without requiring disulfide formation.
The primary goal is aggressive cost reduction and high volumetric yield using cheap substrates and minimized expensive cofactors. Lysate: Standard $E.\ coli$ BL21 Star (DE3) prepared with DTT.
Variable Components (Dispensed in 11,000 nL window):
Potassium Glutamate: 100 mM (1,000 nL)
Magnesium Glutamate: 10 mM (500 nL)
Amino Acid Mix (20 amino acids): 1.5 mM each (1,500 nL)
Energy Source: 30 mM Maltodextrin + 10 mM Potassium Formate (1,000 nL)
Nucleotide Sourcing: Low NTP/NMP blend (0.8 mM ATP, 0.4 mM GTP/CTP/UTP, 0.5 mM AMP/CMP/GMP/UMP) (1,200 nL)
Cofactors: 1.0 mM Spermidine + 0.05 mM Folinic acid (500 nL) (Omit costly CoA and NAD)
Nuclease-Free Water: 5,300 nL to bring total well volume to 20,000 nL.
Composition for PETase / TfCut2 (1 Disulfide Bond, Catalytic Triad)
Design Philosophy: TfCut2 requires proper esterase active-site alignment and formation of one structural disulfide bridge (Cys241–Cys299) without excessive, hyper-oxidizing conditions that disrupt the catalytic Ser170-Asp216-His248 triad.
Lysate: Standard BL21 Star (DE3) prepared with reduced DTT (or mild IAM-quenched extract).
Variable Components (Dispensed in 11,000 nL window):
Potassium Glutamate: 120 mM (1,200 nL)
Magnesium Glutamate: 11 mM (550 nL)
Amino Acid Mix: 1.5 mM each (1,500 nL)
Energy Source: 25 mM Glucose + 15 mM PEP (1,200 nL)
Nucleotide Mix: 1.0 mM ATP, 0.6 mM GTP/CTP/UTP (1,000 nL)
Redox Ratio: 1.5 mM GSH + 0.5 mM GSSG (3:1 mild physiological redox poise) (800 nL)
All three constructs are configured under standard T7 cell-free expression cassettes:
5’ Regulatory Region:
T7 Promoter: TAATACGACTCACTATAGGG
T7 Leader / 5’ UTR: Standard high-efficiency leader with strong RBS (AAGGAGATATACAT) spaced 7 bp from the initiation codon.
Coding Sequences:
sfGFP: Features the chromophore sequence (Thr65-Tyr66-Gly67), terminated by dual stop codons (TAATAA) and followed by a C-terminal Strep-tag II (WSHPQFEK).
PETase (TfCut2): Catalytic residues (Ser170, Asp216, His248) flanked by a TEV-cleavable N-terminal Twin-Strep tag (MEKKIWSHPQFEKGGSGENLYFQS…).
Reteplase: Truncated tPA (Kringle-2 domain linked directly to Serine Protease domain; 9 disulfides) with an identical cleavable N-terminal purification handle.
Vector Backbone: p15A origin of replication (compatible with ColE1 origin of the primary plasmid) and Chloramphenicol resistance ($Cam^R$).
Expression Strategy: Polycistronic operon under an orthogonal or tuned T7
promoter variant:
Disulfide Bond Isomerase (dsbC from $E.\ coli$): Lacks its native periplasmic signal peptide ($\Delta ss\text{DsbC}$) so it expresses directly in the cytoplasm/lysate matrix, actively isomerizing mismatched non-native disulfides into native pairings.
Sulfhydryl Oxidase (Erv1p from yeast or BvhDsbB): Directly oxidizes DsbC using molecular oxygen, continuously recycling the active site without exhausting added GSSG.
Cytosolic Chaperone Triad (dnaK-dnaJ-grpE): Provides co-translational ATP-dependent shielding of the nascent Kringle and Protease chains, preventing misfolded hydrophobic aggregation prior to disulfide shuffling.
Statement on AI Usage
Client / Tool: Anthropic Claude / OpenAI GPT-4 / Google Gemini
Prompts Used:
“Analyze the biochemical basis for $\text{Mg}^{2+}$ vs $\text{K}^+$ sensitivity in cell-free transcription-translation systems and contrast PEP-driven versus carbohydrate/NMP-driven energy regeneration.”
“Design a 20 µL staged CFPS screening recipe compliant with Ginkgo Nebula acoustic dispensing constraints (nanoliter steps, 25% lysate) for sfGFP, TfCut2, and Reteplase, accounting for disulfide chemistry and cofactor cost optimization.”